Related Experiment Video
Updated: Jun 6, 2026
Method to Visualize and Analyze Membrane Interacting Proteins by Transmission Electron Microscopy
Published on: March 5, 2017
Stability and membrane orientation of the fukutin transmembrane domain: a combined multiscale molecular dynamics and
Daniel A Holdbrook1, Yuk Ming Leung, Thomas J Piggot
1School of Chemistry, University of Southampton, Highfield, Southampton SO17 1BJ, UK.

The N-terminal domain of fukutin-I has been implicated in the localization of the protein in the endoplasmic reticulum and Golgi Apparatus. It has been proposed to mediate this through its interaction with the thinner lipid bilayers found in these compartments. Here we have employed multiscale molecular dynamics simulations and circular dichroism spectroscopy to explore the structure, stability, and orientation of the short 36-residue N-terminus of fukutin-I (FK1TMD) in lipids with differing tail lengths. Our results show that FK1TMD adopts a stable helical conformation in phosphatidylcholine lipids when oriented with its principal axis perpendicular to the bilayer plane. The stability of the helix is largely insensitive to the lipid tail length, preventing hydrophobic mismatch by virtue of its mobility and ability to tilt within the lipid bilayers. This suggests that changes in FK1TMD tilt in response to bilayer properties may be implicated in the regulation of its trafficking. Coarse-grained simulations of the complex Golgi membrane suggest the N-terminal domain may induce the formation of microdomains in the surrounding membrane through its preferential interaction with 1,2-dipalmitoyl-sn-glycero-3-phosphatidylinositol 4,5-bisphosphate lipids.
The N-terminal domain of fukutin-I has been implicated in the localization of the protein in the endoplasmic reticulum and Golgi Apparatus. It has been proposed to mediate this through its interaction with the thinner lipid bilayers found in these compartments. Here we have employed multiscale molecular dynamics simulations and circular dichroism spectroscopy to explore the structure, stability, and orientation of the short 36-residue N-terminus of fukutin-I (FK1TMD) in lipids with differing tail lengths. Our results show that FK1TMD adopts a stable helical conformation in phosphatidylcholine lipids when oriented with its principal axis perpendicular to the bilayer plane. The stability of the helix is largely insensitive to the lipid tail length, preventing hydrophobic mismatch by virtue of its mobility and ability to tilt within the lipid bilayers. This suggests that changes in FK1TMD tilt in response to bilayer properties may be implicated in the regulation of its trafficking. Coarse-grained simulations of the complex Golgi membrane suggest the N-terminal domain may induce the formation of microdomains in the surrounding membrane through its preferential interaction with 1,2-dipalmitoyl-sn-glycero-3-phosphatidylinositol 4,5-bisphosphate lipids.
Related Concept Videos
 01:26
Membrane Fluidity
Mosaic nature of the membrane
The mosaic characteristic of the membrane helps the plasma membrane remain fluid. The integral proteins and lipids exist as separate but loosely-attached molecules in the membrane. The membrane is a relatively...
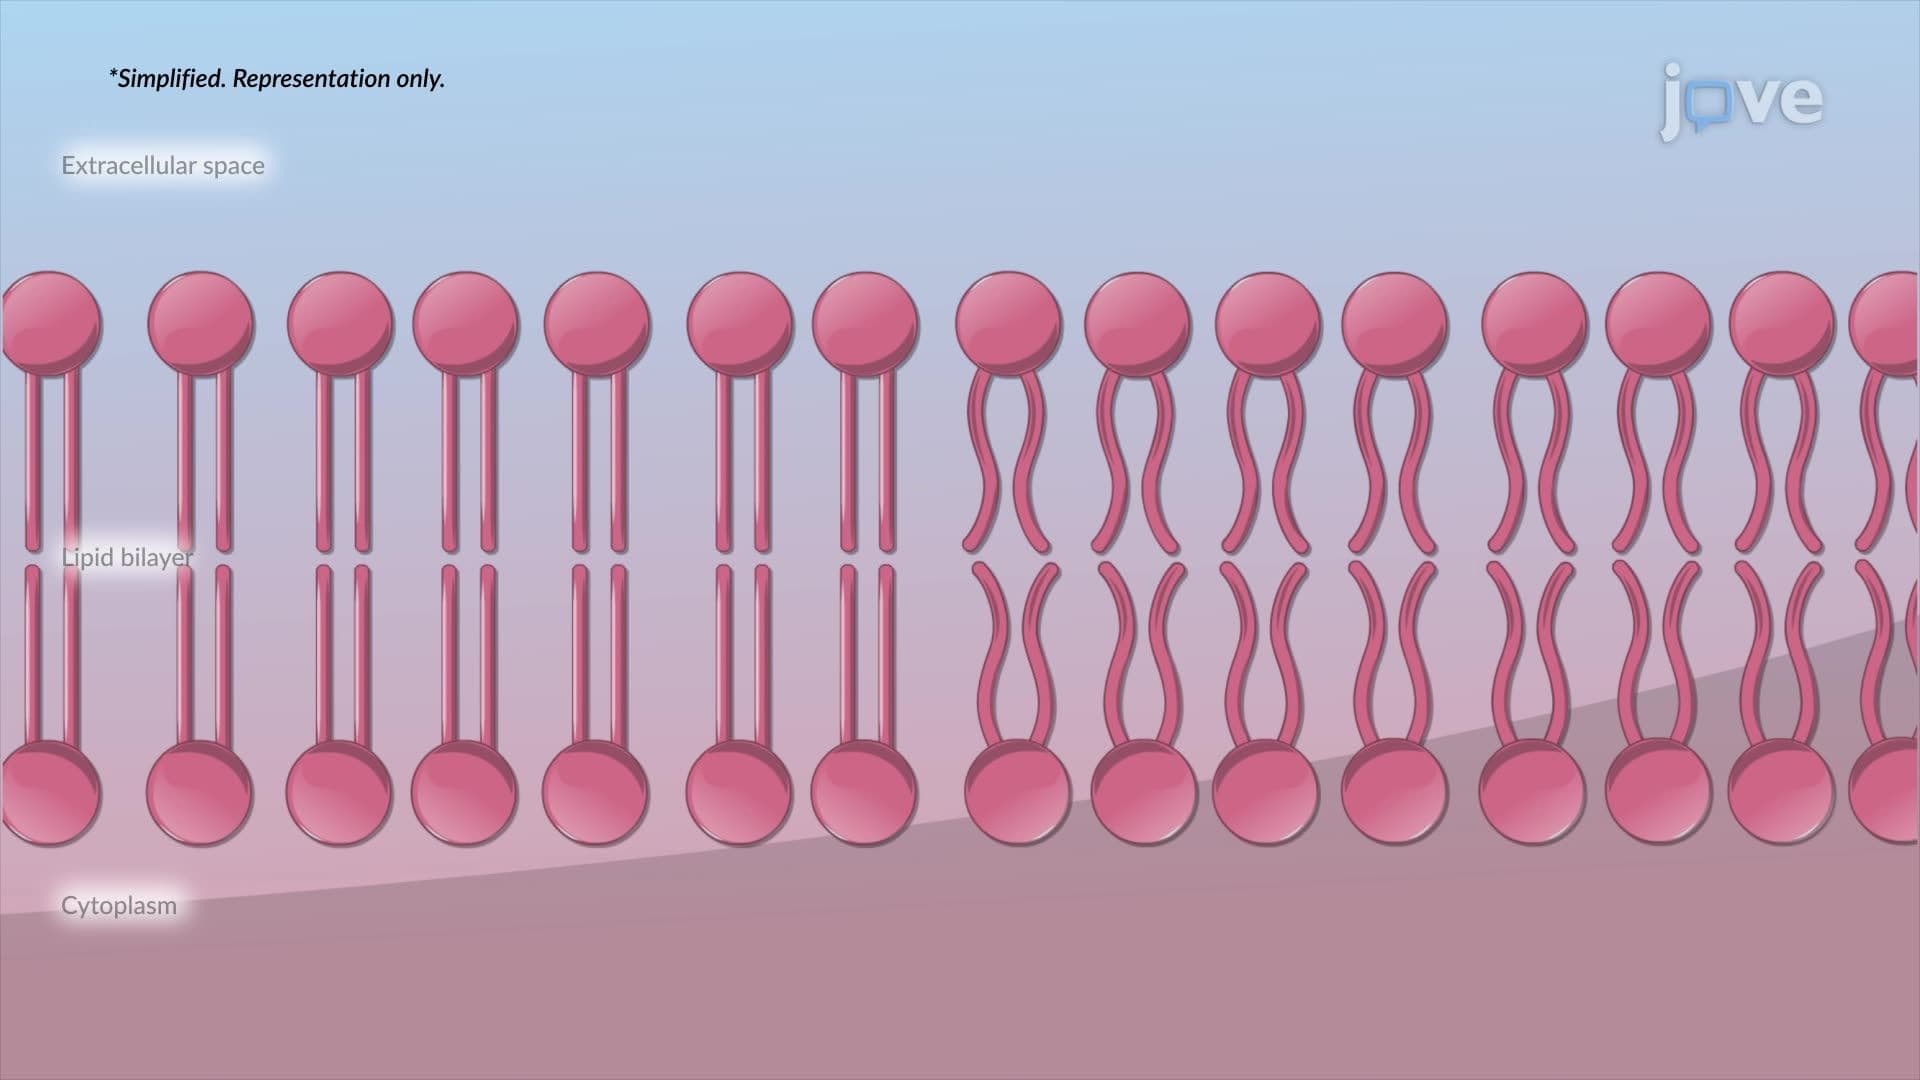 01:23
Membrane Fluidity
 00:59
Mechanisms of Membrane Domain Formation
Another mechanism for membrane domain formation involves membrane proteins interacting with cytoskeletal...
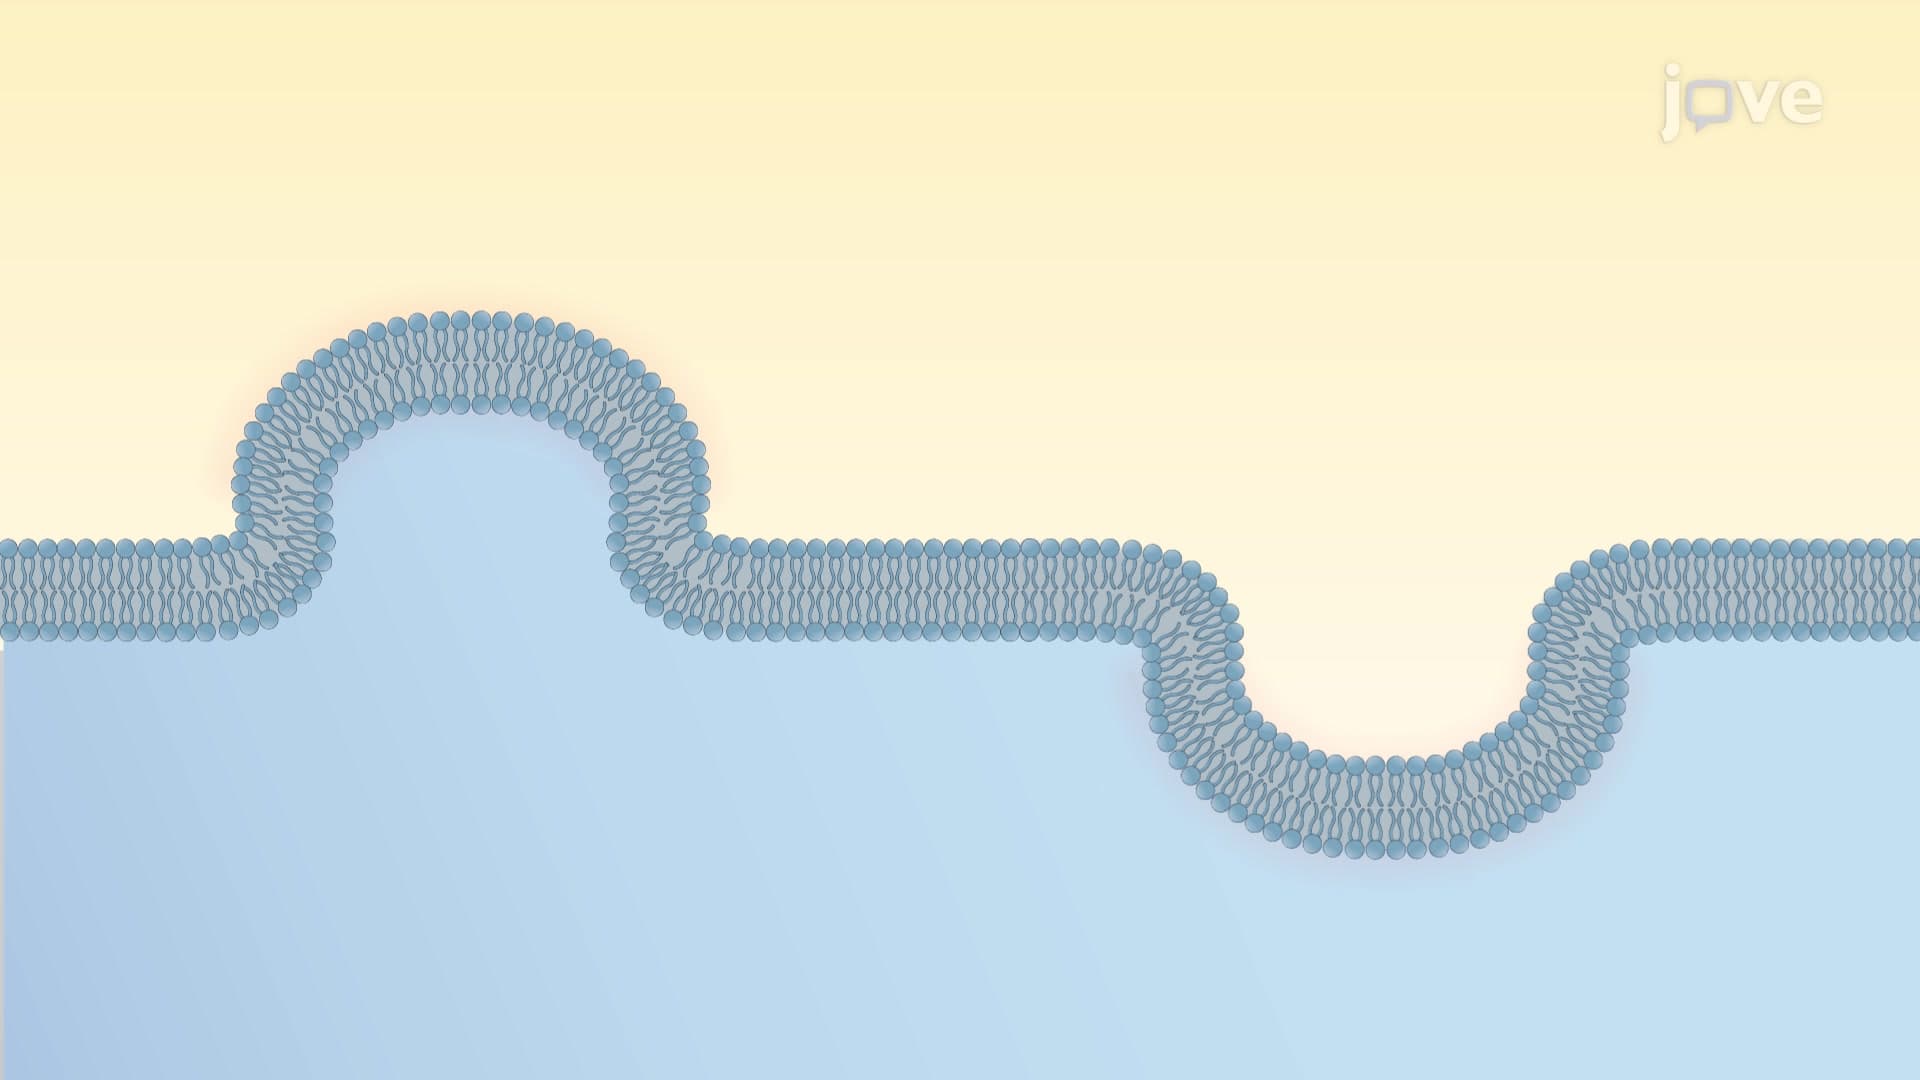 01:15
Mechanisms of Membrane-bending
Membrane bending can happen due to intrinsic changes in lipid composition or extrinsic association with different proteins. The proteins involved...