Related Experiment Video
Updated: Jun 5, 2026

Presynapse Formation Assay Using Presynapse Organizer Beads and “Neuron Ball” Culture
Published on: August 2, 2019
RIM proteins activate vesicle priming by reversing autoinhibitory homodimerization of Munc13
Lunbin Deng1, Pascal S Kaeser, Wei Xu
1Department of Molecular and Cellular Physiology, Stanford University, Lorry Lokey Building, 265 Campus Drive, Stanford, CA 94305-5453, USA.

Abstract:
At a synapse, the presynaptic active zone mediates synaptic vesicle exocytosis. RIM proteins are active zone scaffolding molecules that--among others--mediate vesicle priming and directly or indirectly interact with most other essential presynaptic proteins. In particular, the Zn²+ finger domain of RIMs binds to the C₂A domain of the priming factor Munc13, which forms a homodimer in the absence of RIM but a heterodimer with it. Here, we show that RIMs mediate vesicle priming not by coupling Munc13 to other active zone proteins as thought but by directly activating Munc13. Specifically, we found that the isolated Zn²+ finger domain of RIMs autonomously promoted vesicle priming by binding to Munc13, thereby relieving Munc13 homodimerization. Strikingly, constitutively monomeric mutants of Munc13 rescued priming in RIM-deficient synapses, whereas wild-type Munc13 did not. Both mutant and wild-type Munc13, however, rescued priming in Munc13-deficient synapses. Thus, homodimerization of Munc13 inhibits its priming function, and RIMs activate priming by disrupting Munc13 homodimerization.
Related Concept Videos
 01:14
Rab Proteins
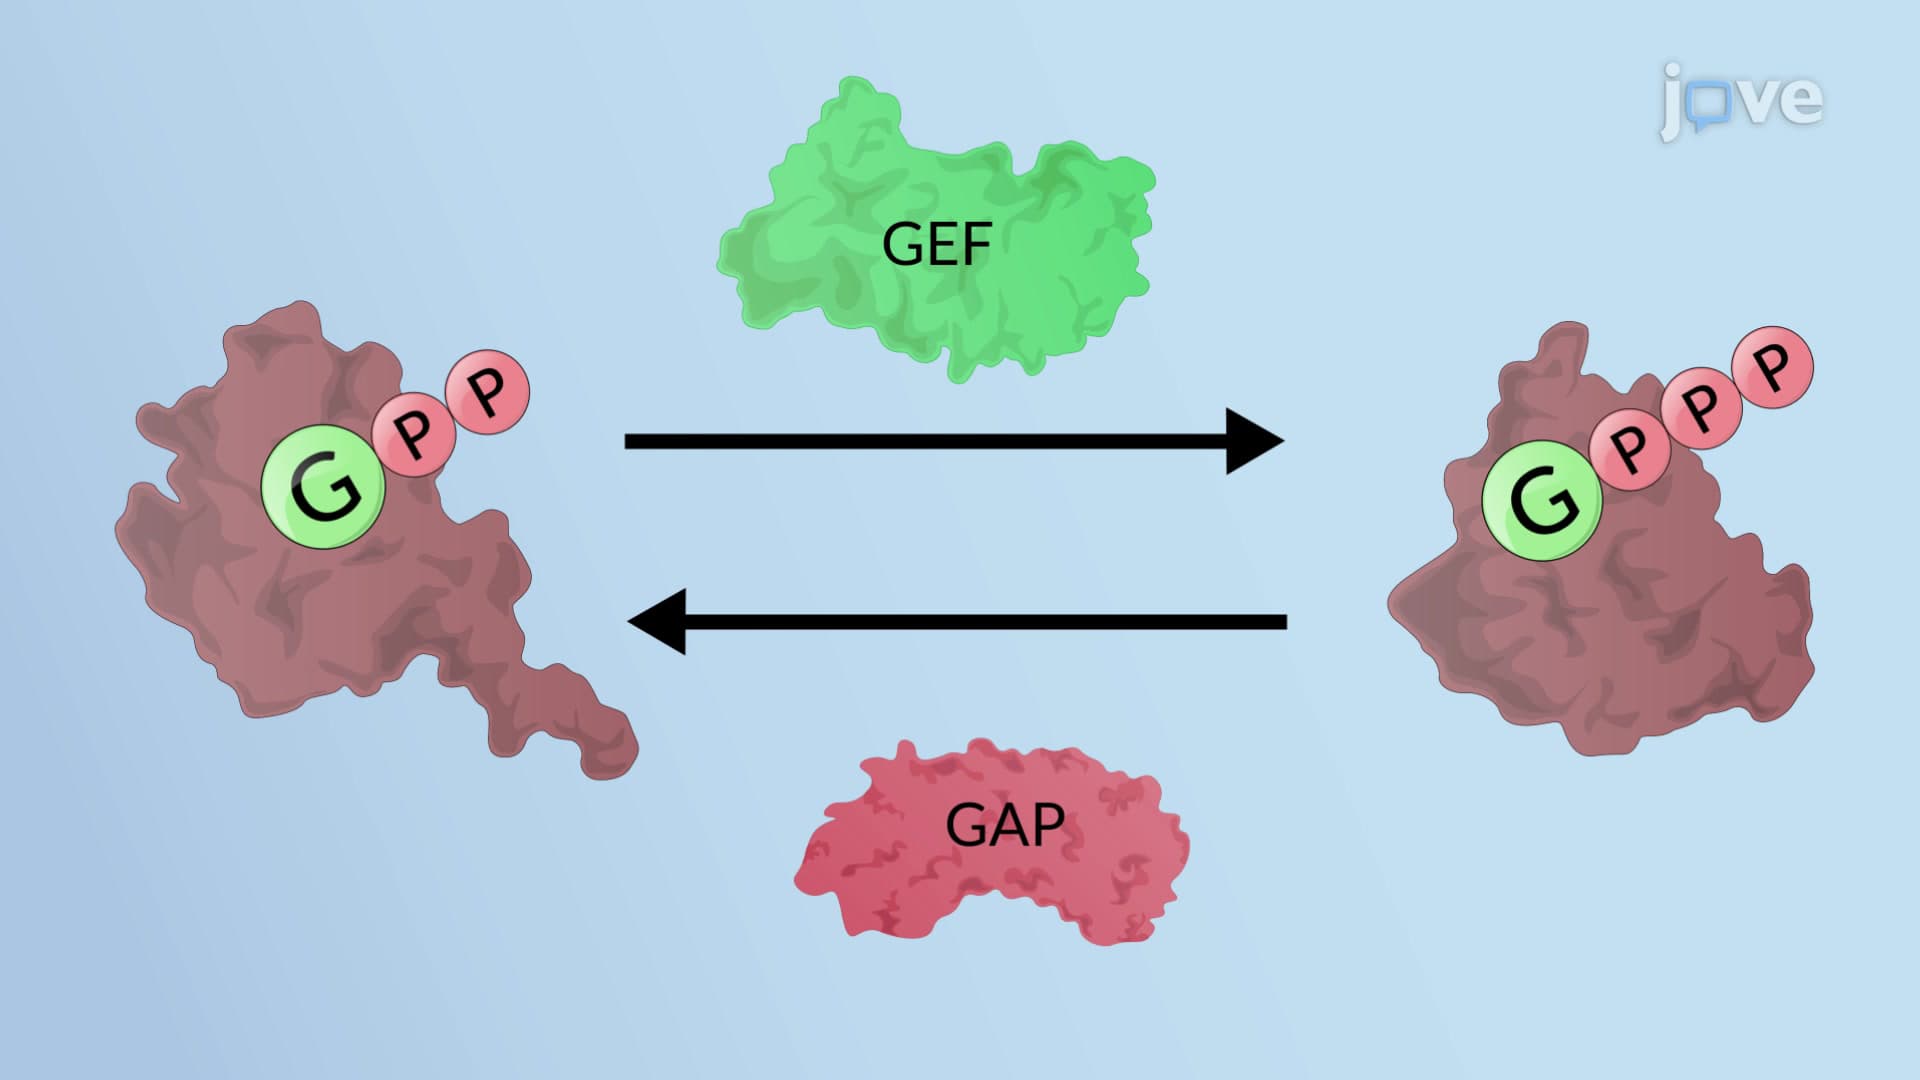
Rab proteins switch between a cytosolic, GDP-bound inactive state and a membrane-anchored, GTP-bound active state. By themselves, Rabs show slow rates of GDP/GTP exchange and GTP hydrolysis. Thus, Rab proteins are considered...
 01:32
Pinching-off of Coated Vesicles
 01:38
Intralumenal Vesicles and Multivesicular Bodies
 01:37
The Unfolded Protein Response
 01:26
Fusion of Secretory Vesicles with the Plasma Membrane
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
 01:31
Regulation of the Unfolded Protein Response