Related Experiment Video
Updated: Jun 3, 2026

Targeting Cysteine Thiols for in Vitro Site-specific Glycosylation of Recombinant Proteins
Published on: October 4, 2017
A cytosolic STIM2 preprotein created by signal peptide inefficiency activates ORAI1 in a store-independent manner
Sarah J L Graham1, Marie A Dziadek, Lorna S Johnstone
1School of Biological Sciences, University of Auckland, Auckland, New Zealand.

Abstract:
Calcium (Ca(2+)) influx through the plasma membrane store-operated Ca(2+) channel ORAI1 is controlled by Ca(2+) sensors of the stromal interaction molecule (STIM) family. STIM1 responds to endoplasmic reticulum (ER) Ca(2+) store depletion by redistributing and activating ORAI1 from regions of the ER juxtaposed to the plasma membrane. Unlike STIM1, STIM2 can regulate ORAI1 in a store-dependent and store-independent manner, but the mechanism by which this is achieved is unknown. Here we find that STIM2 is translated from a highly conserved methionine residue and is directed to the ER by an incredibly long 101-amino acid signal peptide. We find that although the majority of the total STIM2 population resides on the ER membrane, a second population escapes ER targeting to accumulate as a full-length preprotein in the cytosol, signal peptide intact. Unlike STIM2, preSTIM2 localizes to the inner leaflet of the plasma membrane where it interacts with ORAI1 to regulate basal Ca(2+) concentration and Ca(2+)-dependent gene transcription in a store-independent manner. Furthermore, a third protein comprising a fragment of the STIM2 signal peptide is released from the ER membrane into the cytosol where it regulates gene transcription in a Ca(2+)-independent manner. This study establishes a new model for STIM2-mediated regulation of ORAI1 in which two distinct proteins, STIM2 and preSTIM2, control store-dependent and store-independent modes of ORAI1 activation.
More Related Videos
 10:45
Isolation of Human Myoblasts, Assessment of Myogenic Differentiation, and Store-operated Calcium Entry Measurement
Published on: July 26, 2017
 14:18
Fluorescence-based Measurement of Store-operated Calcium Entry in Live Cells: from Cultured Cancer Cell to Skeletal Muscle Fiber
Published on: February 13, 2012
Related Concept Videos
 01:15
Amplifying Signals via Second Messengers
 01:34
Directing Proteins to the Rough Endoplasmic Reticulum
 01:26
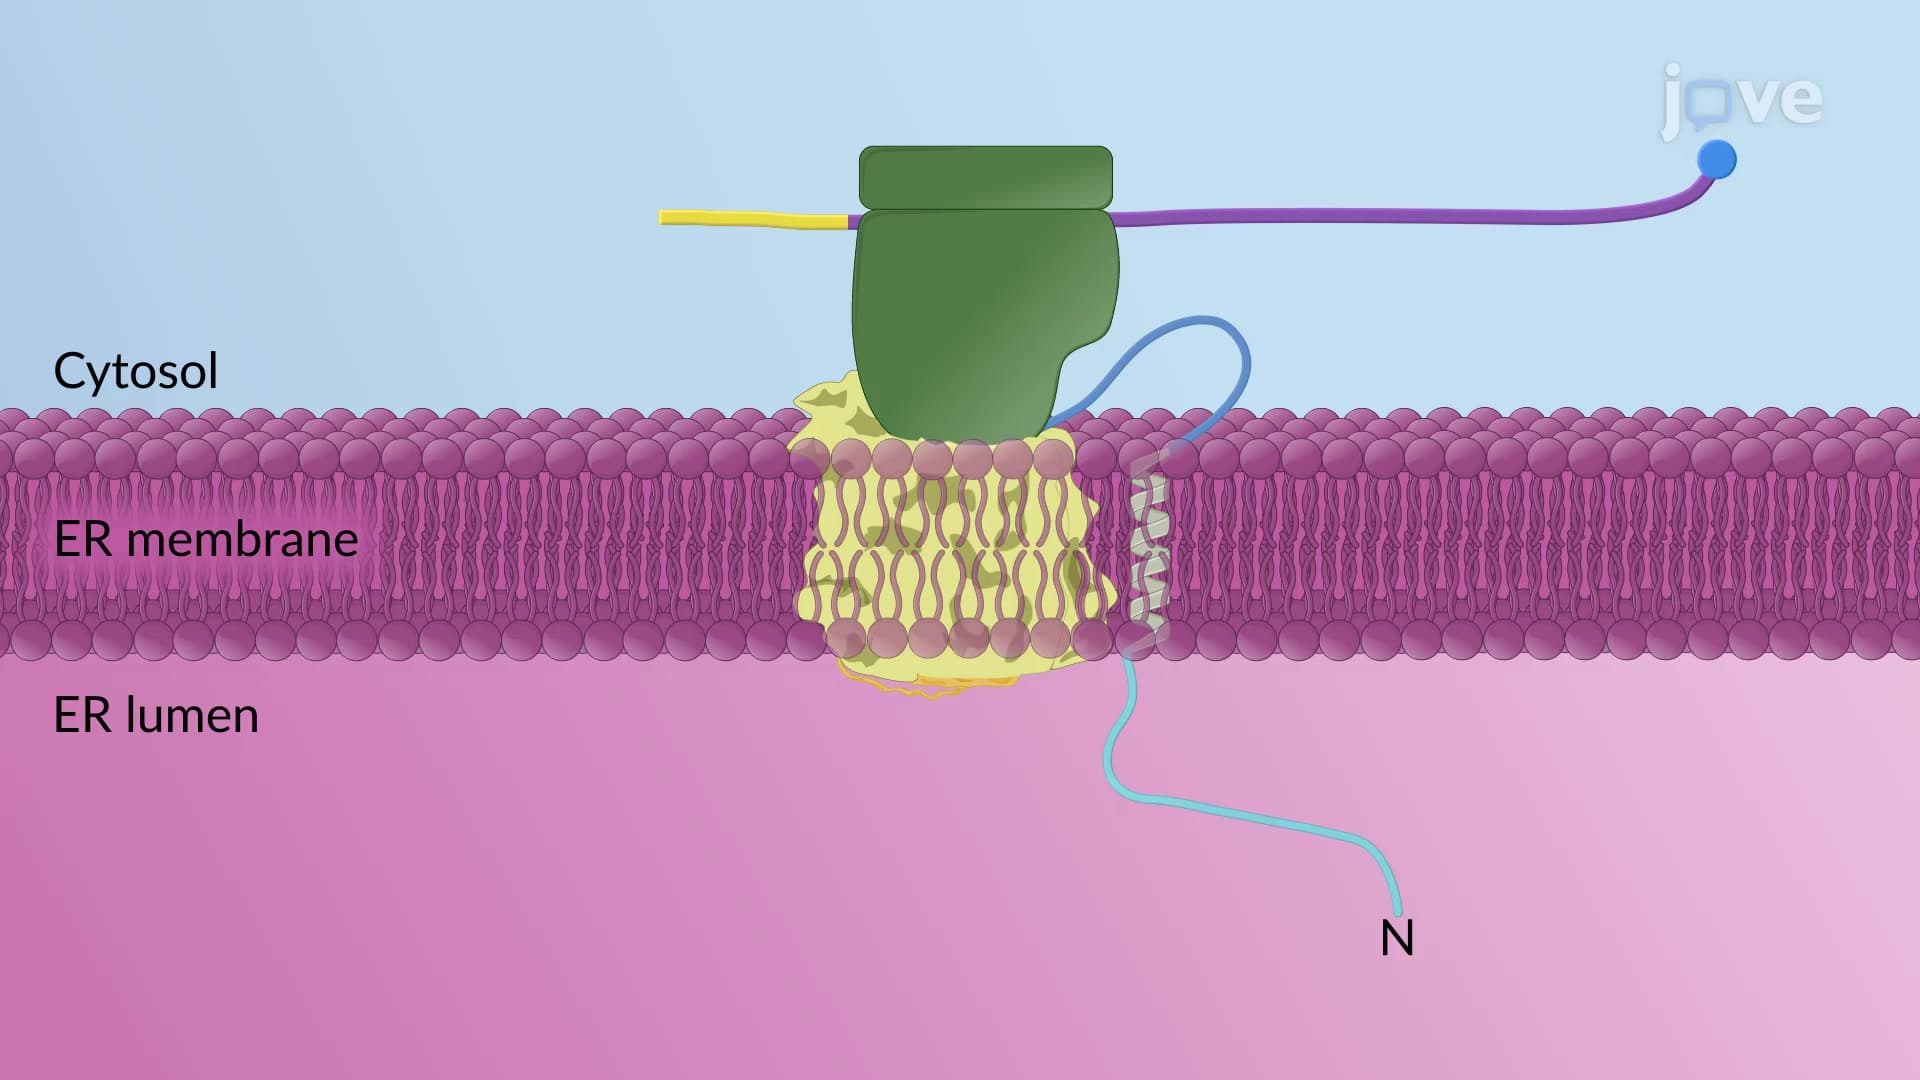
Insertion of Single-pass Transmembrane Proteins in the RER
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
 01:11
IP3/DAG Signaling Pathway
 01:16
Calmodulin-dependent Signaling
The Ca2+-CaM complex does not have enzymatic activity by itself. Instead, the complex binds downstream target proteins, including membrane proteins or enzymes,...
 01:31
Regulation of the Unfolded Protein Response