
Inositol 1, 4, 5-trisphosphate receptor interacts with the SNARE domain of syntaxin 1B
Sayaka Tanaka1, Hiroyuki Kabayama, Masahiro Enomoto
1Department of Neurosurgery, Graduate School of Medicine, University of Tokyo, 7-3-1 Hongo, Bunkyo-ku, Tokyo, 113-8655, Japan.

Abstract:
Inositol 1, 4, 5-trisphosphate receptors (IP(3)Rs) are intracellular ligand-gated Ca(2+) channels that mediate Ca(2+) release from the endoplasmic reticulum (ER) into the cytosol and function in diverse cellular processes including fertilization, muscle contraction, apoptosis, secretion, and synaptic plasticity. The Ca(2+) release activity of IP(3)Rs is tightly regulated by many factors including IP(3)R-binding proteins. We show that IP(3)Rs interact with syntaxin 1 (Syx1), a membrane trafficking protein that regulates various plasma-membrane ion channels including N-, P/Q, and L-type voltage-gated Ca(2+) channels, voltage-gated potassium channels, and an epithelial sodium channel. We found that a SNARE-domain of Syx1B, one of the two Syx1 isoforms, directly interacted with the type1 IP(3)R (IP(3)R1) internal coupling domain, a known modulator for channel opening. These results indicate that Syx1B is an IP(3)R-interacting protein and that its interaction may play a crucial role in regulating the channel activity of IP(3)Rs in Syx1B-expressing cells.
Related Concept Videos
 01:42
Phosphoinositides and PIPs
Different phosphoinositides are synthesized and recruited on the cytosolic face of the plasma membrane. The localization of specific phosphoinositides concentrated in separate membrane...
 01:43
SNAREs and Membrane Fusion
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
 01:26
Fusion of Secretory Vesicles with the Plasma Membrane
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
 01:11
IP3/DAG Signaling Pathway
 01:28
Protein Translocation Machinery on the ER Membrane
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the translocon complex.
 01:19
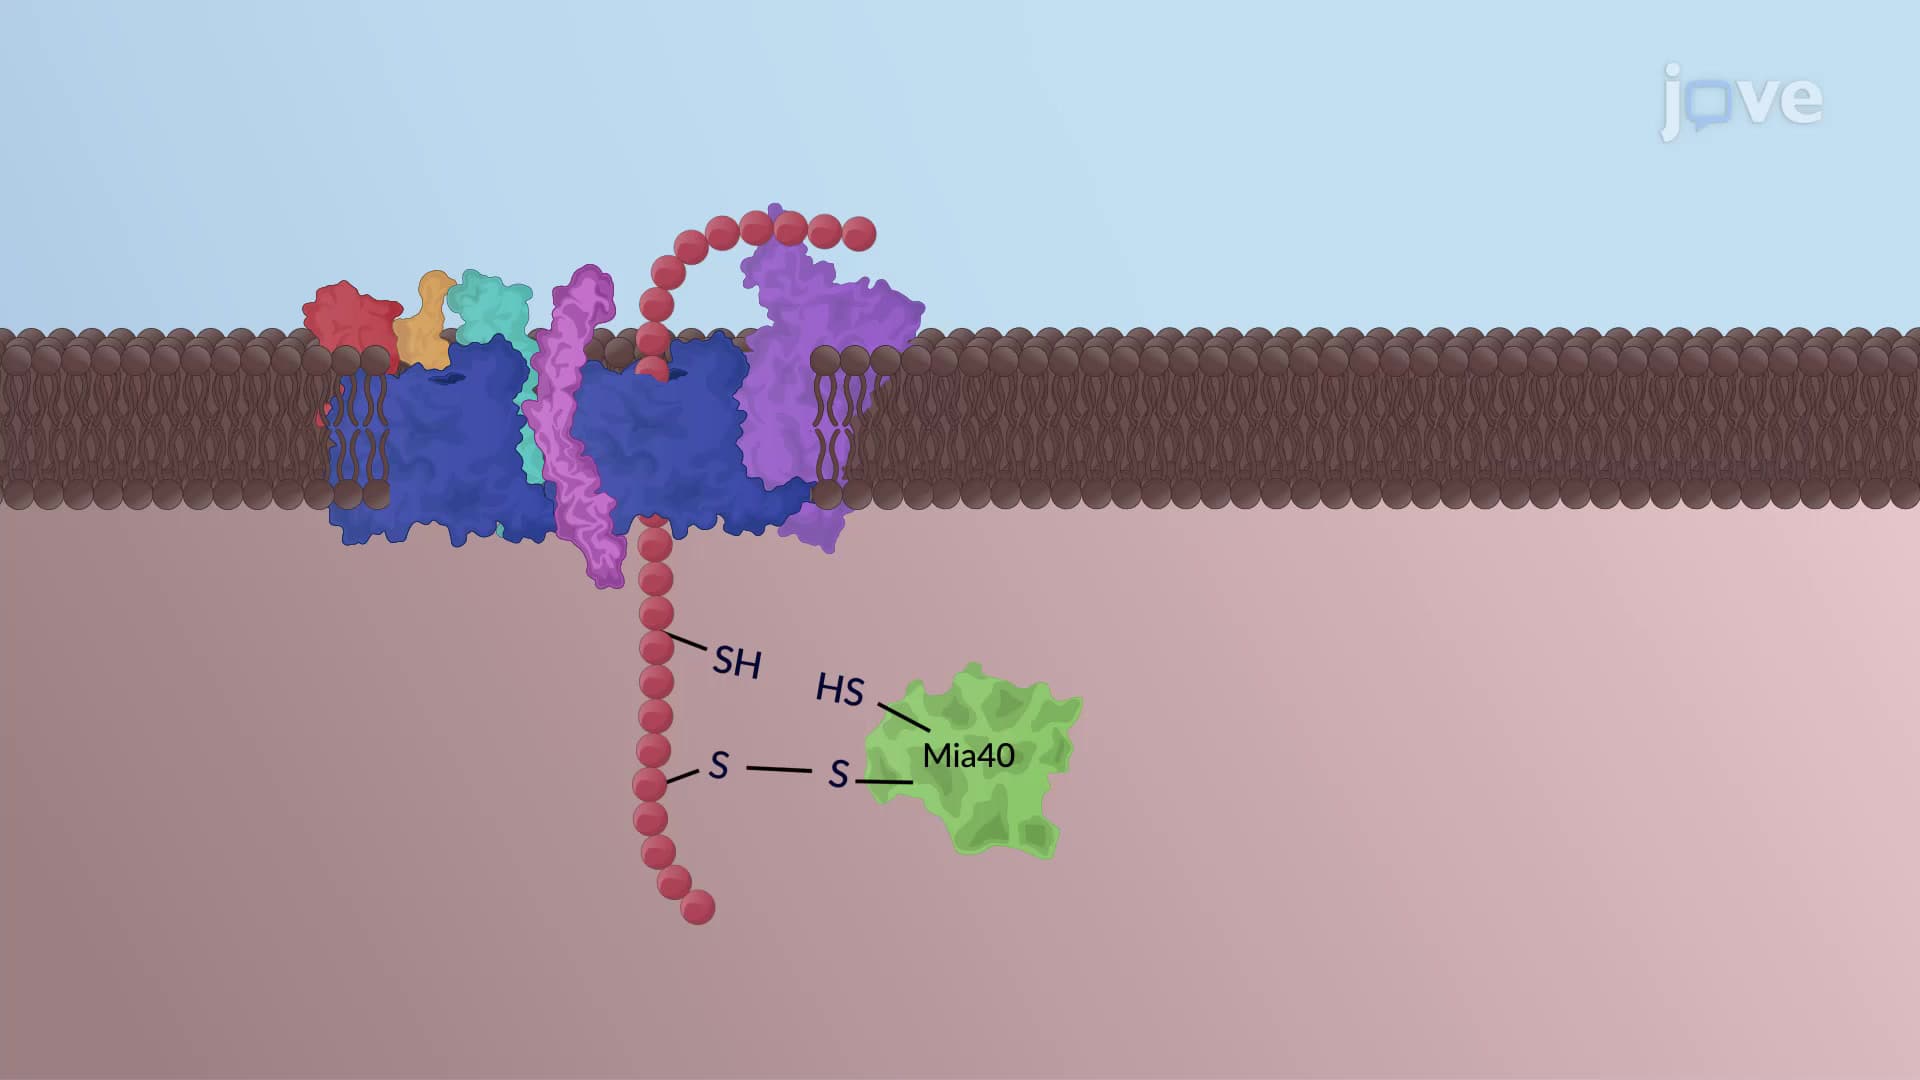
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...