Related Experiment Video
Updated: Jun 3, 2026

Method to Visualize and Analyze Membrane Interacting Proteins by Transmission Electron Microscopy
Published on: March 5, 2017
Two modes of interaction between the membrane-embedded TARP stargazin's C-terminal domain and the bilayer visualized
Matthew F Roberts1, David W Taylor, Vinzenz M Unger
1Department of Molecular Biophysics and Biochemistry, Yale University School of Medicine, New Haven, CT 06510, USA.

Abstract:
Glutamate-mediated neurotransmission through ligand-gated, ionotropic glutamate receptors is the main form of excitatory neurotransmission in the vertebrate central nervous system where it plays central roles in learning, memory and a variety of disorders. Acting as auxiliary subunits, transmembrane α-amino-3-hydroxy-5-methyl-4-isoxazole propionic acid receptor (AMPAR) regulatory proteins (TARPs) are essential regulators for glutamate-mediated neurotransmission in the central nervous system. Here, we report the first electron crystallographic reconstructions of full-length mouse stargazin (γ-2) at ∼20Å resolution in a membrane bilayer environment. Formation of ordered arrays required anionic lipids and was modulated by cholesterol and monovalent cations. Projection structures revealed that the C-termini of stargazin monomers closely interacted with the bilayer surface in an extended conformation that placed the C-terminal PDZ-binding motif ∼100Å away from the transmembrane domain and in close proximity to a membrane re-entrant region. The C-termini interaction with the bilayer was modulated by the ionic strength of the solution and overall protein secondary structure increased when membrane-bound. Our data suggest that stargazin interactions with and within the membrane play significant roles in TARP structure and directly visualize TARP functional mechanisms essential for AMPAR trafficking and clustering.
Related Concept Videos
 01:09
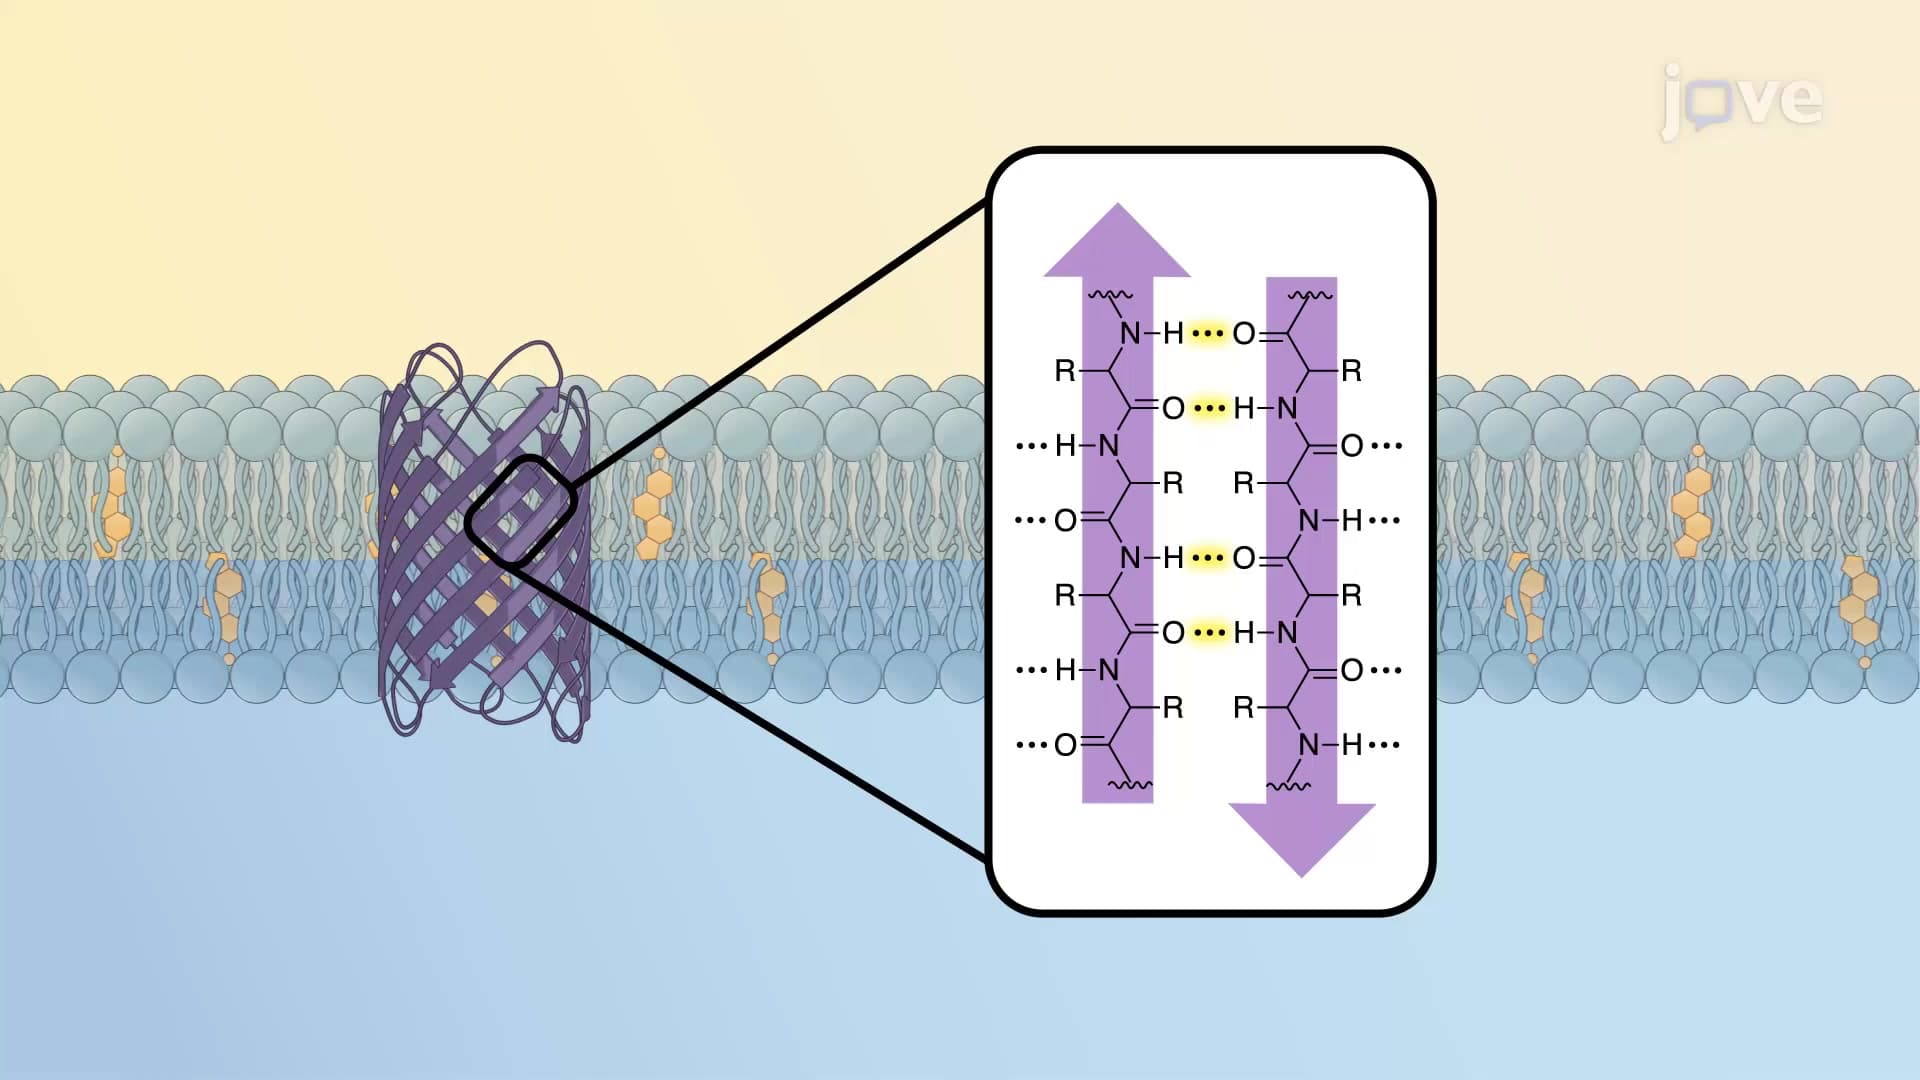
Multi-pass Transmembrane Proteins and β-barrels
α-Helix containing multi-pass transmembrane proteins
Multi-pass transmembrane proteins such as G-protein-linked receptors (GPCRs) and...
 01:19
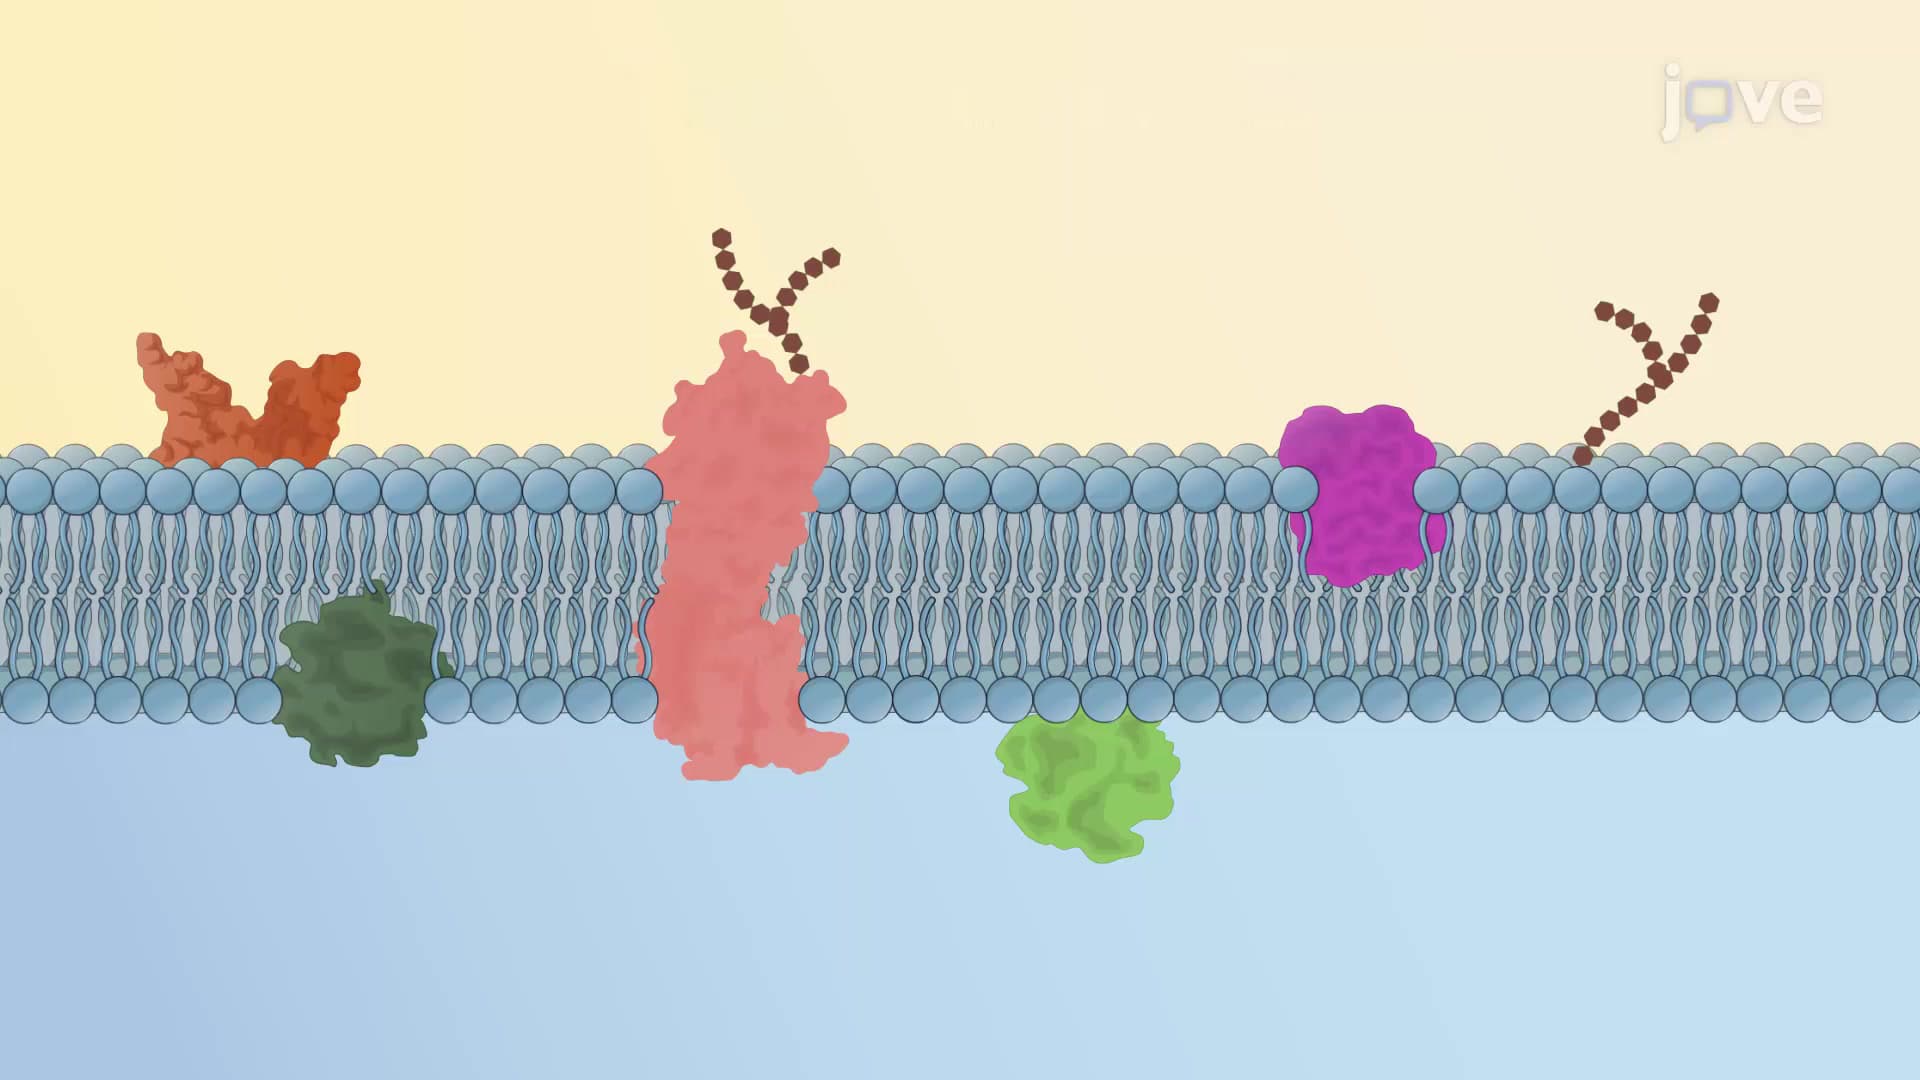
Fluid Mosaic Model
 00:59
Mechanisms of Membrane Domain Formation
Another mechanism for membrane domain formation involves membrane proteins interacting with cytoskeletal...
 01:43
SNAREs and Membrane Fusion
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
 01:45
Tail-anchoring of Proteins in the ER Membrane
 01:45
Vesicular Tubular Clusters
With the help of motor proteins such...