Staying in touch: the molecular era of organelle contact sites

Yael Elbaz1, Maya Schuldiner

  • 1Department of Molecular Genetics, Weizmann Institute of Science, Rehovot 76100, Israel.

Related Concept Videos

Contact-dependent Signaling01:19

Contact-dependent Signaling

Contact-dependent signaling, as the name suggests, requires that communicating cells be in direct contact with each other. This is achieved either through receptor-ligand interactions or by specialized cytoplasmic channels that allow the flow of small molecules between cells. In animal cells, channels called gap junctions facilitate contact-dependent signaling in certain tissues, whereas, plasmodesmata perform a similar function in plants.
Gap Junctions
In animal cells, gap junctions are formed...
Attachment of Sister Chromatids02:57

Attachment of Sister Chromatids

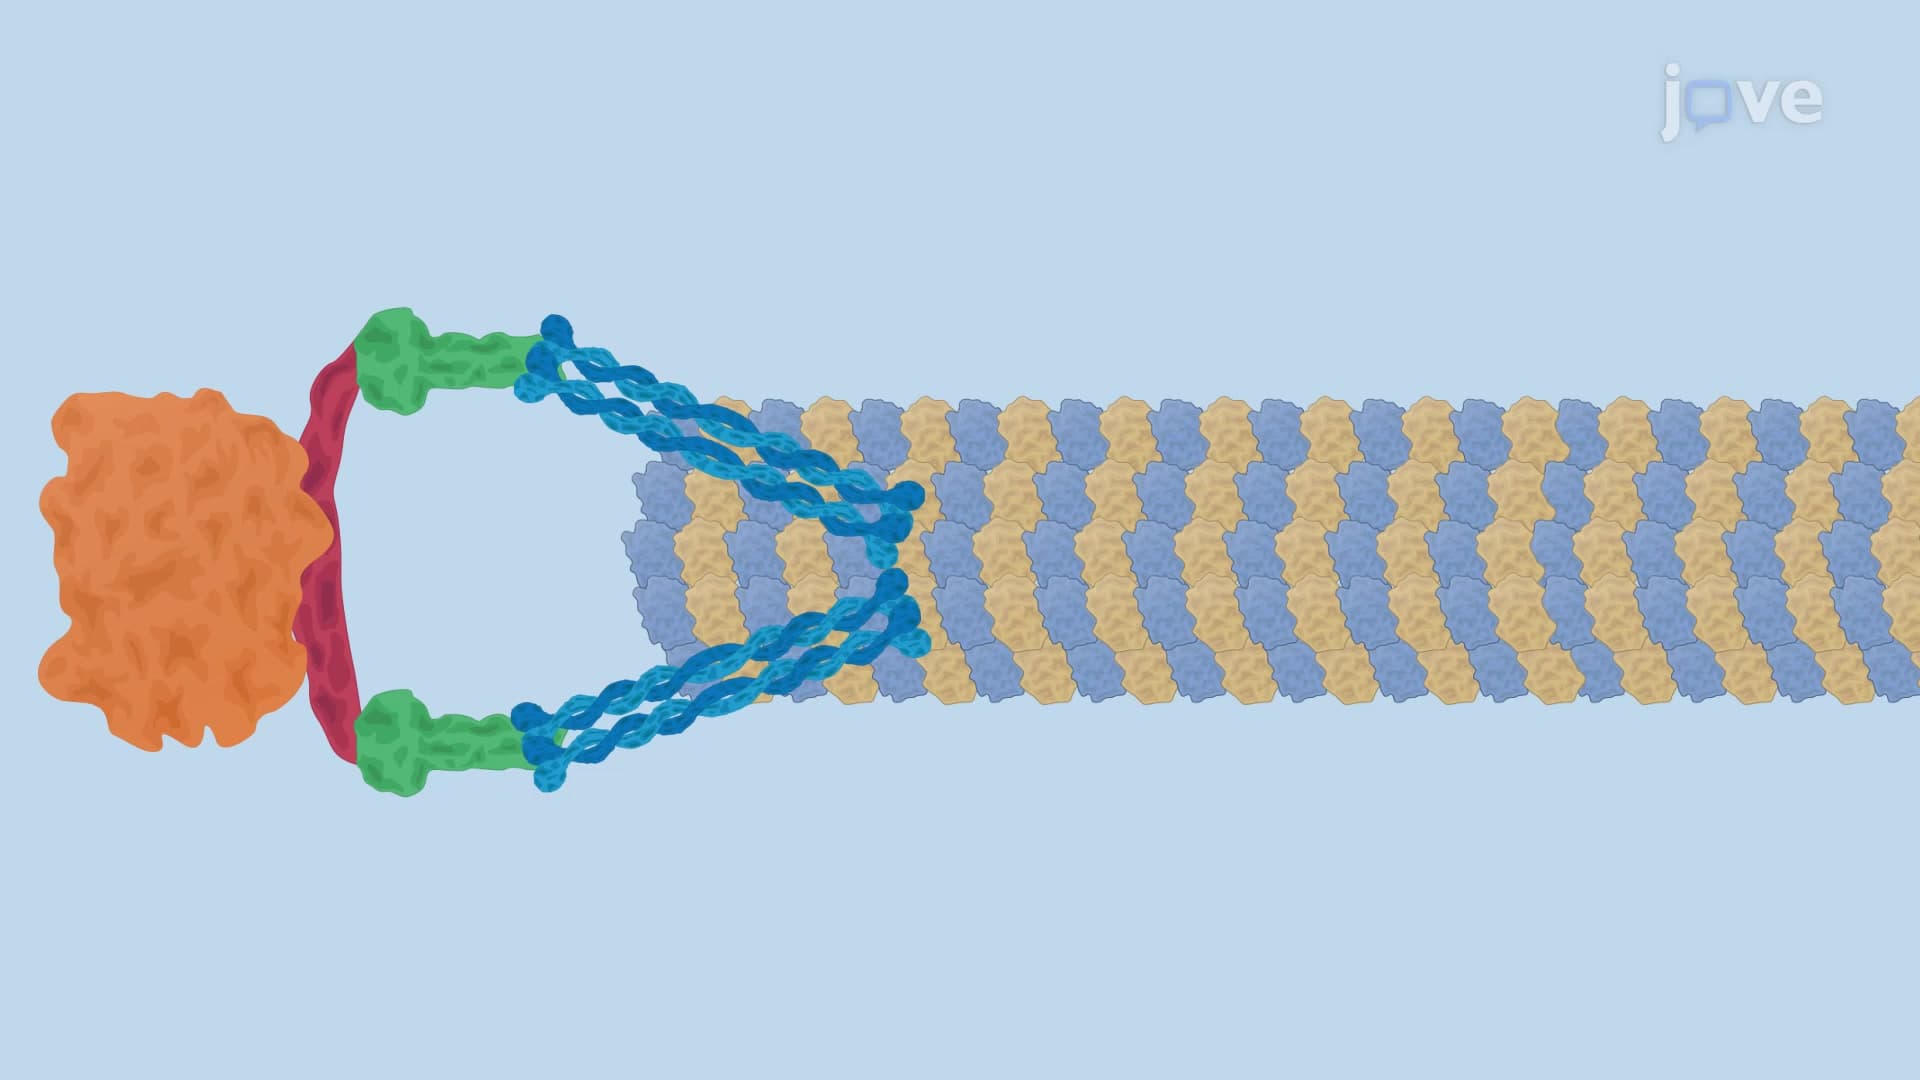
As cells progress into mitosis, the nuclear envelope breaks down, and the condensed chromosomes are exposed to the array of bipolar microtubules of the mitotic spindle. The kinetochore, a large, disc-shaped protein complex, is present at the centromere region of the sister chromatids and acts as a binding site for the microtubules.  Usually, the plus-end of a single microtubule is embedded within the kinetochore. However, some kinetochores first establish lateral contact with the side-wall of a...
Mechanisms of Membrane Domain Formation00:59

Mechanisms of Membrane Domain Formation

Different physical properties of lipids and proteins allow them to localize and form distinct islands or domains in the membrane. Some membrane domains are formed due to protein-protein interactions, whereas others are formed due to the presence of specific lipids such as sphingolipids and sterols—for example, large proteins, such as bacteriorhodopsin, aggregate and create distinct domains.
Another mechanism for membrane domain formation involves membrane proteins interacting with cytoskeletal...
The Movement of Organelles and Vesicles01:43

The Movement of Organelles and Vesicles
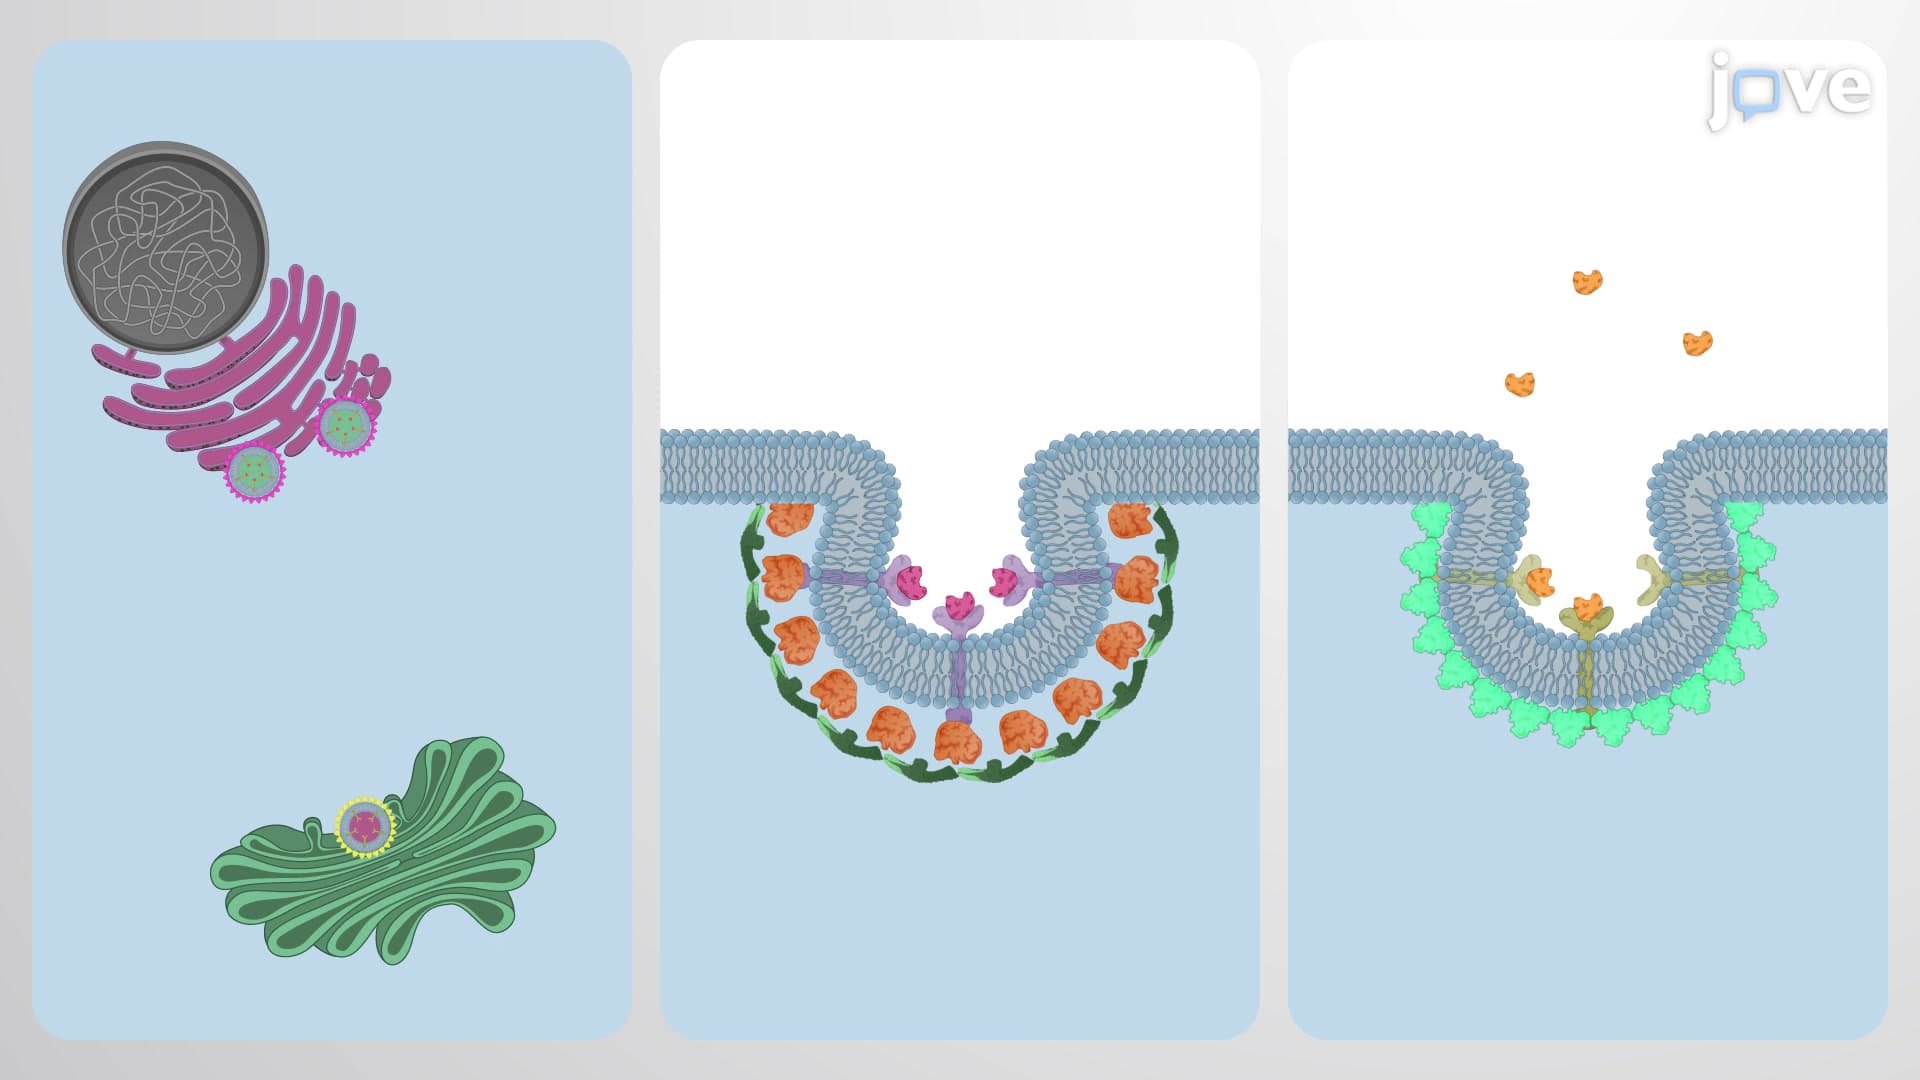
In eukaryotic cells,  cytoskeletal filaments such as actin, microtubules, and intermediate filaments form a mesh-like cytoskeletal network. These filaments serve as tracks for transporting cellular cargo. Specialized motor proteins use the chemical energy stored in adenosine triphosphate (ATP) for this transport. During interphase, microtubules are polarized, with the plus-end towards the cell periphery and the minus-end towards the cell center. Two microtubule-associated motor proteins,...
Introduction to Membrane Traffic01:44

Introduction to Membrane Traffic

The ER, Golgi apparatus, endosomes, and lysosomes work in tandem to modify, sort, and package proteins and lipids. An integrated membrane trafficking network facilitates the back and forth shuttling of molecules within different organelles in the same cell or across the cell membrane.
The transport of soluble and membrane proteins is mediated by transport vesicles that collect cargo from one cellular compartment and deliver it to another by fusing with the target organelle membrane. The Rab...
Intracellular Signaling Affects Focal Adhesions01:17

Intracellular Signaling Affects Focal Adhesions

Integrins act both as extracellular input receivers and as intracellular processing activators. As their name suggests, integrins are entirely integrated into the membrane structure. Their hydrophobic membrane-spanning regions interact with the phospholipid bilayer's hydrophobic region. These membrane receptors provide extracellular attachment sites for effectors like hormones and growth factors. They activate intracellular response cascades when their effectors are bound and active.
Some...