Related Experiment Video
Updated: May 23, 2026

From Constructs to Crystals – Towards Structure Determination of β-barrel Outer Membrane Proteins
Published on: July 4, 2016
The N-terminal domain of a TonB-dependent transporter undergoes a reversible stepwise denaturation
Ricardo H Flores Jiménez1, David S Cafiso
1Department of Chemistry, Biophysics Program, and Center for Membrane Biology, University of Virginia, Charlottesville, Virginia 22904-4319, United States.

Abstract:
Gram-negative bacteria contain a family of outer membrane transport proteins that function in the uptake of rare nutrients, such as iron and vitamin B(12). These proteins are termed TonB-dependent because transport requires an interaction with the inner-membrane protein TonB. Using a combination of site-directed spin labeling and chemical denaturation, we examined the site-specific unfolding of regions of the Escherichia coli vitamin B(12) transporter, BtuB. The data indicate that a portion of the N-terminal region of the protein, which occupies the lumen of the BtuB barrel, denatures prior to the unfolding of the barrel and that the free energy of folding for the N-terminus is smaller than that typically seen for globular proteins. Moreover, the data indicate that the N-terminal domain does not unfold in a single event but unfolds in a series of independent steps. The unfolding of the N-terminus is reversible, and removal of denaturant restores the native fold of the protein. These data are consistent with proposed transport mechanisms that involve a transient rearrangement or unfolding of the N-terminus of the protein, and they provide evidence of a specific protein conformation that might be an intermediate accessed during transport.
Related Concept Videos
 01:34
Protein Transport into the Inner Mitochondrial Membrane
Transport of mitochondrial precursors across the TIM23 channel is driven by...
 01:26
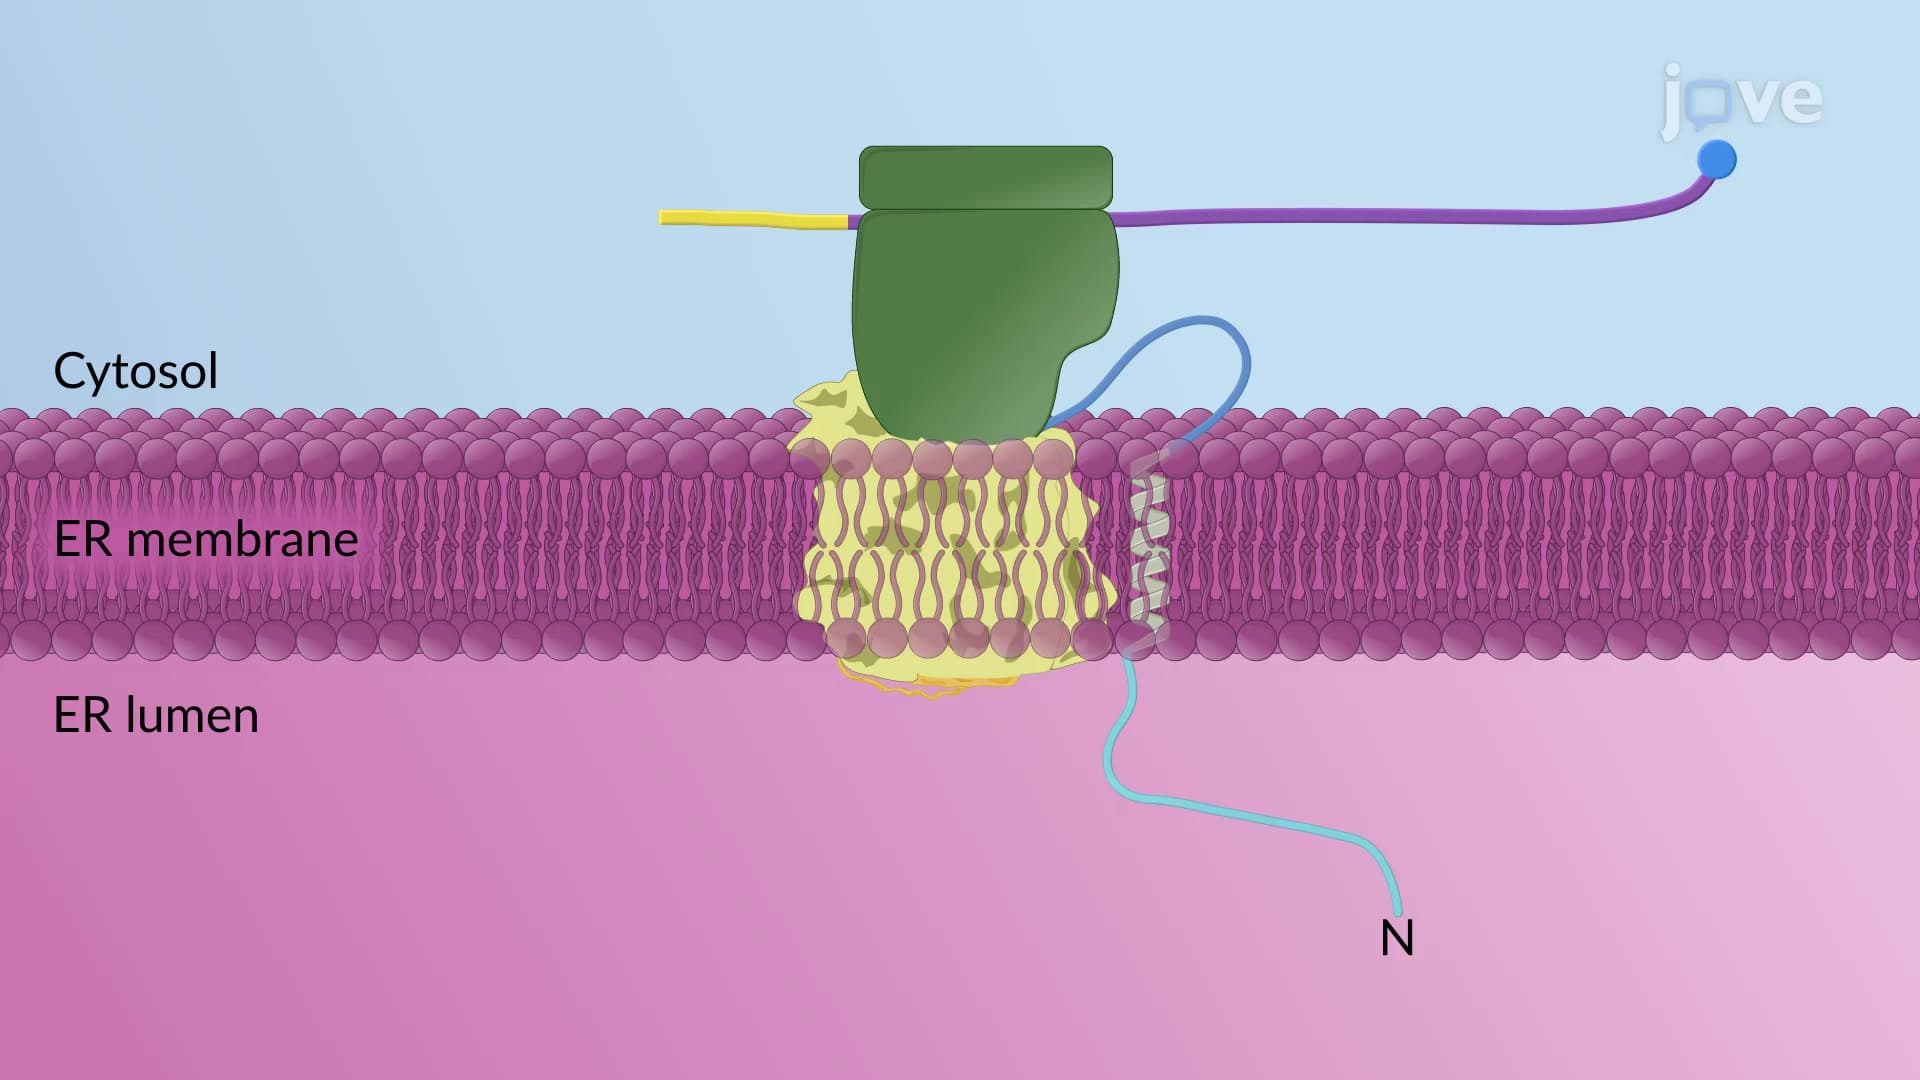
Insertion of Single-pass Transmembrane Proteins in the RER
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
 01:45
Tail-anchoring of Proteins in the ER Membrane
 01:37
Energy to Drive Translocation
Generally, polypeptides are unfolded by two distinct...
 01:19
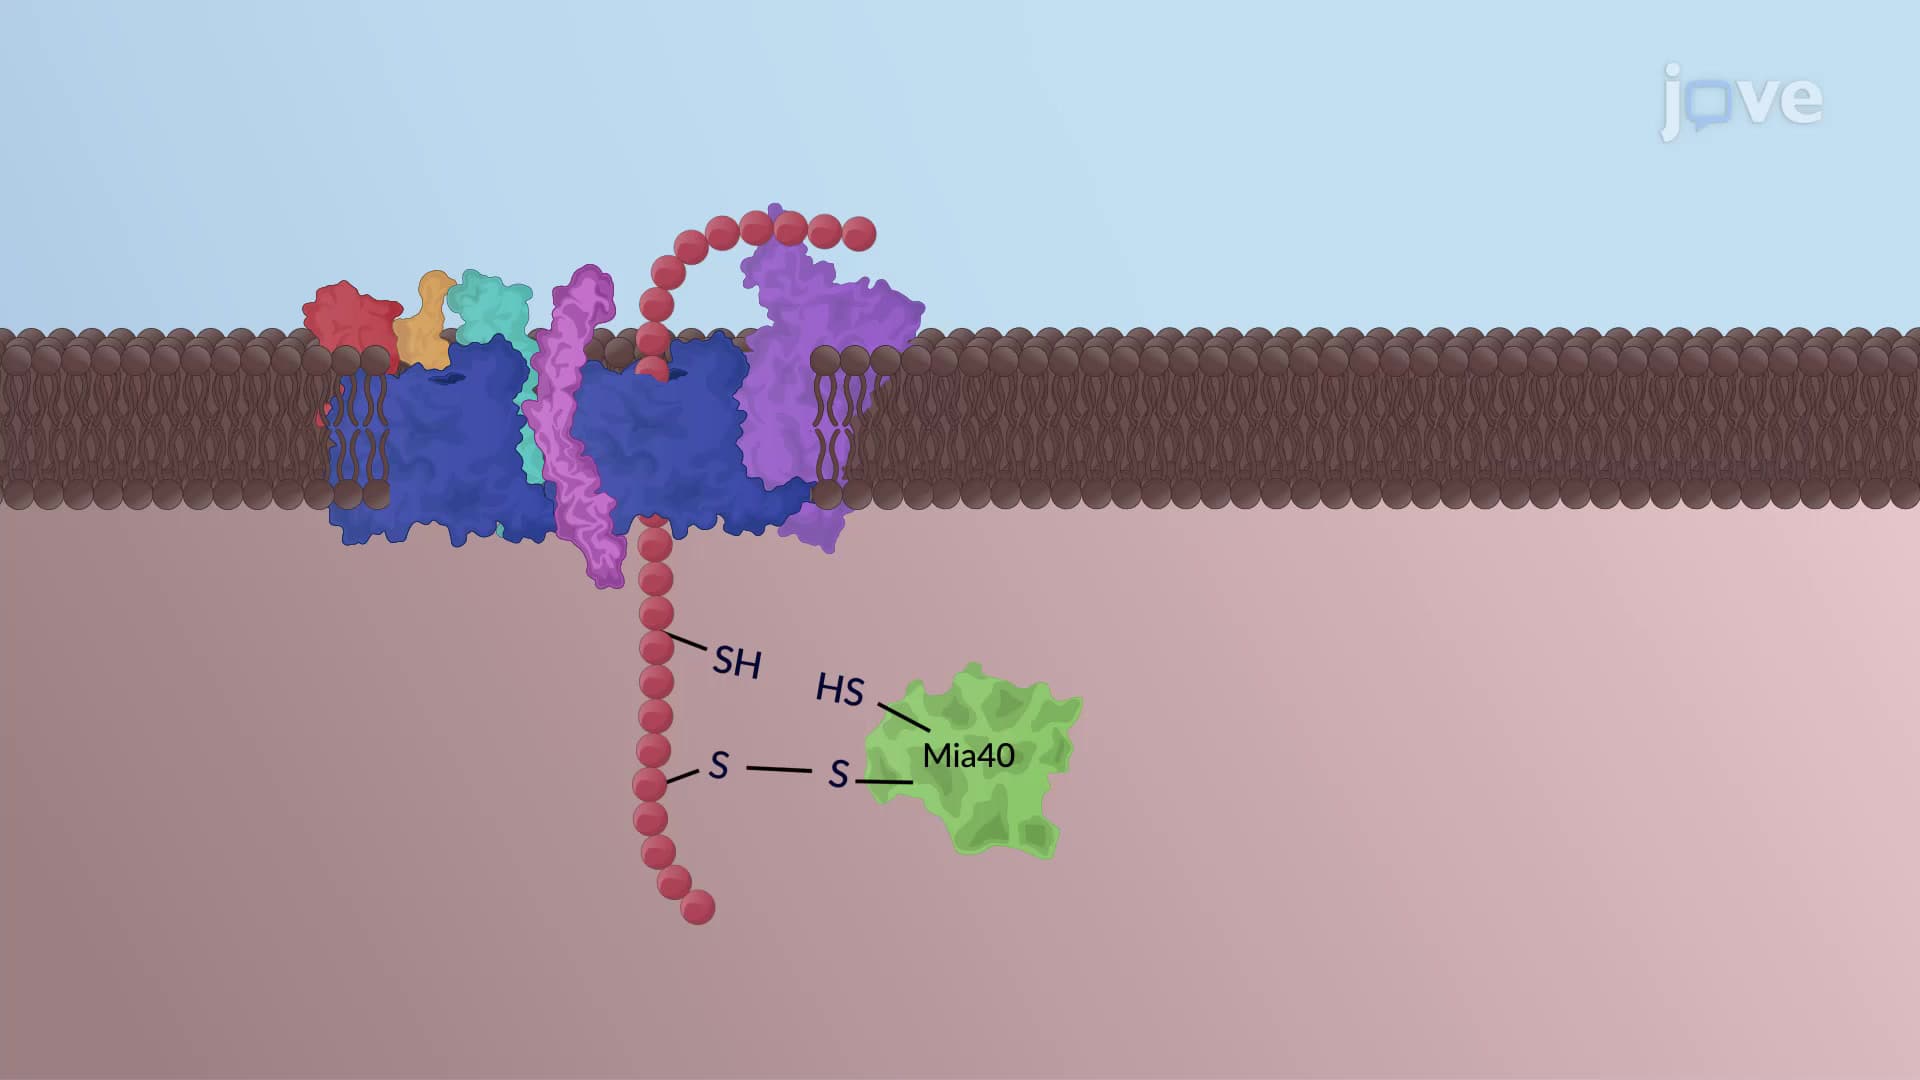
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:31
ABC Transporters: Exporter