Related Experiment Video
Updated: May 17, 2026
In Vitro Reconstitution of Self-Organizing Protein Patterns on Supported Lipid Bilayers
Published on: July 28, 2018
Origin of the conformational heterogeneity of cardiolipin-bound cytochrome C
Yuning Hong1, Julia Muenzner, Sebastian K Grimm
1Department of Chemistry, Dartmouth College, Hanover, New Hampshire 03755, United States.

Abstract:
Interactions of cytochrome c (cyt c) with cardiolipin (CL) partially unfold the protein, activating its peroxidase function, a critical event in the execution of apoptosis. However, structural features of the altered protein species in the heterogeneous ensemble are difficult to probe with ensemble averaging. Analyses of the dye-to-heme distance distributions P(r) from time-resolved FRET (TR-FRET) have uncovered two distinct types of CL-bound cyt c conformations, extended and compact. We have combined TR-FRET, fluorescence correlation spectroscopy (FCS), and biolayer interferometry to develop a systematic understanding of the functional partitioning between the two conformations. The two subpopulations are in equilibrium with each other, with a submillisecond rate of conformational exchange reflecting the protein folding into a compact non-native state, as well as protein interactions with the lipid surface. Electrostatic interactions with the negatively charged lipid surface that correlate with physiologically relevant changes in CL concentrations strongly affect the kinetics of cyt c binding and conformational exchange. A predominantly peripheral binding mechanism, rather than deep protein insertion into the membrane, provides a rationale for the general denaturing effect of the CL surface and the large-scale protein unfolding. These findings closely relate to cyt c folding dynamics and suggest a general strategy for extending the time window in monitoring the kinetics of folding.
More Related Videos
Related Concept Videos
 01:35
Asymmetric Lipid Bilayer
 01:28
The Inner Mitochondrial Membrane
 01:41
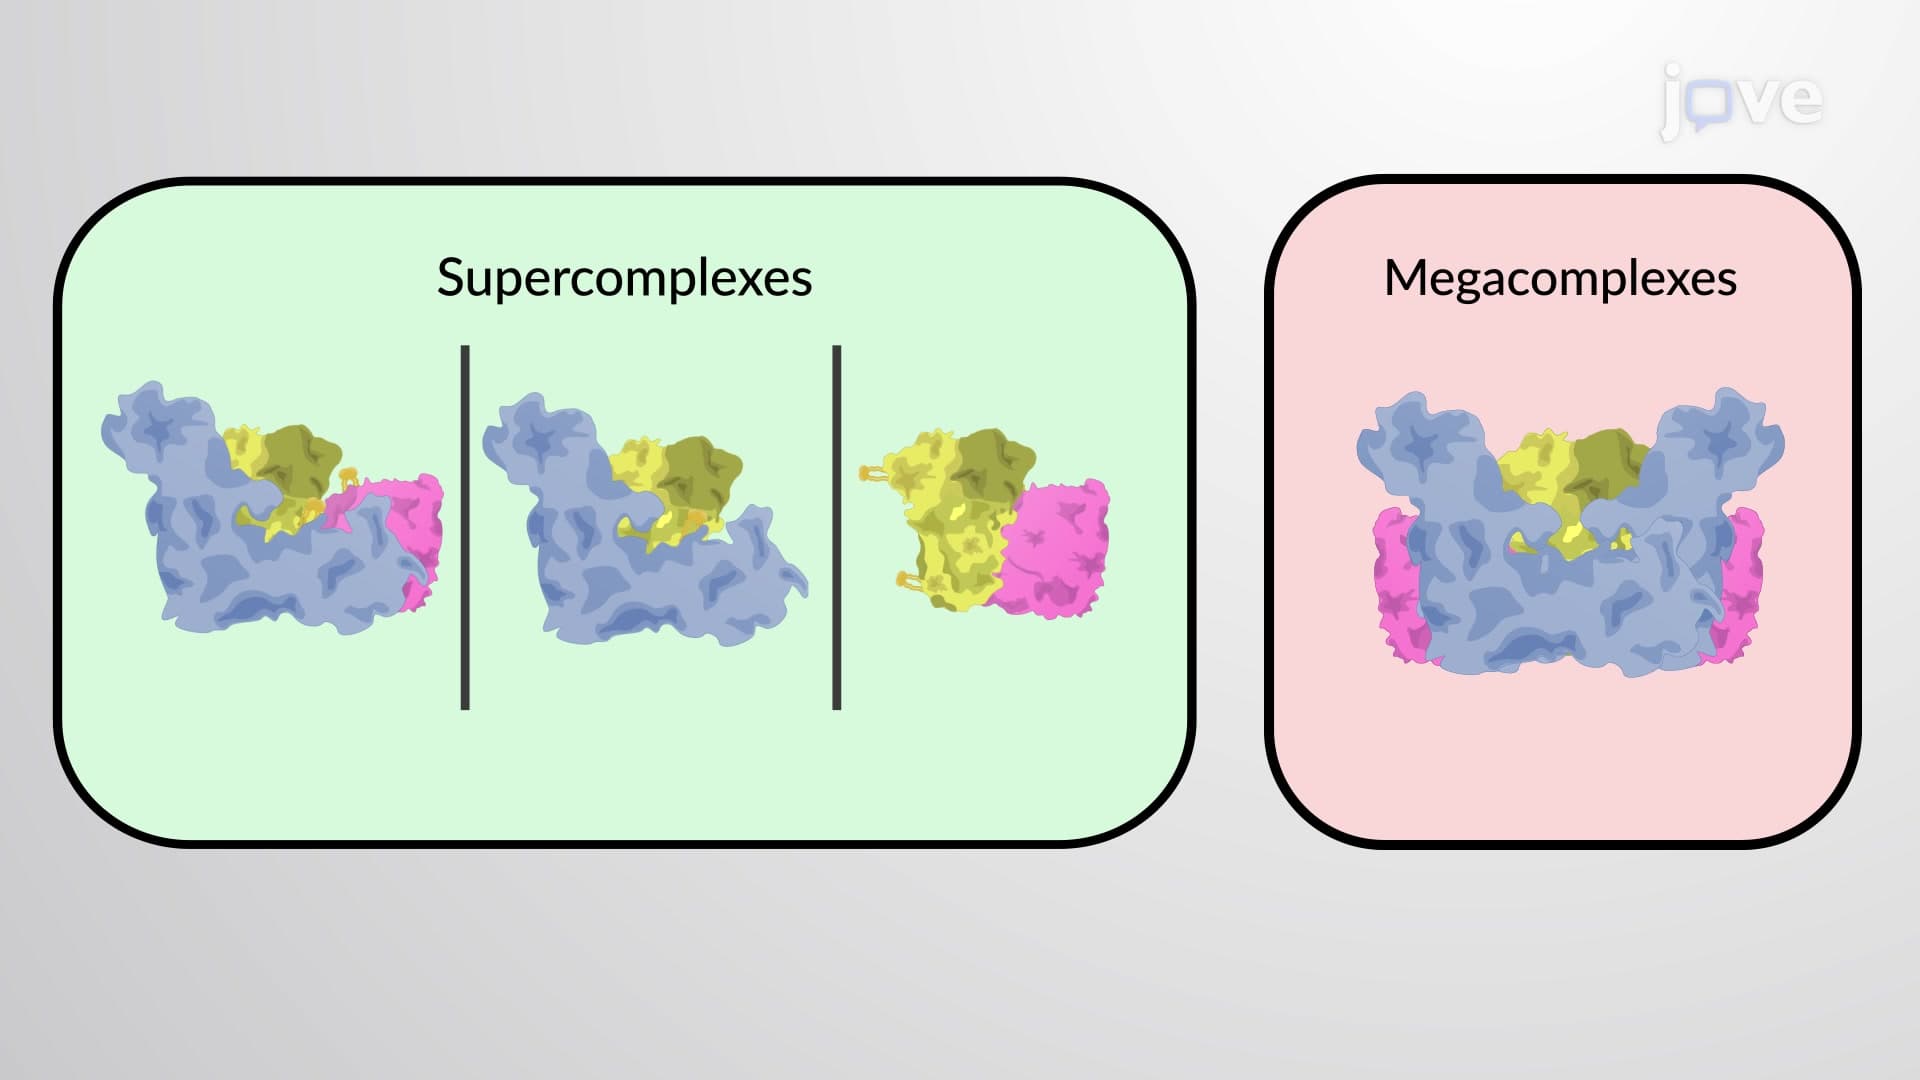
The Supercomplexes in the Crista Membrane
 01:43
Electron Transport Chain: Complex III and IV
 01:26
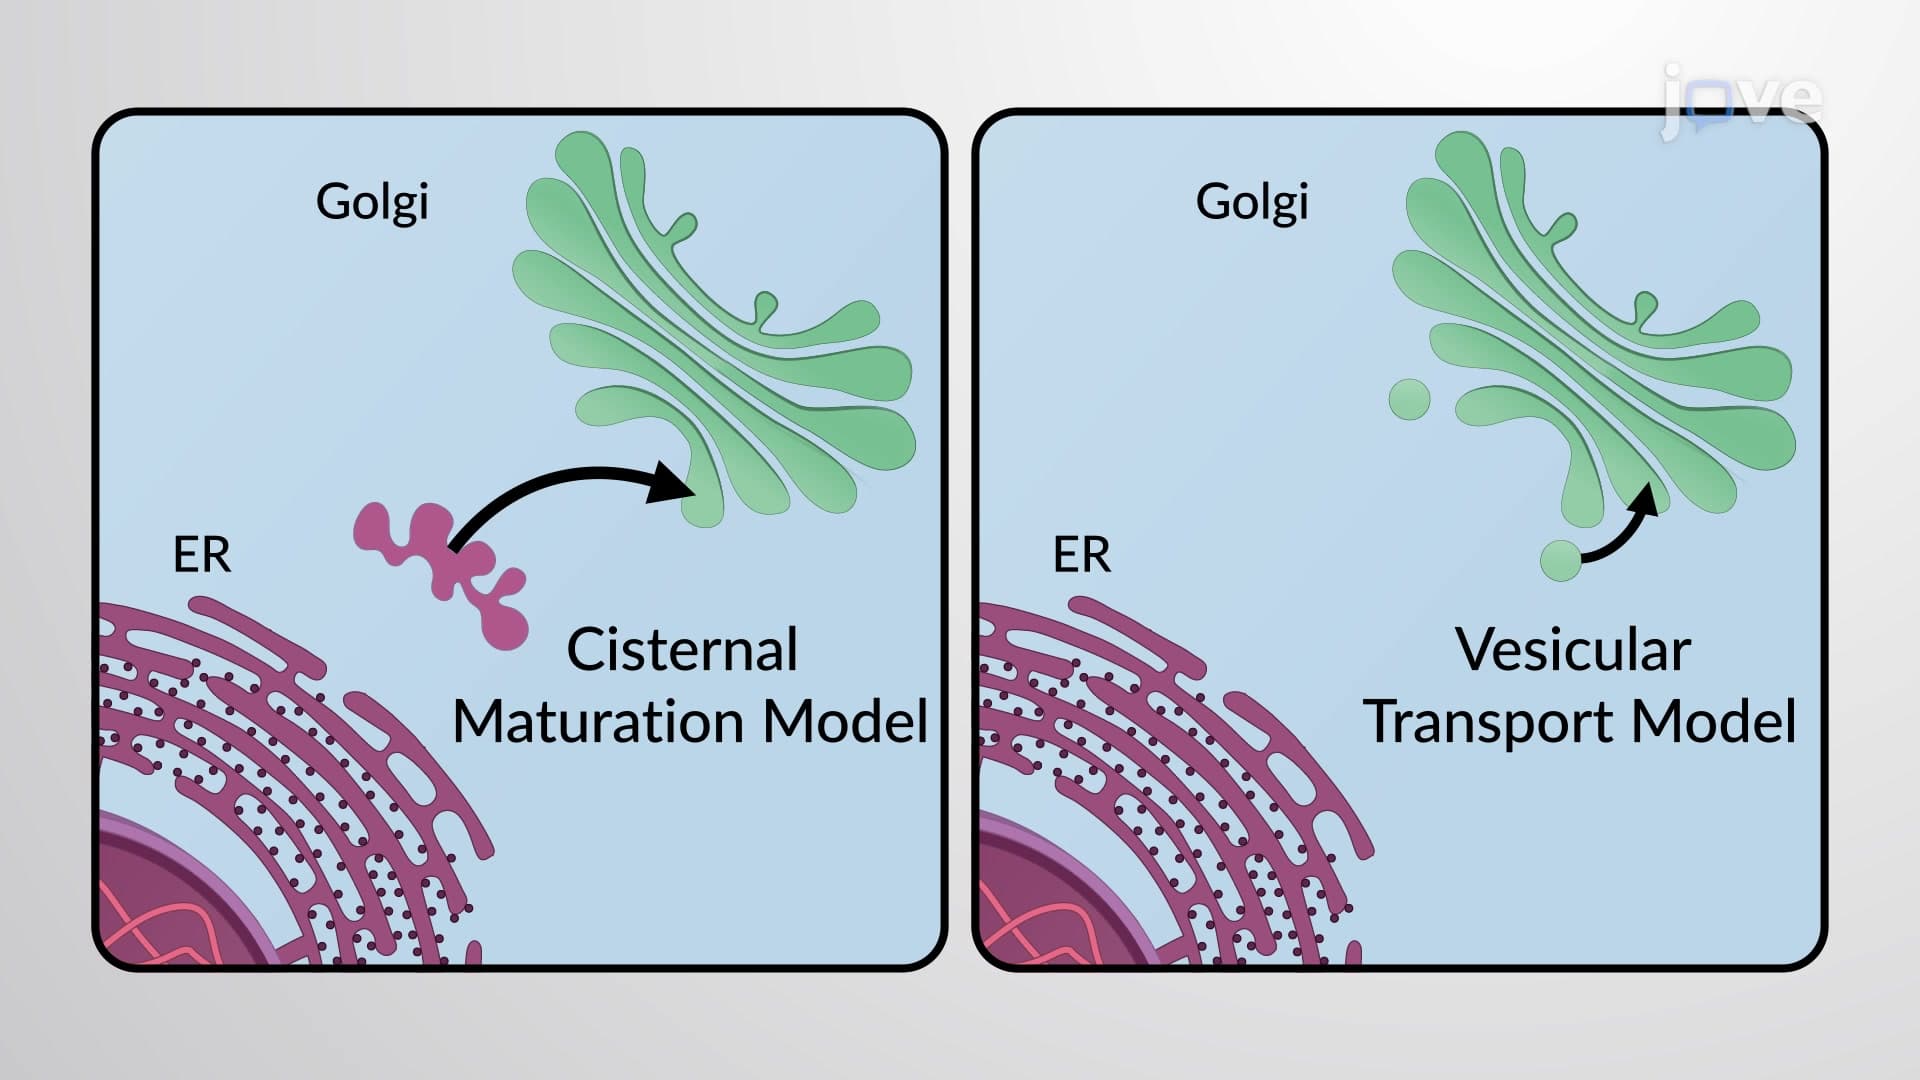
Transport Across the Golgi
 01:28
Assembly of the Lipid Bilayer in the ER
A large chunk of any biological membrane is composed of phospholipids. These lipids have a heterogeneous distribution across different subcellular organelles and even between...