Related Experiment Video
Updated: May 17, 2026

Förster Resonance Energy Transfer Mapping: A New Methodology to Elucidate Global Structural Features
Published on: March 16, 2022
Orientation of internal signal-anchor sequences at the Sec61 translocon
Lucyna Kocik1, Tina Junne, Martin Spiess
1Biozentrum, University of Basel, Klingelbergstrasse 70, CH-4056 Basel, Switzerland.

Translocation and insertion of secretory and membrane proteins at the endoplasmic reticulum are mediated by the Sec61 translocon. Evidence from in vivo as well as in vitro experiments indicates that N-terminal signal-anchor sequences initially insert N-first before they invert their orientation to translocate the C-terminus. Inversion is driven by flanking charges according to the positive-inside rule and inhibited by increased signal hydrophobicity. Here, we show that upon extending the N-terminal hydrophilic domain preceding the signal core to more than ~20 residues, the insertion behavior changes. Apparent signal inversion and the effect of hydrophobicity are largely lost, suggesting that N-first insertion is limited to N-terminal signal anchors. Extended N-domains sterically hinder N-translocation in a length-dependent manner also for reverse signal anchors with inverted flanking charges. The results indicate a mechanistic difference in the insertion process of N-terminal and internal signal sequences.
Translocation and insertion of secretory and membrane proteins at the endoplasmic reticulum are mediated by the Sec61 translocon. Evidence from in vivo as well as in vitro experiments indicates that N-terminal signal-anchor sequences initially insert N-first before they invert their orientation to translocate the C-terminus. Inversion is driven by flanking charges according to the positive-inside rule and inhibited by increased signal hydrophobicity. Here, we show that upon extending the N-terminal hydrophilic domain preceding the signal core to more than ~20 residues, the insertion behavior changes. Apparent signal inversion and the effect of hydrophobicity are largely lost, suggesting that N-first insertion is limited to N-terminal signal anchors. Extended N-domains sterically hinder N-translocation in a length-dependent manner also for reverse signal anchors with inverted flanking charges. The results indicate a mechanistic difference in the insertion process of N-terminal and internal signal sequences.
Related Concept Videos
 01:26
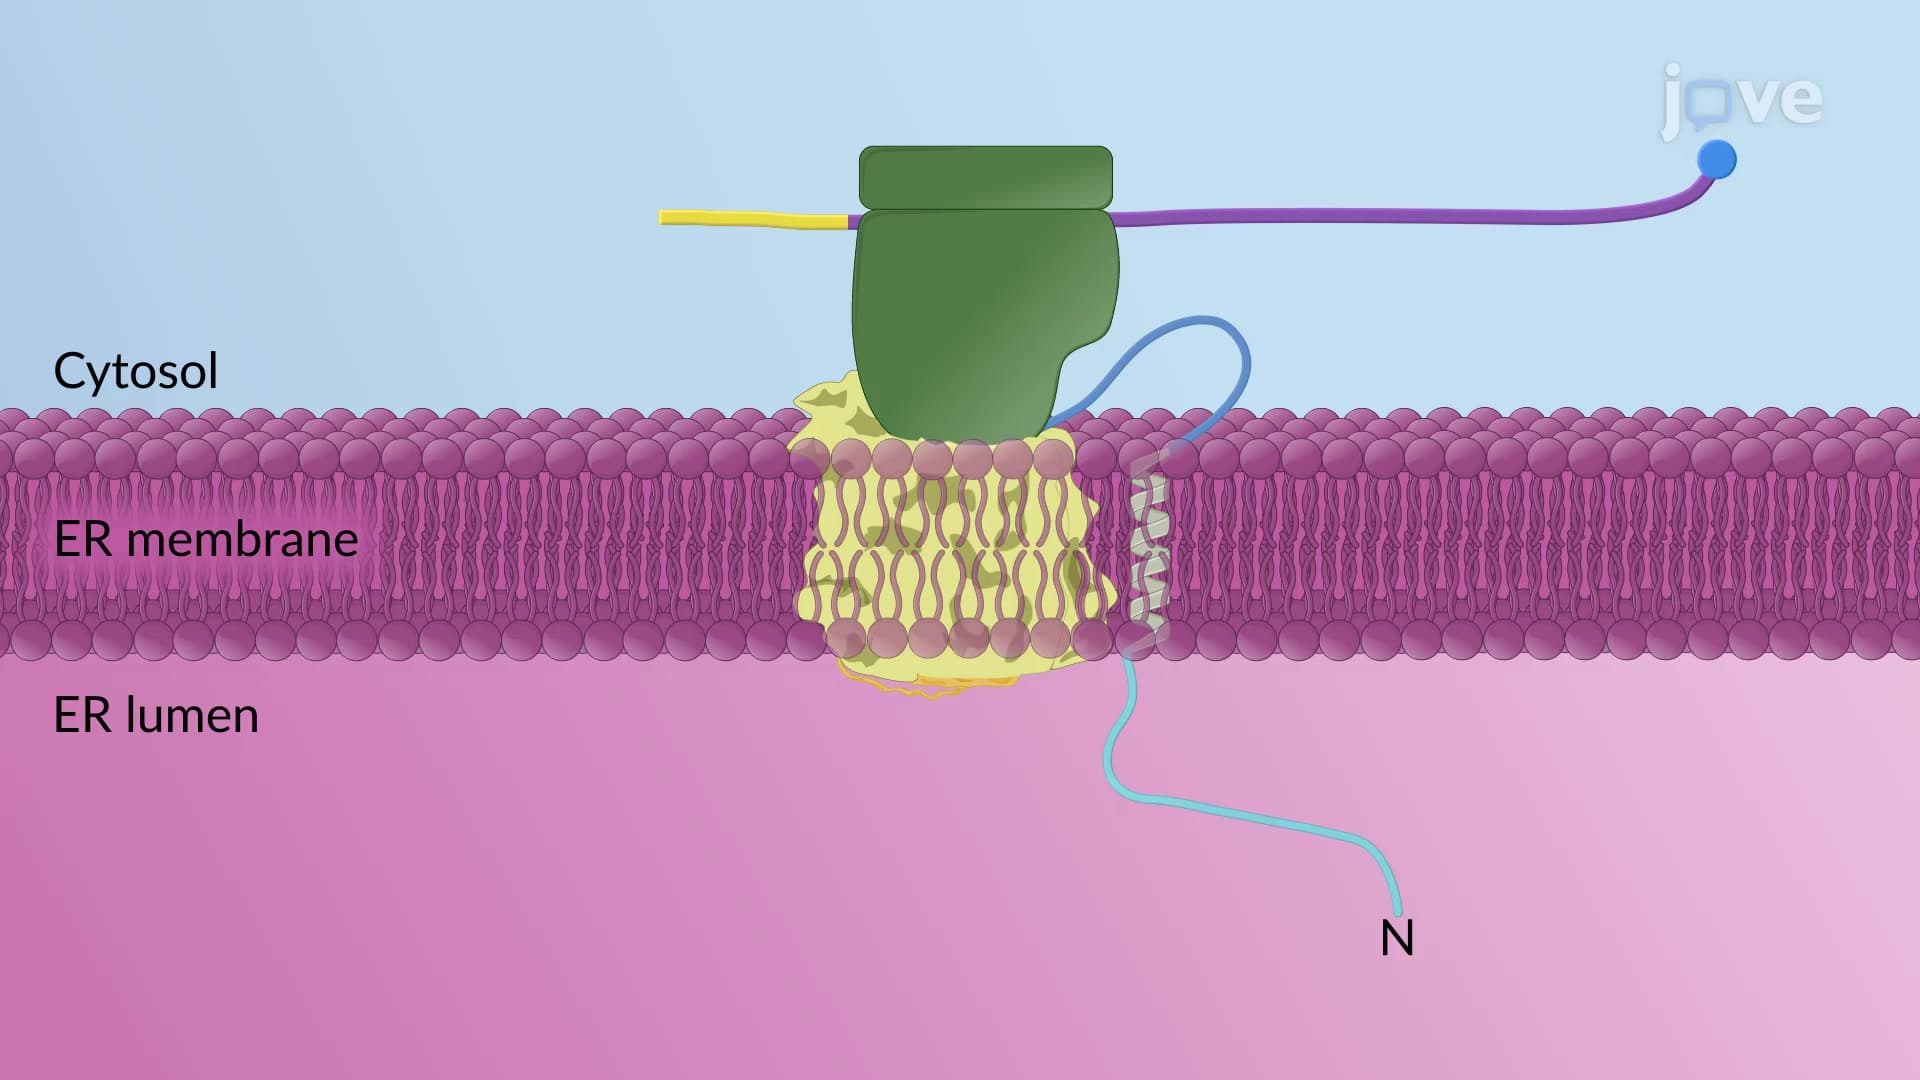
Insertion of Single-pass Transmembrane Proteins in the RER
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
 01:20
Cotranslational Protein Translocation
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
 01:28
Protein Translocation Machinery on the ER Membrane
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the translocon complex.
 01:45
Tail-anchoring of Proteins in the ER Membrane
 01:29
GPI Anchoring of Proteins in the ER Membrane
GPI-anchor structure
A sequence of 11 enzymatic reactions results in the synthesis of the complete GPI anchor consisting of a hydrophobic and a hydrophilic portion. The hydrophobic portion comprises phosphatidylinositol, while the hydrophilic part comprises polar groups like phosphoethanolamine,...
 01:27
Post-translational Translocation of Proteins to the RER
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...