Related Experiment Video
Updated: May 17, 2026

Construction of Cyclic Cell-Penetrating Peptides for Enhanced Penetration of Biological Barriers
Published on: September 19, 2022
Cyclotides insert into lipid bilayers to form membrane pores and destabilize the membrane through hydrophobic and
Conan K Wang1, Hanna P Wacklin, David J Craik
1University of Queensland, Institute for Molecular Bioscience, Brisbane, Queensland 4072, Australia.

Abstract:
Cyclotides are a family of plant-derived circular proteins with potential therapeutic applications arising from their remarkable stability, broad sequence diversity, and range of bioactivities. Their membrane-binding activity is believed to be a critical component of their mechanism of action. Using isothermal titration calorimetry, we studied the binding of the prototypical cyclotides kalata B1 and kalata B2 (and various mutants) to dodecylphosphocholine micelles and phosphoethanolamine-containing lipid bilayers. Although binding is predominantly an entropy-driven process, suggesting that hydrophobic forces contribute significantly to cyclotide-lipid complex formation, specific binding to the phosphoethanolamine-lipid headgroup is also required, which is evident from the enthalpic changes in the free energy of binding. In addition, using a combination of dissipative quartz crystal microbalance measurements and neutron reflectometry, we elucidated the process by which cyclotides interact with bilayer membranes. Initially, a small number of cyclotides bind to the membrane surface and then insert first into the outer membrane leaflet followed by penetration through the membrane and pore formation. At higher concentrations of cyclotides, destabilization of membranes occurs. Our results provide significant mechanistic insight into how cyclotides exert their bioactivities.
Related Concept Videos
 00:59
Mechanisms of Membrane Domain Formation
Another mechanism for membrane domain formation involves membrane proteins interacting with cytoskeletal...
 01:17
Pore Transport and Ion-Pair Transport
Pore transport, also known as convective transport, is a process where small molecules like urea, water, and sugars rapidly cross cell membranes as though there were channels or pores in the membrane. Although direct microscopic evidence is limited but the concept of pores or channels is widely accepted based on physiological evidence. Despite the lack of direct microscopic...
 01:26
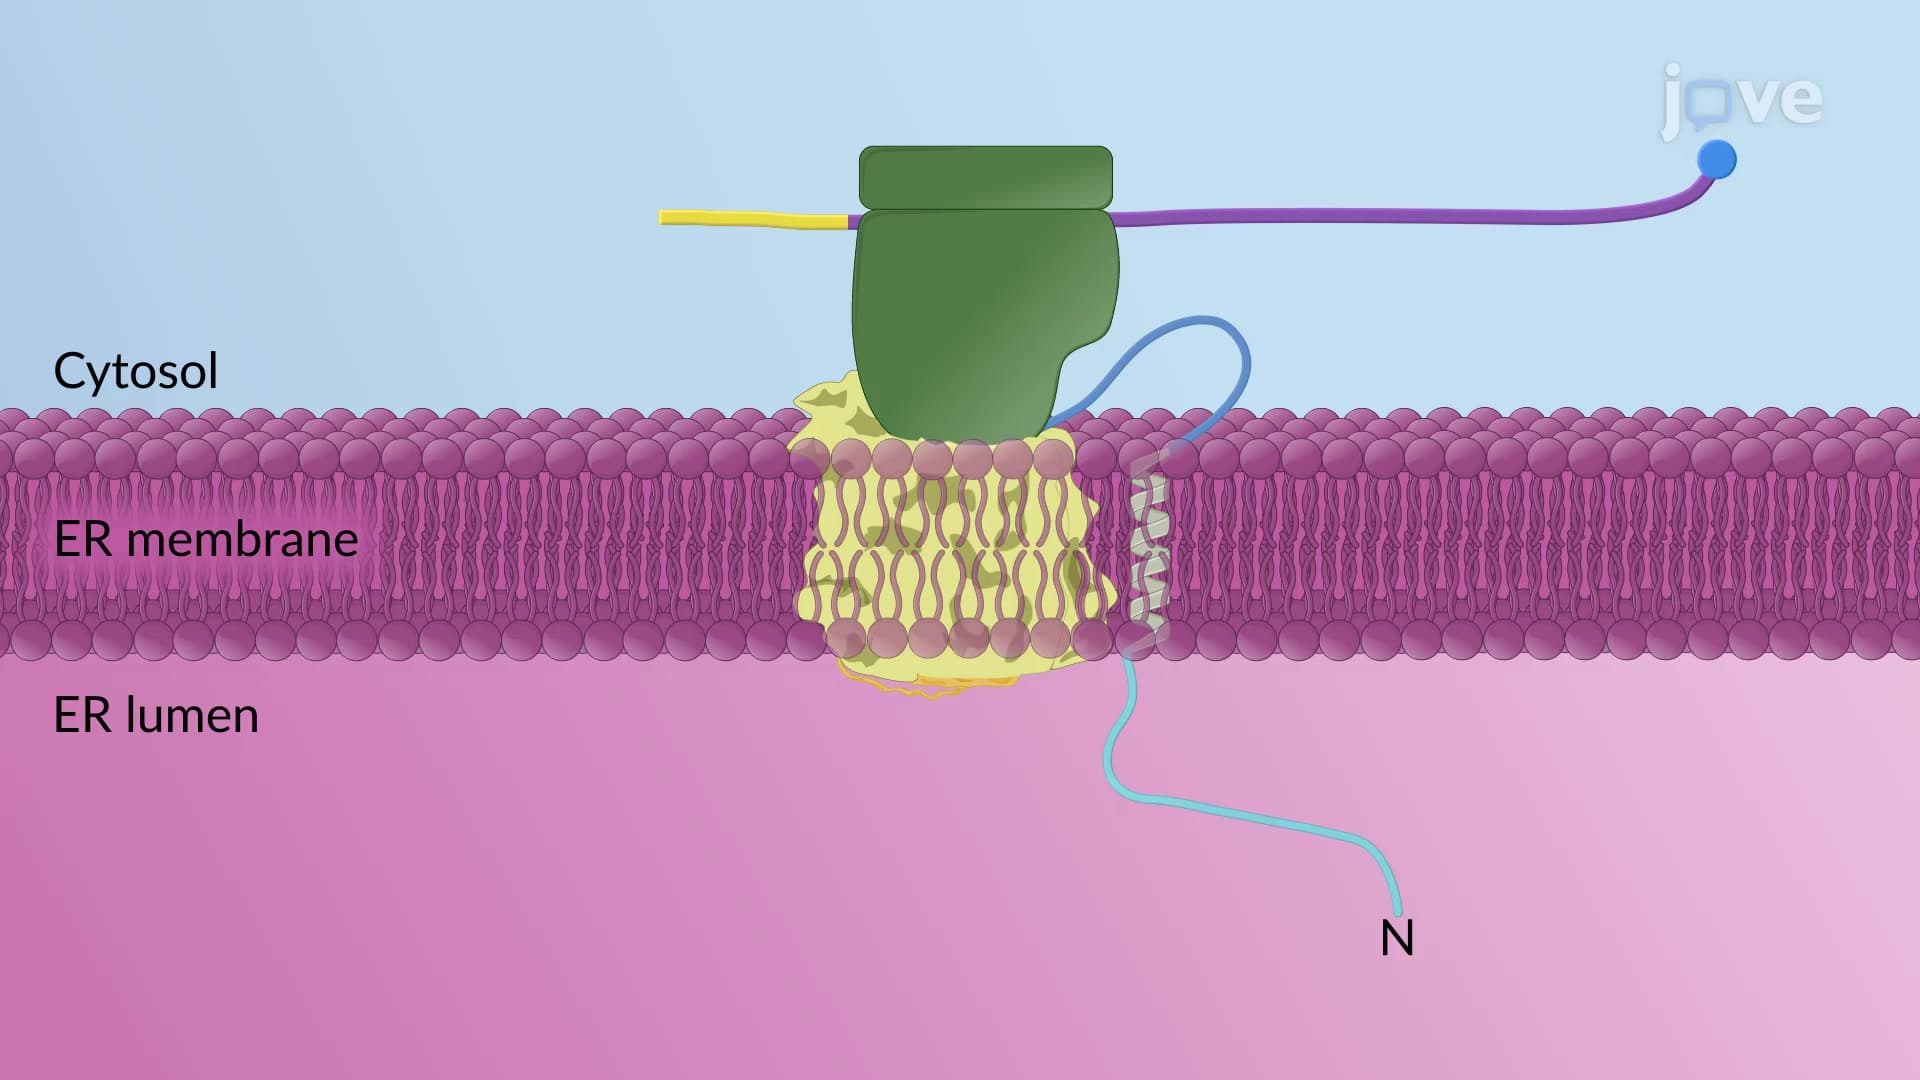
Insertion of Single-pass Transmembrane Proteins in the RER
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
 01:35
Asymmetric Lipid Bilayer
 01:09
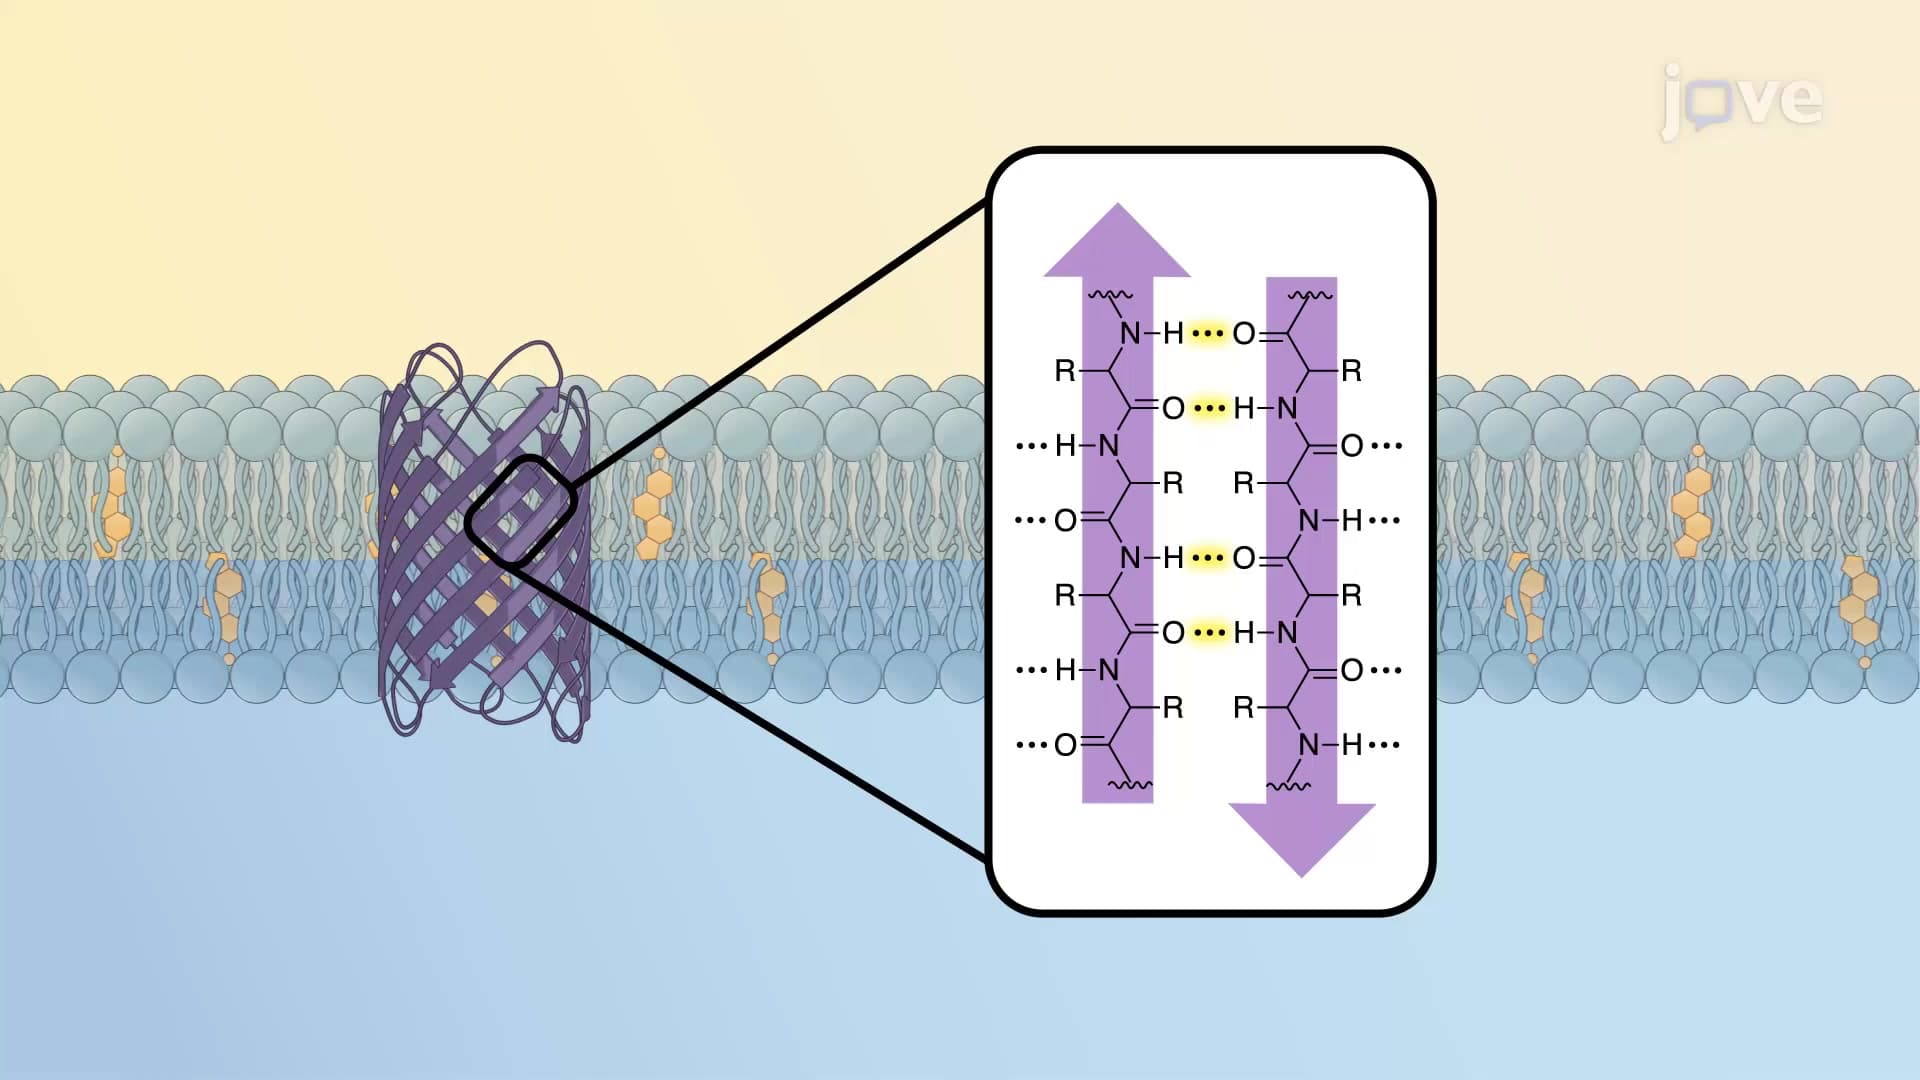
Multi-pass Transmembrane Proteins and β-barrels
α-Helix containing multi-pass transmembrane proteins
Multi-pass transmembrane proteins such as G-protein-linked receptors (GPCRs) and...
 01:12
Clathrin Coated Vesicles