Related Experiment Video
Updated: May 16, 2026

Transmembrane Domain Oligomerization Propensity determined by ToxR Assay
Published on: May 26, 2011
Altering hydrophobic sequence lengths shows that hydrophobic mismatch controls affinity for ordered lipid domains
1Department of Biochemistry and Cell Biology, Stony Brook University, Stony Brook, New York 11794-5215, USA.

Abstract:
The hypothesis that mismatch between transmembrane (TM) length and bilayer width controls TM protein affinity for ordered lipid domains (rafts) was tested using perfringolysin O (PFO), a pore-forming cholesterol-dependent cytolysin. PFO forms a multimeric barrel with many TM segments. The properties of PFO mutants with lengthened or shortened TM segments were compared with that of PFO with wild type TM sequences. Both mutant and wild type length PFO exhibited cholesterol-dependent membrane insertion. Maximal PFO-induced pore formation occurred in vesicles with wider bilayers for lengthened TM segments and in thinner bilayers for shortened TM segments. In diC(18:0) phosphatidylcholine (PC)/diC(14:1) PC/cholesterol vesicles, which form ordered domains with a relatively thick bilayer and disordered domains with a relatively thin bilayer, affinity for ordered domains was greatest with lengthened TM segments and least with shortened TM segments as judged by FRET. Similar results were observed by microscopy in giant vesicles containing sphingomyelin in place of diC(18:0) PC. In contrast, in diC(16:0) PC/diC(14:0) PC/diC(20:1) PC/cholesterol vesicles, which should form ordered domains with a relatively thin bilayer and disordered domains with a relatively thick bilayer, relative affinity for ordered domains was greatest with shortened TM segments and least with lengthened TM segments. The inability of multi-TM segment proteins (unlike single TM segment proteins) to adapt to mismatch by tilting may explain the sensitivity of raft affinity to mismatch. The difference in width sensitivity for single and multi-TM helix proteins may link raft affinity to multimeric state and thus control the assembly of multimeric TM complexes in rafts.
Insights
Transmembrane protein length mismatch with lipid bilayer width influences protein affinity for membrane rafts. This finding is crucial for understanding how multi-transmembrane segment proteins assemble in rafts.
Area of Science:
- Biochemistry
- Membrane Biology
- Protein-Lipid Interactions
Background:
- Transmembrane (TM) proteins are crucial for cellular functions.
- Lipid rafts are specialized membrane domains that compartmentalize cellular processes.
- The interaction between TM proteins and lipid rafts is vital for protein function and assembly.
Purpose of the Study:
- To investigate the hypothesis that the mismatch between transmembrane (TM) length and lipid bilayer width controls TM protein affinity for ordered lipid domains (rafts).
- To elucidate the role of TM segment length in the membrane insertion and pore formation of perfringolysin O (PFO).
Main Methods:
- Utilized perfringolysin O (PFO), a pore-forming cholesterol-dependent cytolysin, and its mutants with altered TM segment lengths.
- Employed Förster Resonance Energy Transfer (FRET) and microscopy on various vesicle compositions to assess protein-lipid domain interactions.
- Compared PFO behavior in lipid vesicles with differing bilayer thicknesses and domain properties.
Main Results:
- Both wild-type and mutant PFO showed cholesterol-dependent membrane insertion.
- Maximal PFO pore formation correlated with bilayer width matching TM segment length.
- PFO affinity for ordered lipid domains varied significantly with TM length and bilayer width, with longer TM segments preferring thicker bilayers and shorter segments preferring thinner bilayers.
Conclusions:
- Transmembrane segment length and lipid bilayer width mismatch critically regulates TM protein affinity for lipid rafts.
- Multi-transmembrane segment proteins, unlike single-TM proteins, exhibit limited adaptability to bilayer width variations, potentially due to their inability to tilt.
- This width sensitivity links raft affinity to the multimeric state of proteins, influencing the assembly of TM complexes within rafts.
Related Concept Videos
 01:26
Membrane Fluidity
Mosaic nature of the membrane
The mosaic characteristic of the membrane helps the plasma membrane remain fluid. The integral proteins and lipids exist as separate but loosely-attached molecules in the membrane. The membrane is a relatively...
 01:23
Membrane Fluidity
 01:35
Asymmetric Lipid Bilayer
 01:19
Membrane Asymmetry Regulating Transporters
Flippase
Eukaryotic flippases are type-IV P-type ATPases or P4-ATPases belonging to P-type ATPase family proteins that are membrane-bound pumps involved in the ATP-mediated transport of ions and molecules across the membrane. Flippases flip specific phospholipids from the outer to the inner leaflet of a membrane. All P4-ATPases have one...
 01:19
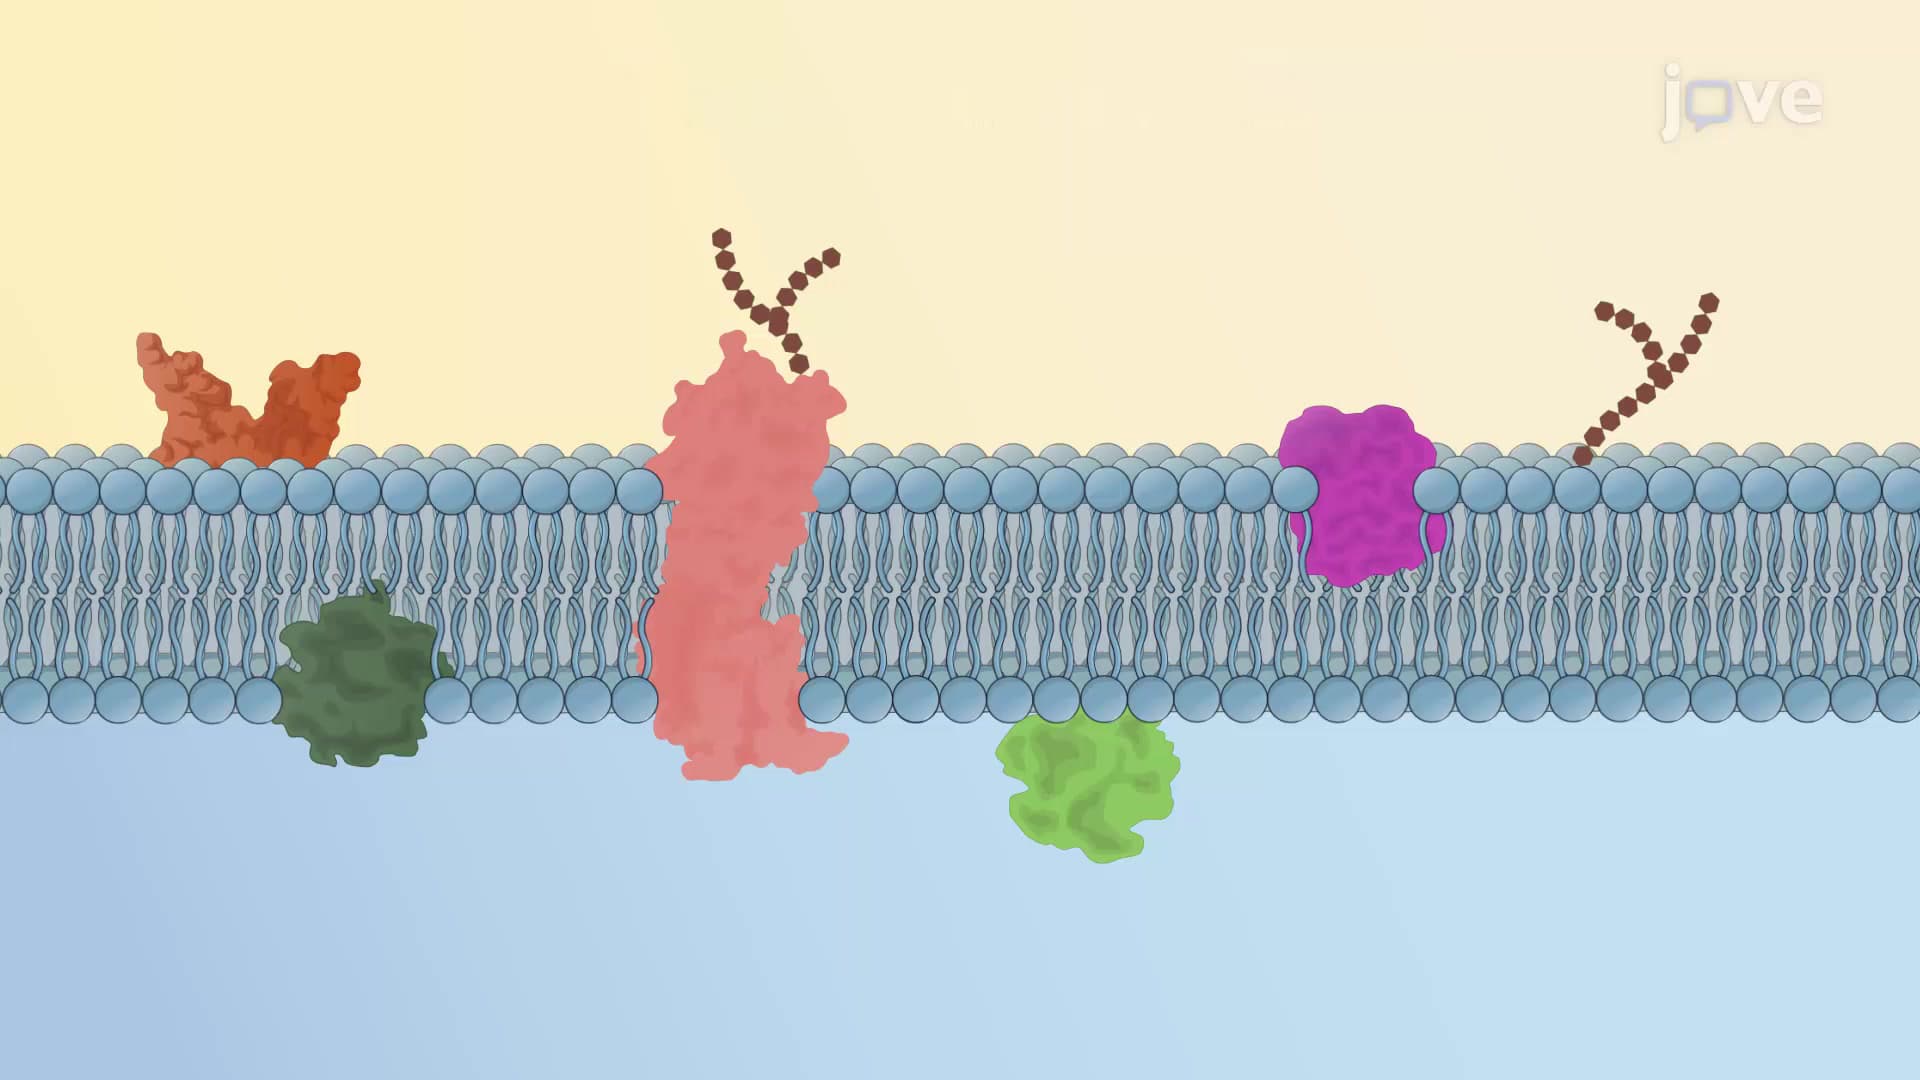
Fluid Mosaic Model
 01:29
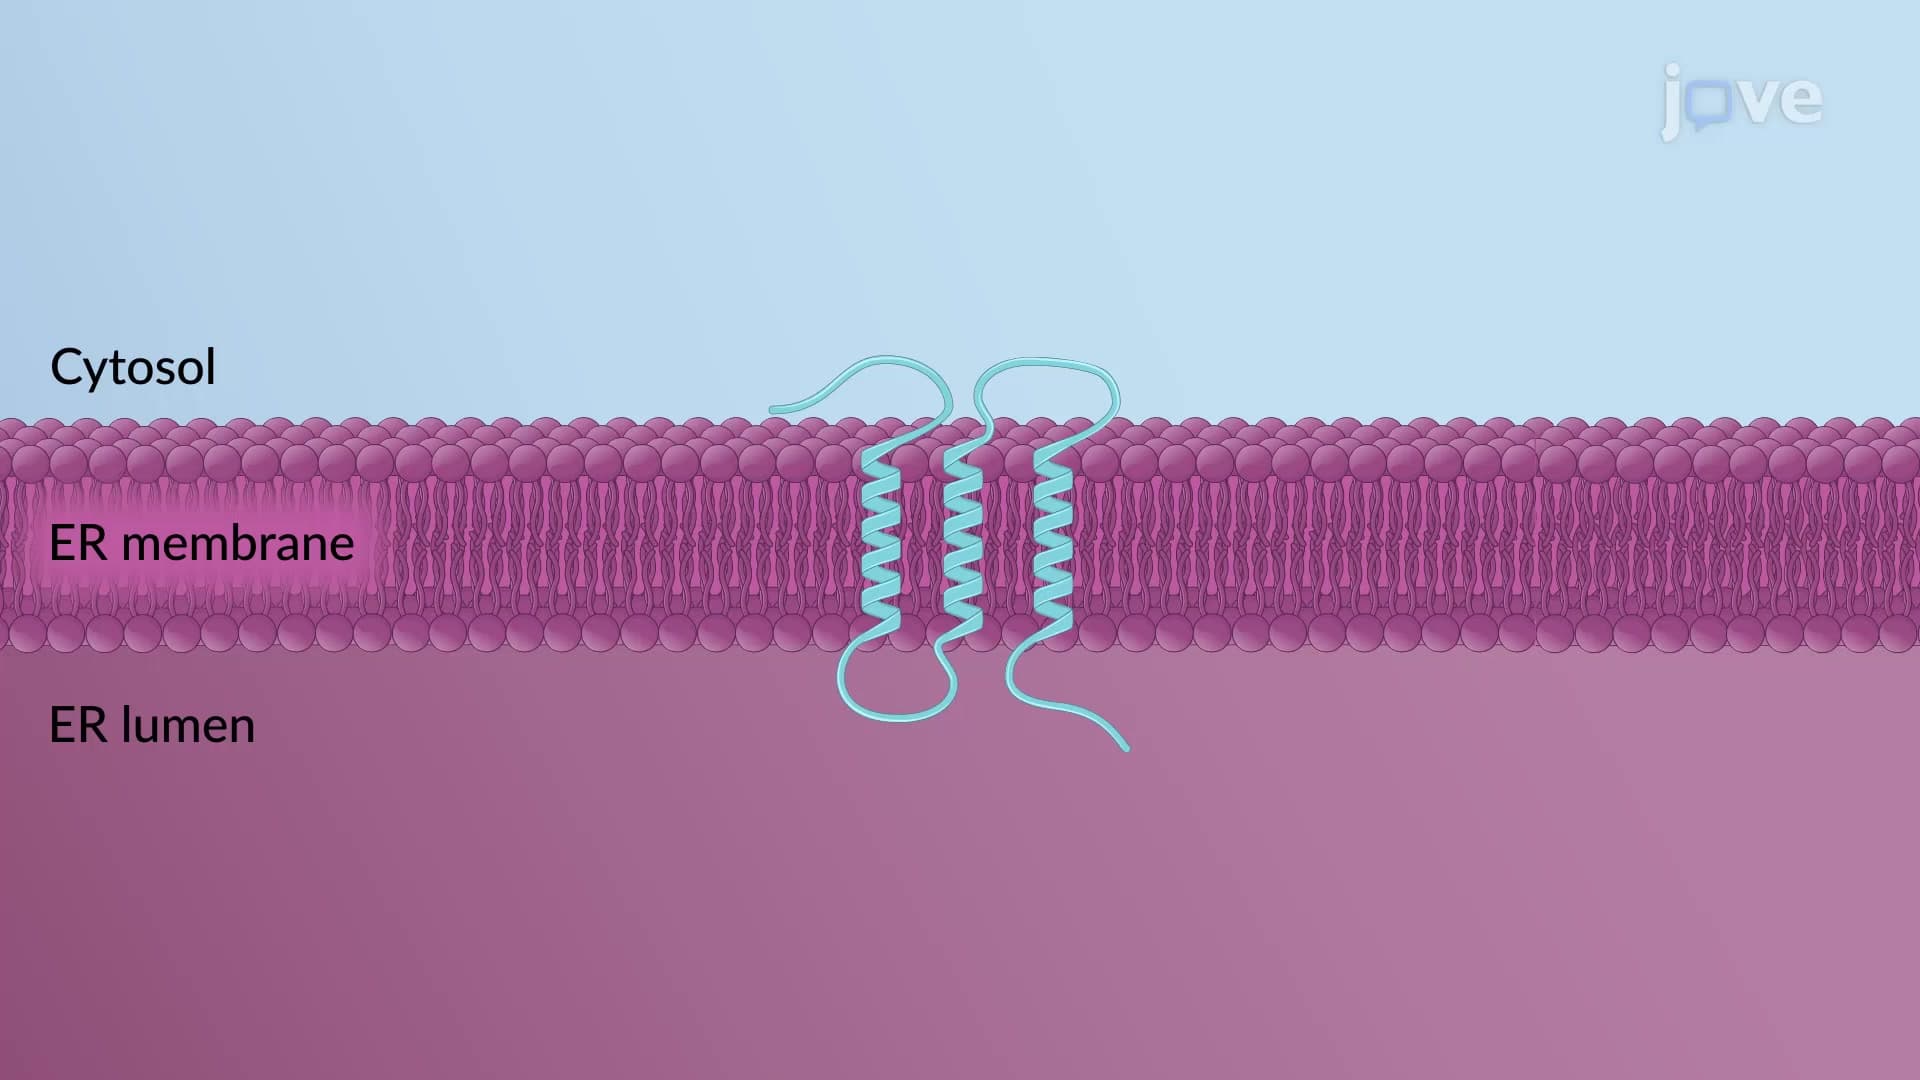
Insertion of Multi-pass Transmembrane Proteins in the RER
The multipass transmembrane proteins are the type IV integral membrane proteins with multiple topogenic sequences determining their spatial arrangement in the ER membrane. Nearly all multipass proteins lack a cleavable signal sequence and use...