Related Experiment Video
Updated: May 15, 2026
High Throughput In Vitro Assessment of Latency Reversing Agents on HIV Transcription and Splicing
Published on: January 22, 2019
BET bromodomain-targeting compounds reactivate HIV from latency via a Tat-independent mechanism
Daniela Boehm1, Vincenzo Calvanese, Roy D Dar
1Gladstone Institute of Virology and Immunology, San Francisco, CA, USA.

The therapeutic potential of pharmacologic inhibition of bromodomain and extraterminal (BET) proteins has recently emerged in hematological malignancies and chronic inflammation. We find that BET inhibitor compounds (JQ1, I-Bet, I-Bet151 and MS417) reactivate HIV from latency. This is evident in polyclonal Jurkat cell populations containing latent infectious HIV, as well as in a primary T-cell model of HIV latency. Importantly, we show that this activation is dependent on the positive transcription elongation factor p-TEFb but independent from the viral Tat protein, arguing against the possibility that removal of the BET protein BRD4, which functions as a cellular competitor for Tat, serves as a primary mechanism for BET inhibitor action. Instead, we find that the related BET protein, BRD2, enforces HIV latency in the absence of Tat, pointing to a new target for BET inhibitor treatment in HIV infection. In shRNA-mediated knockdown experiments, knockdown of BRD2 activates HIV transcription to the same extent as JQ1 treatment, while a lesser effect is observed with BRD4. In single-cell time-lapse fluorescence microscopy, quantitative analyses across ~2,000 viral integration sites confirm the Tat-independent effect of JQ1 and point to positive effects of JQ1 on transcription elongation, while delaying re-initiation of the polymerase complex at the viral promoter. Collectively, our results identify BRD2 as a new Tat-independent suppressor of HIV transcription in latently infected cells and underscore the therapeutic potential of BET inhibitors in the reversal of HIV latency.
The therapeutic potential of pharmacologic inhibition of bromodomain and extraterminal (BET) proteins has recently emerged in hematological malignancies and chronic inflammation. We find that BET inhibitor compounds (JQ1, I-Bet, I-Bet151 and MS417) reactivate HIV from latency. This is evident in polyclonal Jurkat cell populations containing latent infectious HIV, as well as in a primary T-cell model of HIV latency. Importantly, we show that this activation is dependent on the positive transcription elongation factor p-TEFb but independent from the viral Tat protein, arguing against the possibility that removal of the BET protein BRD4, which functions as a cellular competitor for Tat, serves as a primary mechanism for BET inhibitor action. Instead, we find that the related BET protein, BRD2, enforces HIV latency in the absence of Tat, pointing to a new target for BET inhibitor treatment in HIV infection. In shRNA-mediated knockdown experiments, knockdown of BRD2 activates HIV transcription to the same extent as JQ1 treatment, while a lesser effect is observed with BRD4. In single-cell time-lapse fluorescence microscopy, quantitative analyses across ~2,000 viral integration sites confirm the Tat-independent effect of JQ1 and point to positive effects of JQ1 on transcription elongation, while delaying re-initiation of the polymerase complex at the viral promoter. Collectively, our results identify BRD2 as a new Tat-independent suppressor of HIV transcription in latently infected cells and underscore the therapeutic potential of BET inhibitors in the reversal of HIV latency.
Related Concept Videos
 01:26
Size and Structure of Viral Genomes
 01:10
Retrovirus Life Cycles
 01:29
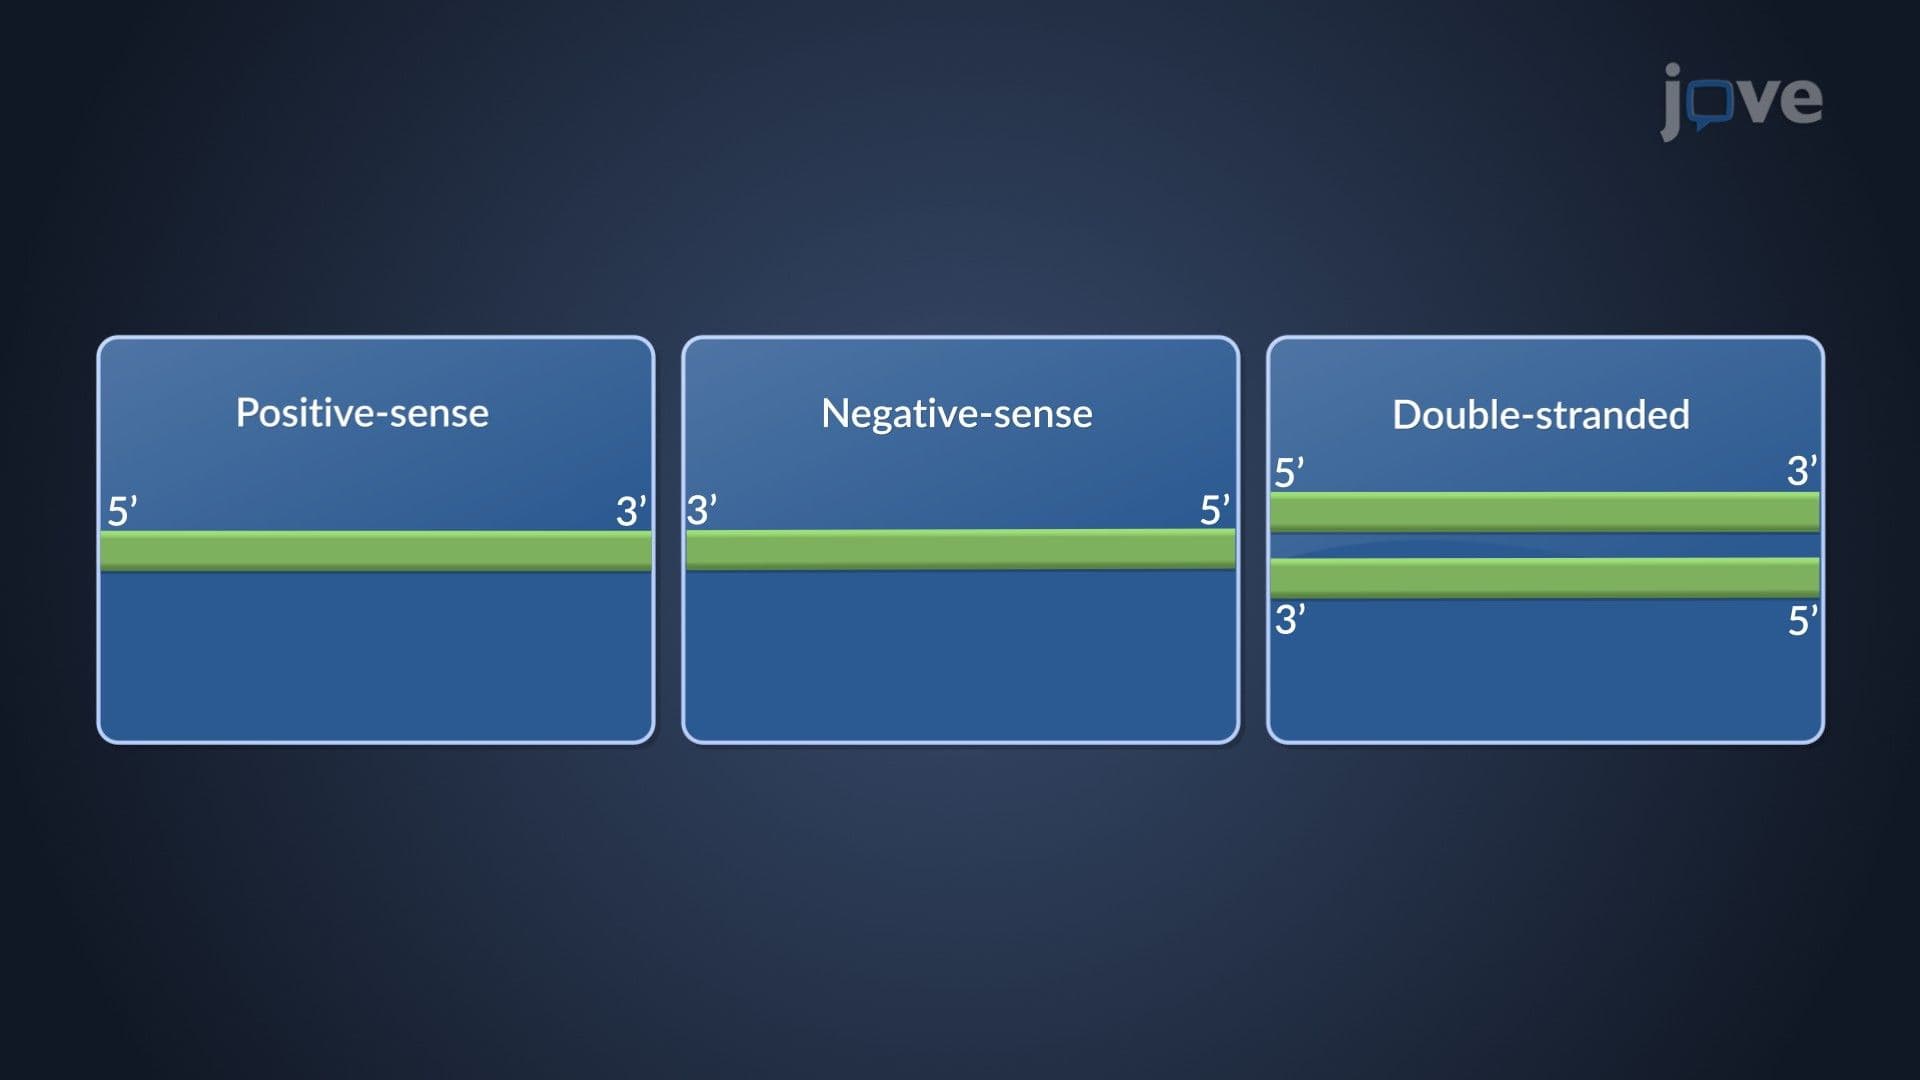
Viruses with RNA Genomes
 03:08
LTR Retrotransposons
The internal coding region of LTR retrotransposons and their mechanism of transposition closely resembles a...
 02:33
Retroviruses
 01:51
Mechanisms of Retrovirus-induced Cancers