Related Experiment Video
Updated: May 14, 2026
Chondrogenic Pellet Formation from Cord Blood-derived Induced Pluripotent Stem Cells
Published on: June 19, 2017
Hypertrophic differentiation during chondrogenic differentiation of progenitor cells is stimulated by BMP-2 but
M M J Caron1, P J Emans, A Cremers
1Department of Orthopaedic Surgery, Caphri School for Public Health and Primary Care, Maastricht University Medical Center, PO Box 5800, 6202 AZ, Maastricht, The Netherlands. marjolein.caron@maastrichtuniversity.nl

Objective:
Bone morphogenic protein (BMP)-2 and BMP-7 are clinically approved and their recombinant proteins are used for bone tissue regenerative purposes and widely evaluated for cartilage regeneration. Previous comparison of the in vitro chondrogenic characteristics of BMP-2 vs BMP-7 did not address hypertrophic differentiation and characterizing their chondrogenic properties with a focus in on chondrocyte hypertrophy was topic of investigation in this study.
Design:
Equimolar concentrations of BMP-2 or BMP-7 were added to chondrogenic differentiating ATDC5, human bone marrow stem cells or rabbit periosteal explants. Expression of Col2a1, Sox9, Acan, Col10a1, Runx2, ALP, Mmp13, Mef2c and Bapx1/Nkx3.2 was determined by reverse transcription-quantitative PCR (RT-qPCR) and immunoblotting. Glycosaminoglycan content, cell proliferation capacity and ALP activity were analysed by colourimetric analyses. Expression of Bapx1/Nkx3.2 and Sox9 was targeted by transfection of target specific siRNA duplexes.
Results:
BMP-2 dose-dependently increased chondrocyte hypertrophy during chondrogenic differentiation of progenitor cells, whereas BMP-7 acted hypertrophy-suppressive and chondro-promotive. Both BMPs did not influence cell proliferation, but they did increase total glycosaminoglycan content. In a candidate approach Bapx1/Nkx3.2 was found to be involved in the BMP-7 mediated suppression of chondrocyte hypertrophy in ATDC5 cells.
Conclusions:
BMP-2 and BMP-7 display opposing actions on the chondrogenic outcome of differentiating progenitor cells: BMP-2 acts a specific inducer of chondrocyte hypertrophy, while BMP-7 appears to increase or maintain chondrogenic potential and prevent chondrocyte hypertrophy. Our results pave the way for an application-dependent differential use of BMP-2 or BMP-7.
Related Concept Videos
 01:15
Differentiation of Common Myeloid Progenitor Cells
 01:27
Growth of Cartilage and Bone Tissue
 01:16
TGF - β Signaling Pathway
 01:24
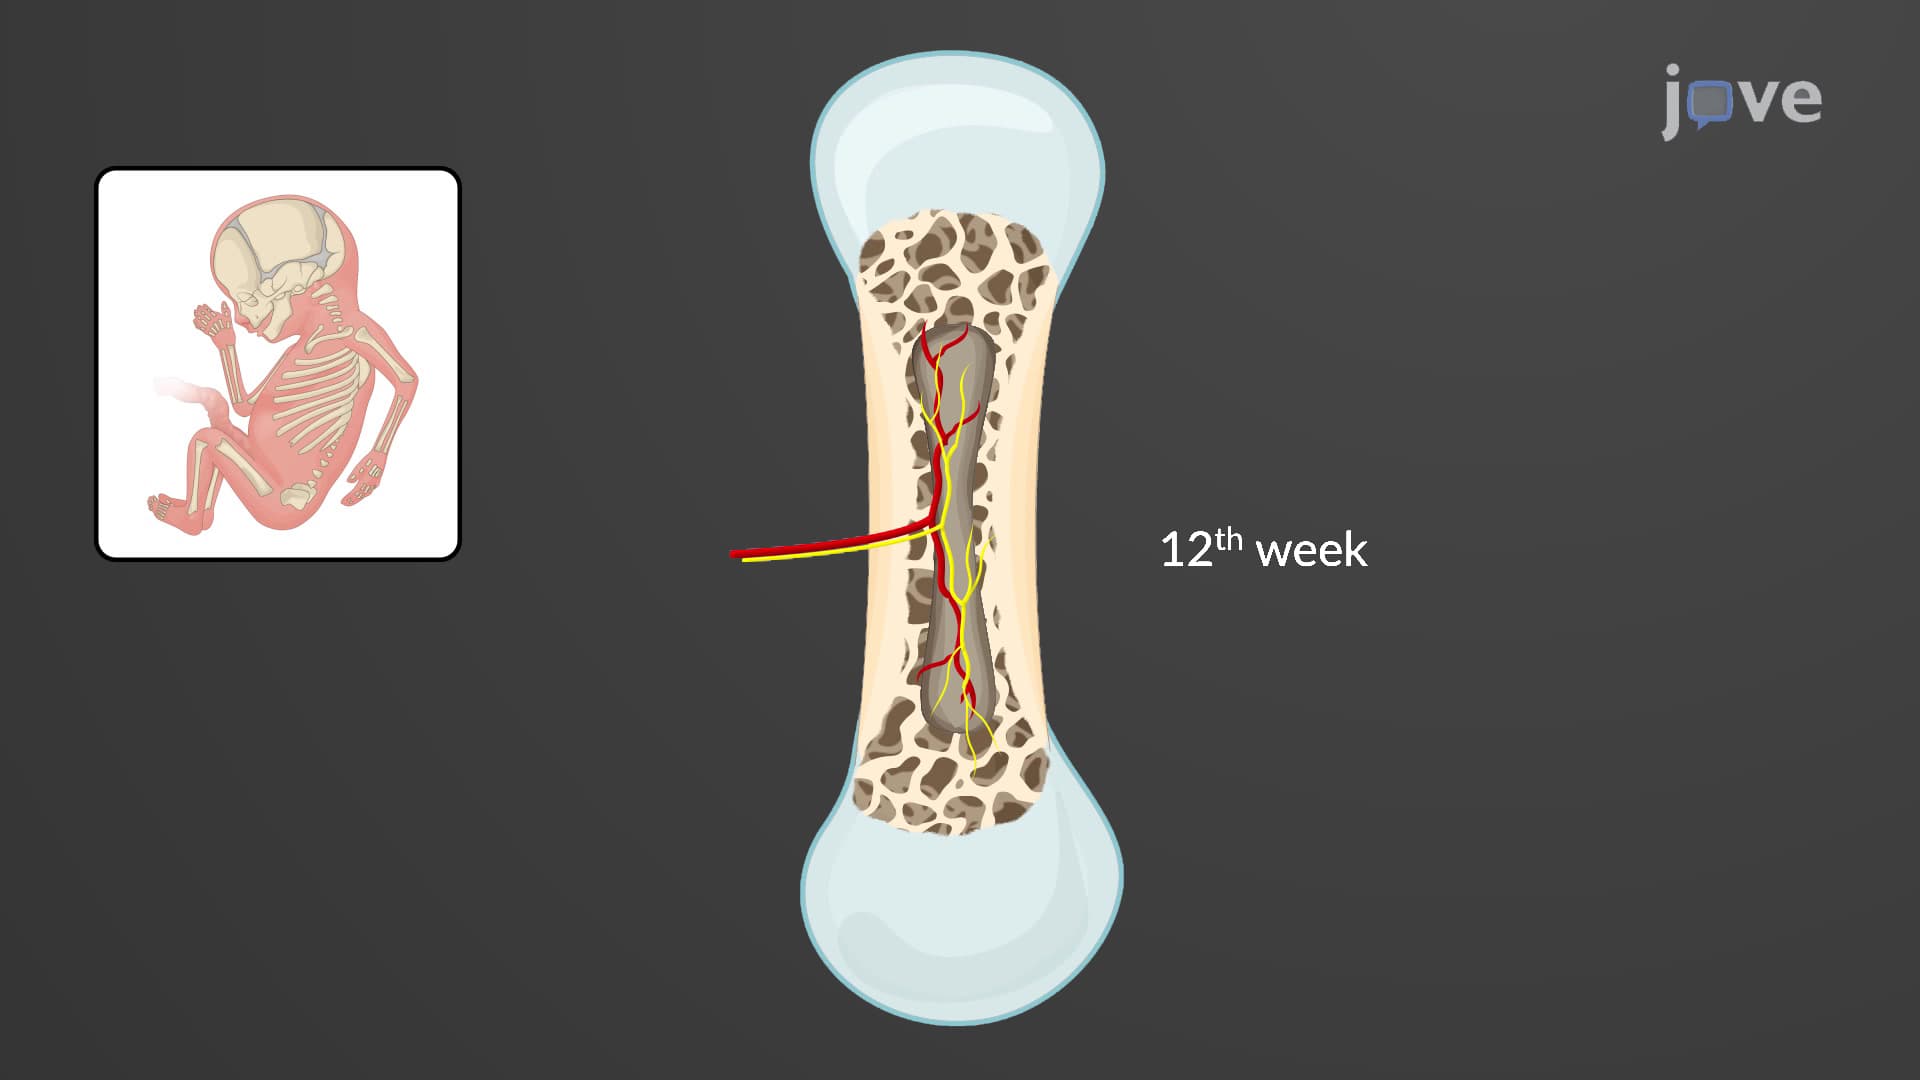
Bone Formation by Endochondral Ossification
 02:23
Master Transcription Regulators
 01:28
Forced Transdifferentiation
Artificial transdifferentiation occurs...