End-joining inhibition at telomeres requires the translocase and polySUMO-dependent ubiquitin ligase Uls1
Related Experiment Video
Updated: May 14, 2026
In Vitro Analysis of E3 Ubiquitin Ligase Function
Published on: May 14, 2021
Rachel Lescasse1, Sabrina Pobiega, Isabelle Callebaut
1CEA, Direction des sciences du vivant/Institut de radiobiologie cellulaire et moléculaire/Service instabilité génétique réparation recombinaison/Laboratoire télomère et réparation du chromosome, Fontenay-aux-roses, France.

Abstract:
In eukaryotes, permanent inhibition of the non-homologous end joining (NHEJ) repair pathway at telomeres ensures that chromosome ends do not fuse. In budding yeast, binding of Rap1 to telomere repeats establishes NHEJ inhibition. Here, we show that the Uls1 protein is required for the maintenance of NHEJ inhibition at telomeres. Uls1 protein is a non-essential Swi2/Snf2-related translocase and a Small Ubiquitin-related Modifier (SUMO)-Targeted Ubiquitin Ligase (STUbL) with unknown targets. Loss of Uls1 results in telomere-telomere fusions. Uls1 requirement is alleviated by the absence of poly-SUMO chains and by rap1 alleles lacking SUMOylation sites. Furthermore, Uls1 limits the accumulation of Rap1 poly-SUMO conjugates. We propose that one of Uls1 functions is to clear non-functional poly-SUMOylated Rap1 molecules from telomeres to ensure the continuous efficiency of NHEJ inhibition. Since Uls1 is the only known STUbL with a translocase activity, it can be the general molecular sweeper for the clearance of poly-SUMOylated proteins on DNA in eukaryotes.
Related Concept Videos
 02:41
Telomeres and Telomerase
02:41Telomeres and Telomerase
 02:10
Translesion DNA Polymerases
TLS polymerases are found in all three domains of life - archaea, bacteria, and eukaryotes. Of the different classes of TLS polymerases, members of the Y family are fitted with specialized structures that...
 01:28
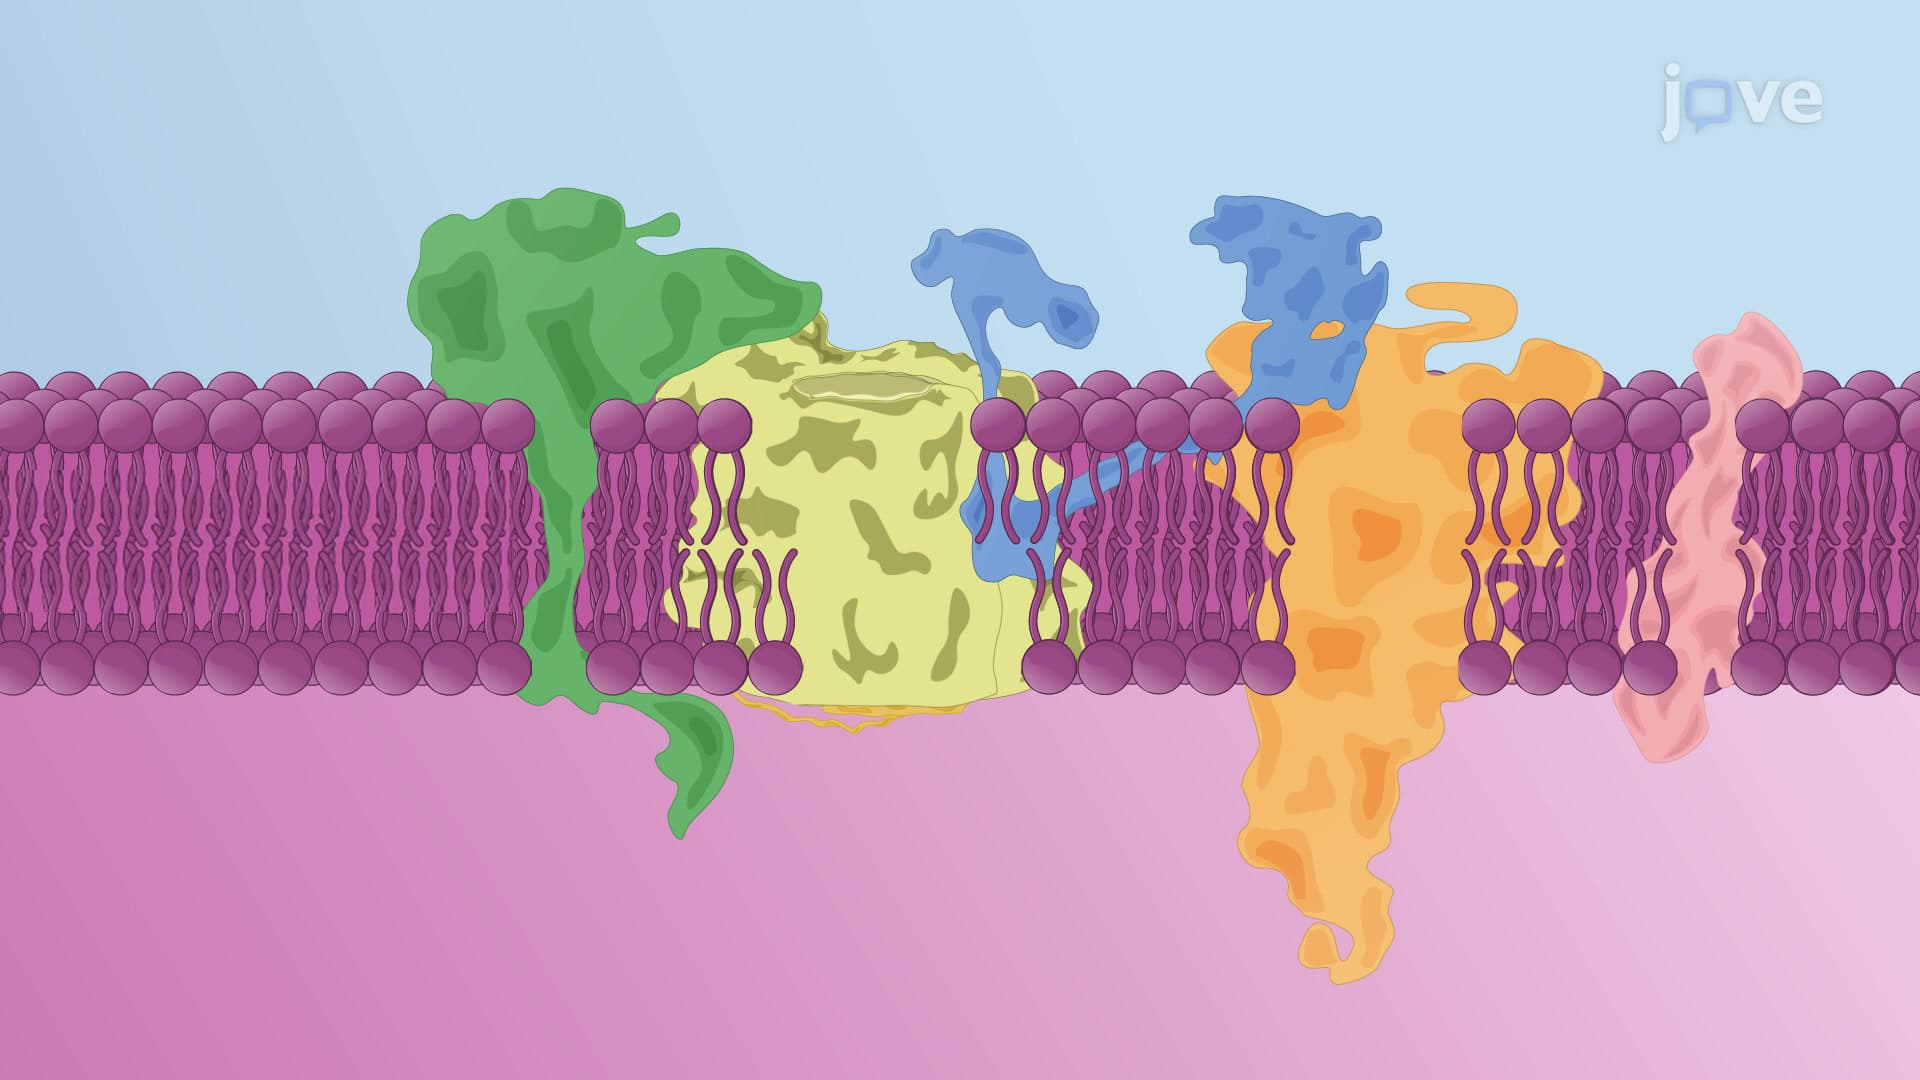
Protein Translocation Machinery on the ER Membrane
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the translocon complex.
 00:50
Anaphase Promoting Complex
 01:38
Intralumenal Vesicles and Multivesicular Bodies