Related Experiment Video
Updated: May 13, 2026

Optimized Protocol for the Extraction of Proteins from the Human Mitral Valve
Published on: June 14, 2017
Structure of the N-terminal domain of human thioredoxin-interacting protein
Galina Polekhina1, David Benjamin Ascher, Shie Foong Kok
1Centre for Cancer Research, Monash Institute of Medical Research, Monash University, 27-31 Wright Street, Clayton, VIC 3168, Australia. galina.polekhina@monash.edu

Abstract:
Thioredoxin-interacting protein (TXNIP) is one of the six known α-arrestins and has recently received considerable attention owing to its involvement in redox signalling and metabolism. Various stress stimuli such as high glucose, heat shock, UV, H2O2 and mechanical stress among others robustly induce the expression of TXNIP, resulting in the sequestration and inactivation of thioredoxin, which in turn leads to cellular oxidative stress. While TXNIP is the only α-arrestin known to bind thioredoxin, TXNIP and two other α-arrestins, Arrdc4 and Arrdc3, have been implicated in metabolism. Furthermore, owing to its roles in the pathologies of diabetes and cardiovascular disease, TXNIP is considered to be a promising drug target. Based on their amino-acid sequences, TXNIP and the other α-arrestins are remotely related to β-arrestins. Here, the crystal structure of the N-terminal domain of TXNIP is reported. It provides the first structural information on any of the α-arrestins and reveals that although TXNIP adopts a β-arrestin fold as predicted, it is structurally more similar to Vps26 proteins than to β-arrestins, while sharing below 15% pairwise sequence identity with either.
Related Concept Videos
 01:26
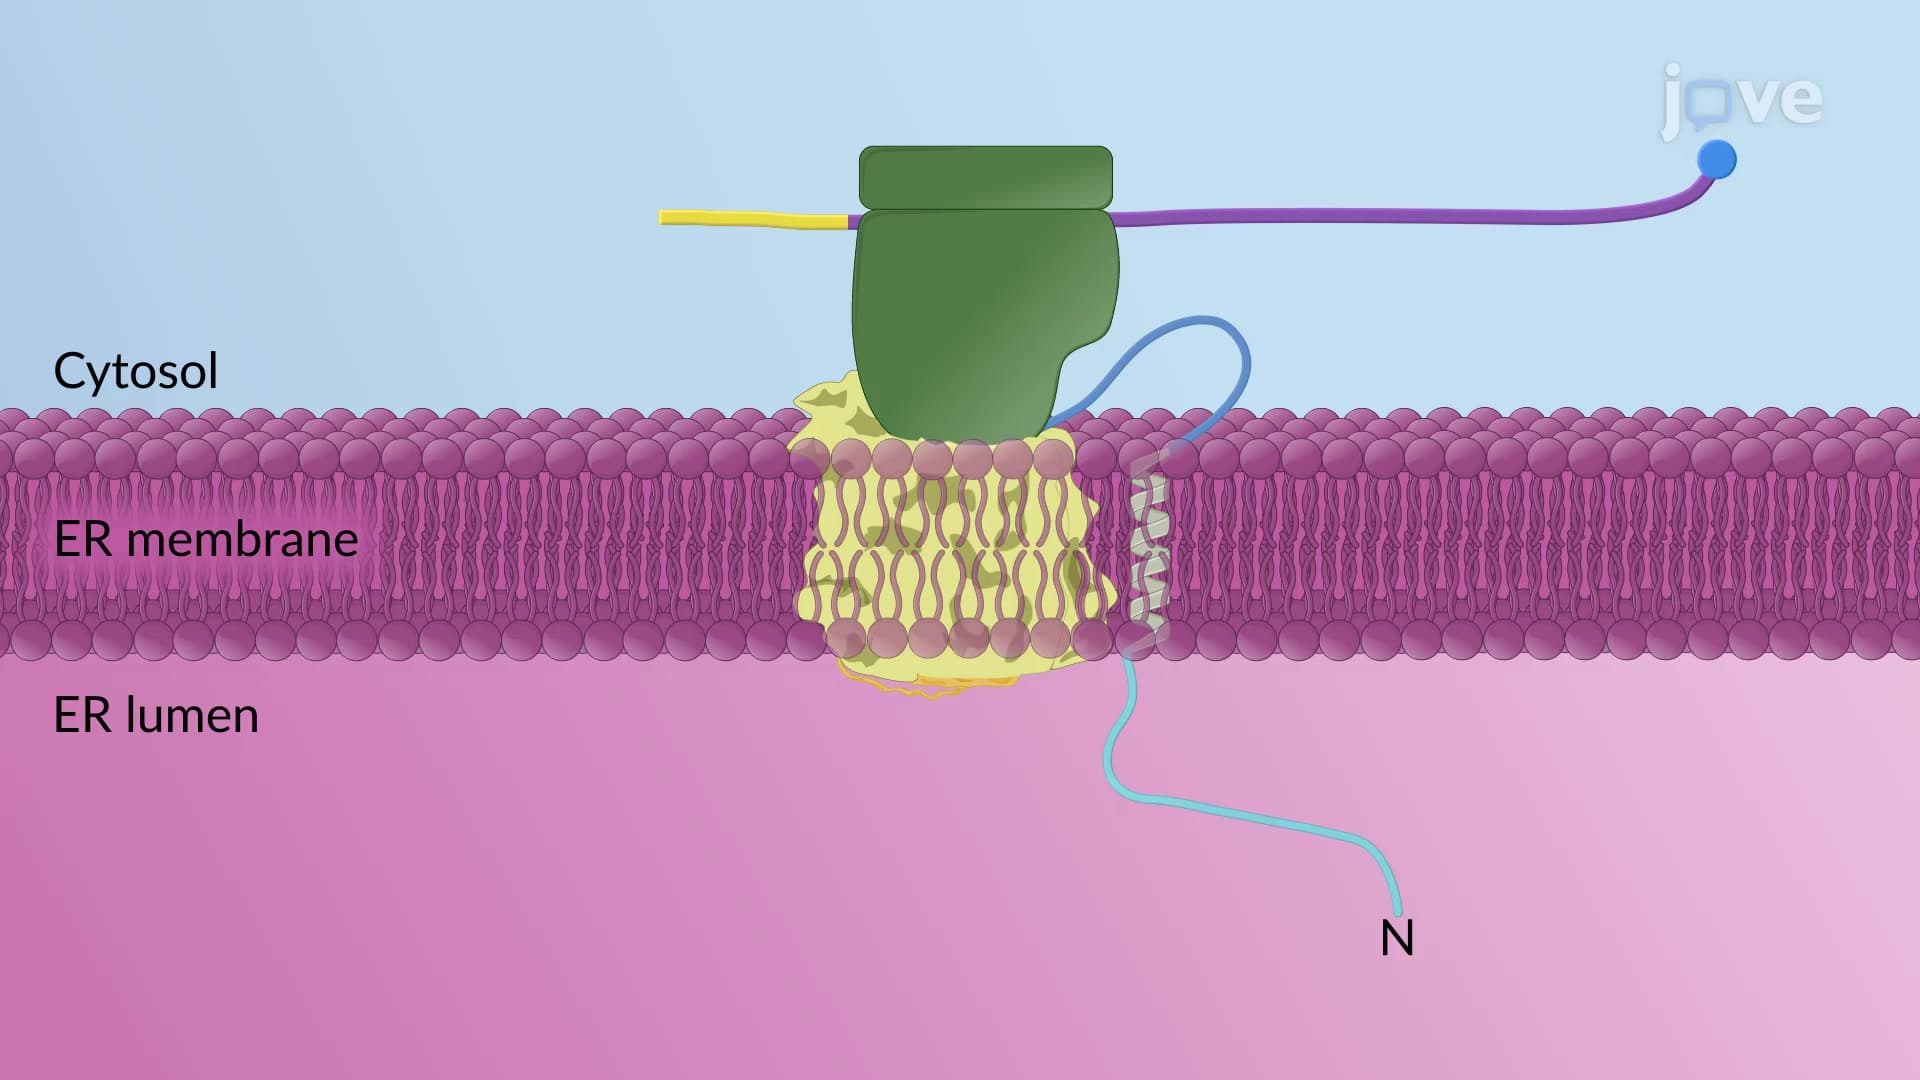
Insertion of Single-pass Transmembrane Proteins in the RER
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
 01:19
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 02:26
Conservation of Protein Domains Over Different Proteins
A limited set of protein domains often duplicate and recombine during evolution. These domains can be organized in different combinations to form...
 01:34
Protein Transport into the Inner Mitochondrial Membrane
Transport of mitochondrial precursors across the TIM23 channel is driven by...
 01:39
Mitochondrial Precursor Proteins
Most of the mitochondrial precursors...
 01:21
Structure of Porins