Related Experiment Video
Updated: May 11, 2026

Detergent-free Ultrafast Reconstitution of Membrane Proteins into Lipid Bilayers Using Fusogenic Complementary-charged Proteoliposomes.
Published on: April 5, 2018
Membrane fusion-competent virus-like proteoliposomes and proteinaceous supported bilayers made directly from cell
Deirdre A Costello1, Chih-Yun Hsia, Jean K Millet
1School of Chemical and Biomolecular Engineering, Cornell University, Ithaca, New York, USA.

Abstract:
Virus-like particles are useful materials for studying virus-host interactions in a safe manner. However, the standard production of pseudovirus based on the vesicular stomatitis virus (VSV) backbone is an intricate procedure that requires trained laboratory personnel. In this work, a new strategy for creating virus-like proteoliposomes (VLPLs) and virus-like supported bilayers (VLSBs) is presented. This strategy uses a cell blebbing technique to induce the formation of nanoscale vesicles from the plasma membrane of BHK cells expressing the hemagglutinin (HA) fusion protein of influenza X-31. These vesicles and supported bilayers contain HA and are used to carry out single particle membrane fusion events, monitored using total internal reflection fluorescence microscopy. The results of these studies show that the VLPLs and VLSBs contain HA proteins that are fully competent to carry out membrane fusion, including the formation of a fusion pore and the release of fluorophores loaded into vesicles. This new strategy for creating spherical and planar geometry virus-like membranes has many potential applications. VLPLs could be used to study fusion proteins of virulent viruses in a safe manner, or they could be used as therapeutic delivery particles to transport beneficial proteins coexpressed in the cells to a target cell. VLSBs could facilitate high throughput screening of antiviral drugs or pathogen-host cell interactions.
More Related Videos
Related Concept Videos
 01:43
SNAREs and Membrane Fusion
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
 01:26
Fusion of Secretory Vesicles with the Plasma Membrane
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
 01:19
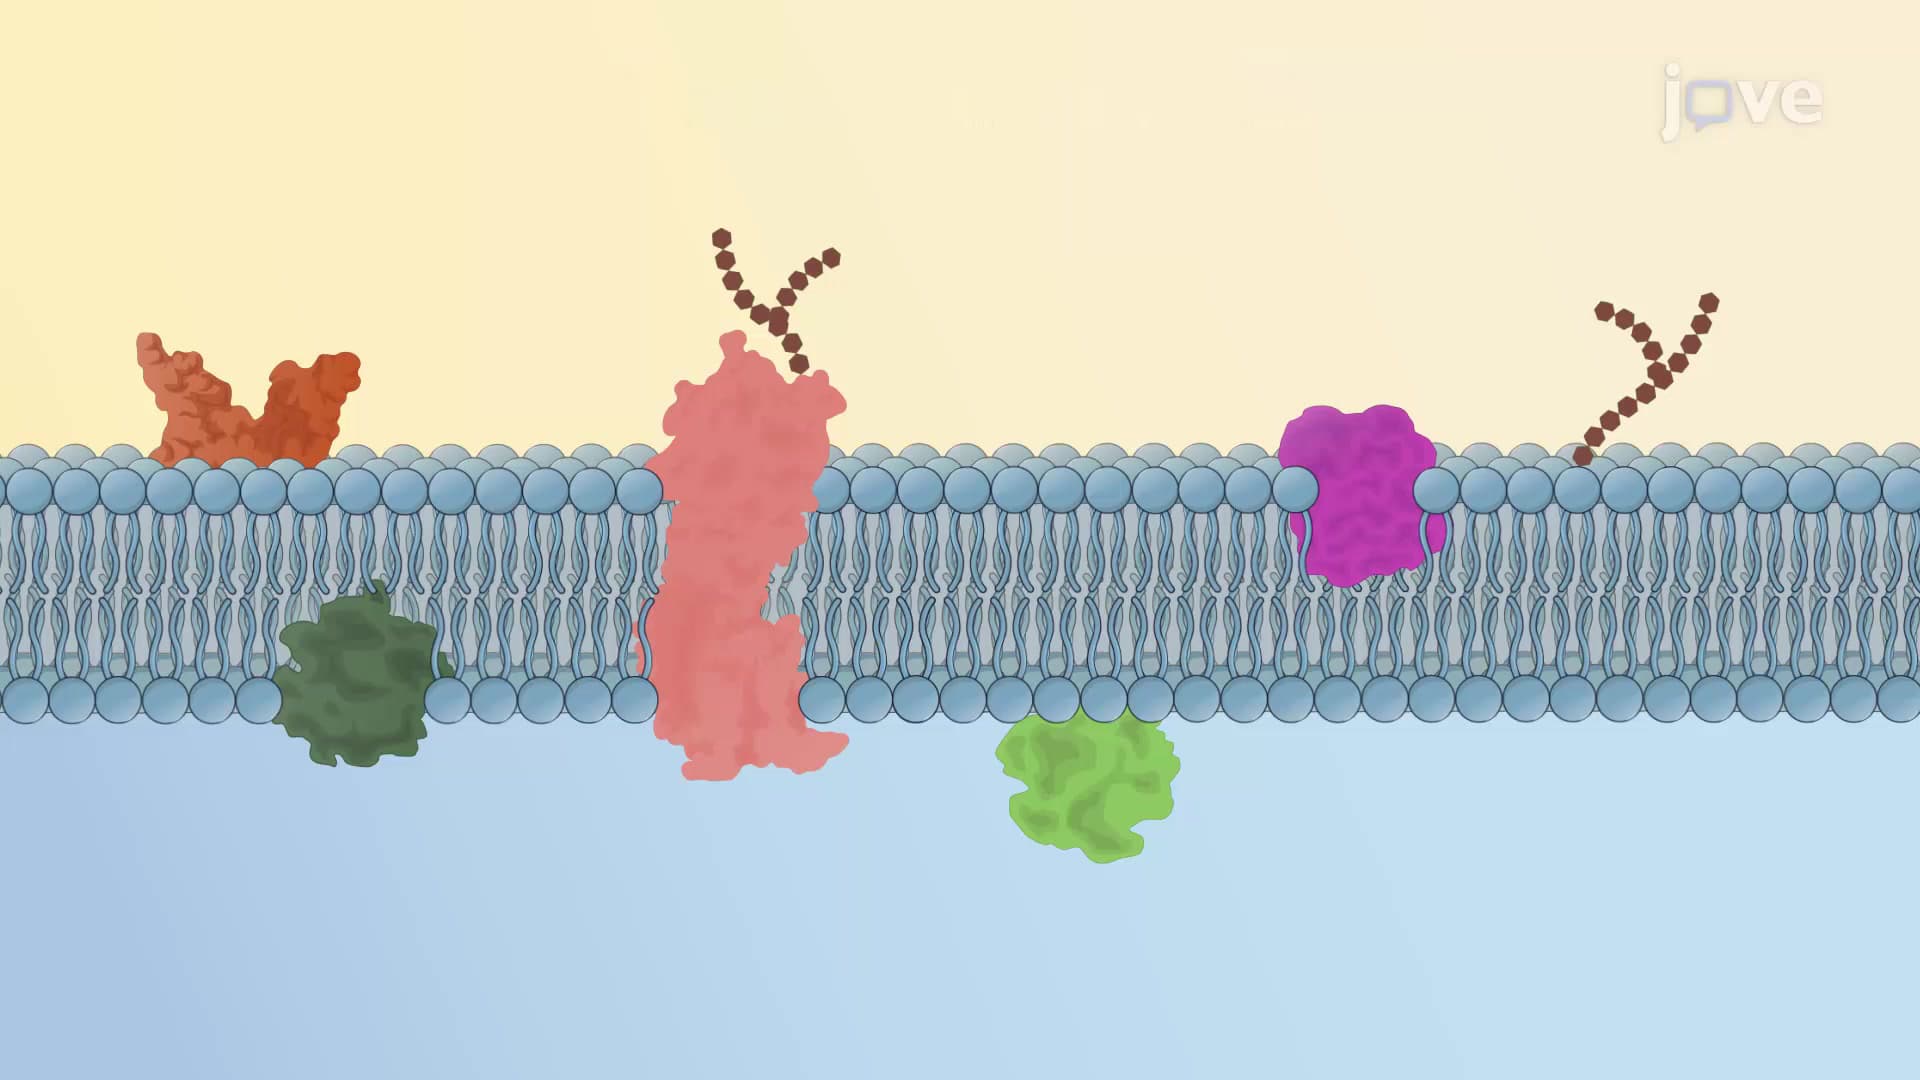
Fluid Mosaic Model
 00:59
Mechanisms of Membrane Domain Formation
Another mechanism for membrane domain formation involves membrane proteins interacting with cytoskeletal...
 01:38
Intralumenal Vesicles and Multivesicular Bodies
 01:26
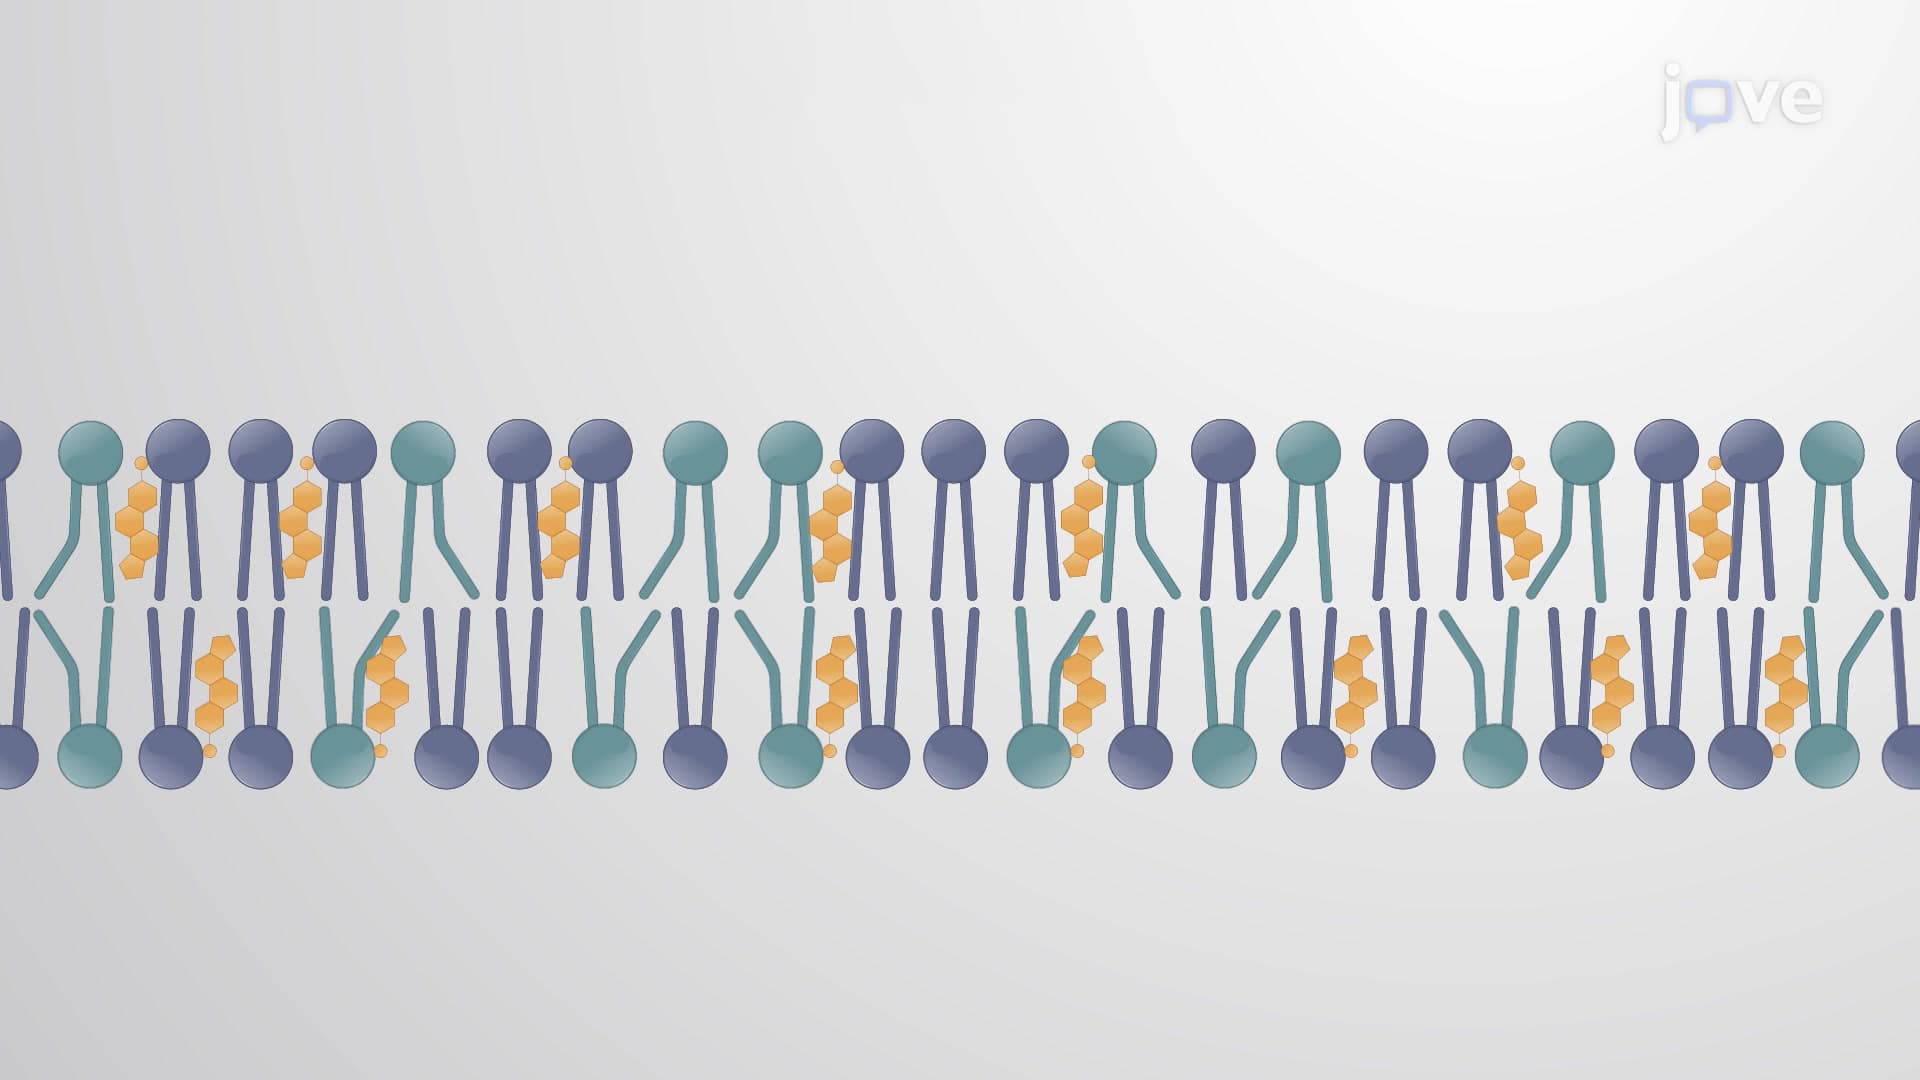
Membrane Fluidity
Mosaic nature of the membrane
The mosaic characteristic of the membrane helps the plasma membrane remain fluid. The integral proteins and lipids exist as separate but loosely-attached molecules in the membrane. The membrane is a relatively...