Related Experiment Video
Updated: May 11, 2026
Arabidopsis thaliana Polar Glycerolipid Profiling by Thin Layer Chromatography (TLC) Coupled with Gas-Liquid Chromatography (GLC)
Published on: March 18, 2011
Golgi traffic and integrity depend on N-myristoyl transferase-1 in Arabidopsis
Luciana Renna1, Giovanni Stefano, Wojciech Majeran
1Michigan State University-Department of Energy Plant Research Lab, Michigan State University, East Lansing, Michigan 48824, USA.

Abstract:
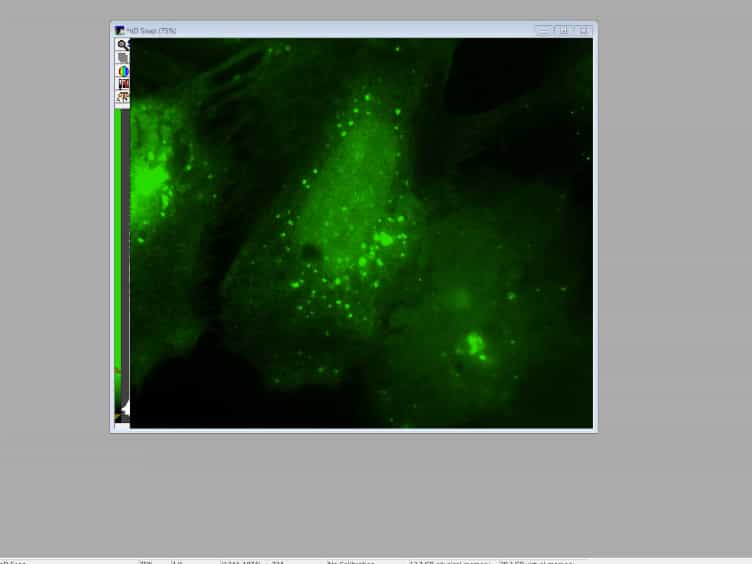
N-myristoylation is a crucial irreversible eukaryotic lipid modification allowing a key subset of proteins to be targeted at the periphery of specific membrane compartments. Eukaryotes have conserved N-myristoylation enzymes, involving one or two N-myristoyltransferases (NMT1 and NMT2), among which NMT1 is the major enzyme. In the postembryonic developmental stages, defects in NMT1 lead to aberrant cell polarity, flower differentiation, fruit maturation, and innate immunity; however, no specific NMT1 target responsible for such deficiencies has hitherto been identified. Using a confocal microscopy forward genetics screen for the identification of Arabidopsis thaliana secretory mutants, we isolated STINGY, a recessive mutant with defective Golgi traffic and integrity. We mapped STINGY to a substitution at position 160 of Arabidopsis NMT1 (NMT1A160T). In vitro kinetic studies with purified NMT1A160T enzyme revealed a significant reduction in its activity due to a remarkable decrease in affinity for both myristoyl-CoA and peptide substrates. We show here that this recessive mutation is responsible for the alteration of Golgi traffic and integrity by predominantly affecting the Golgi membrane/cytosol partitioning of ADP-ribosylation factor proteins. Our results provide important functional insight into N-myristoylation in plants by ascribing postembryonic functions of Arabidopsis NMT1 that involve regulation of the functional and morphological integrity of the plant endomembranes.
Related Concept Videos
 01:26
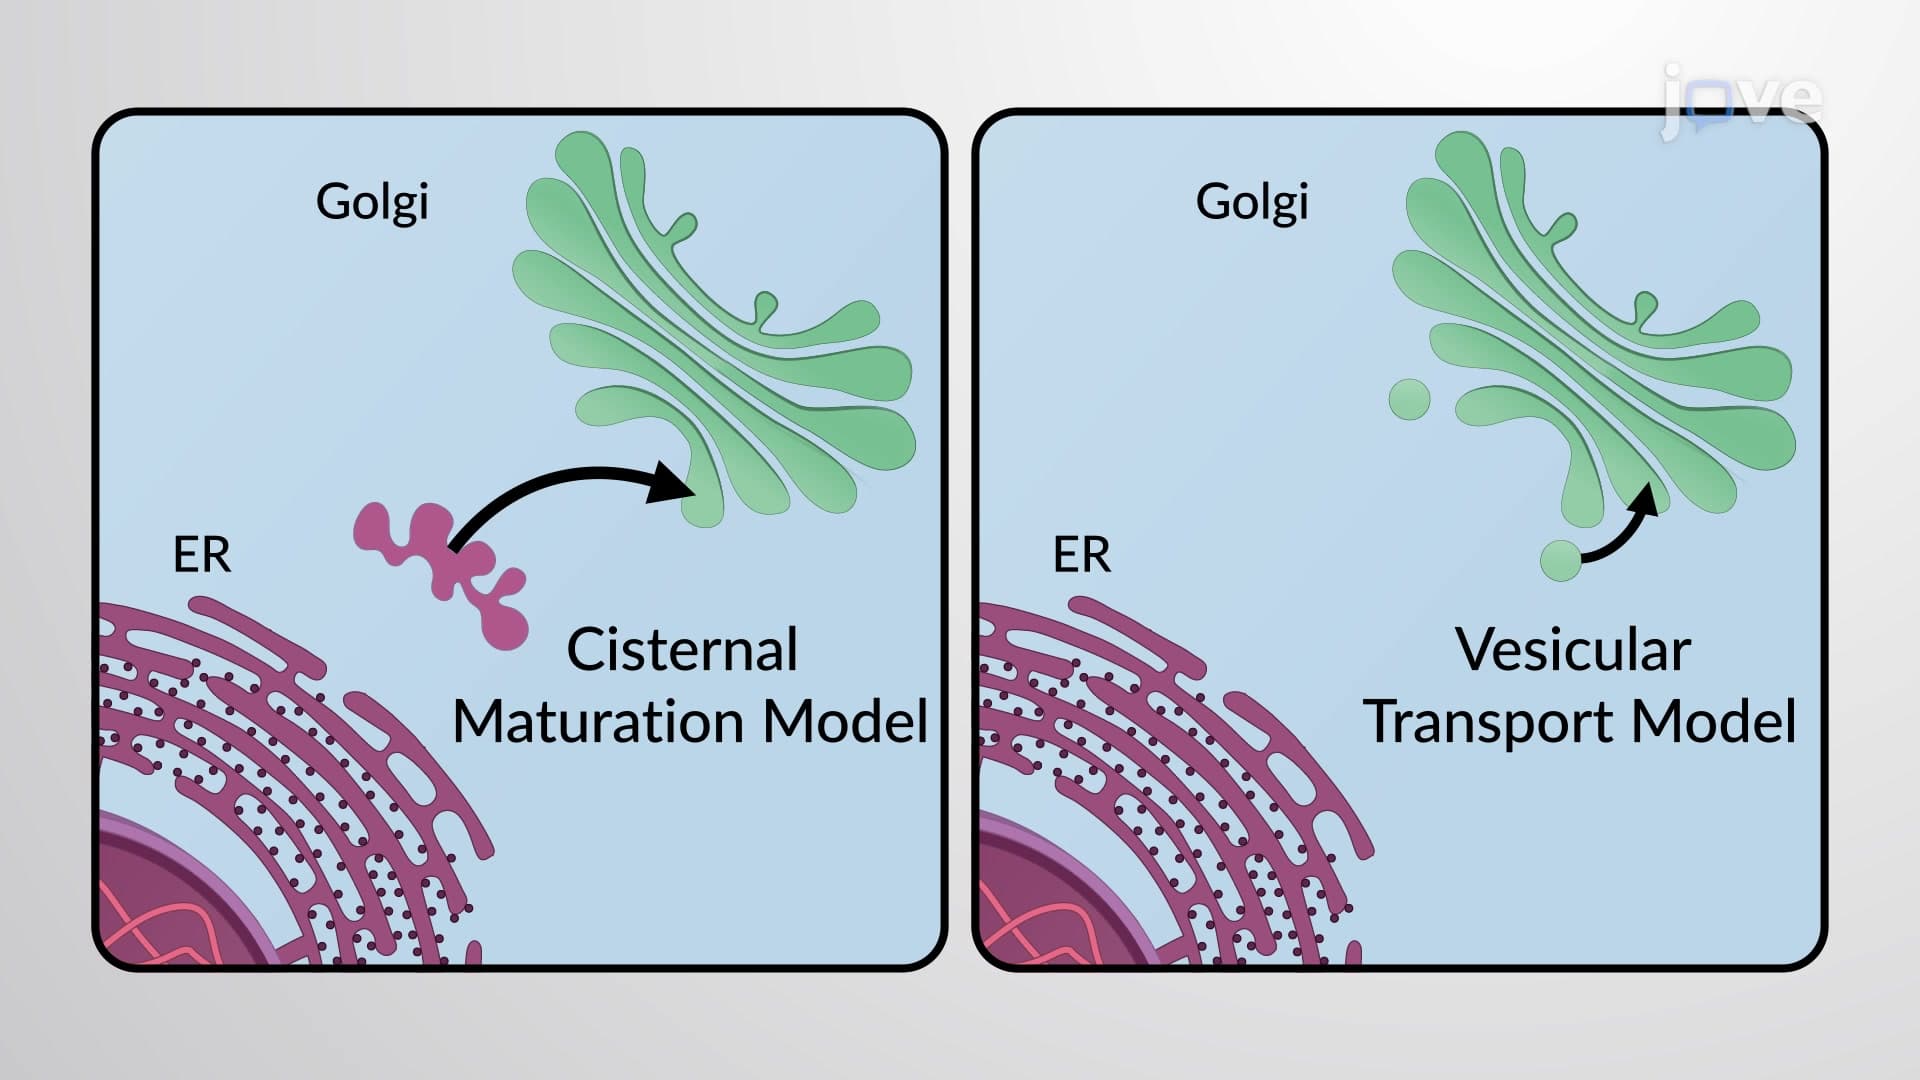
Transport Across the Golgi
 01:45
Tail-anchoring of Proteins in the ER Membrane
 01:11
Protein Transport to the Outer Chloroplast Membrane
Two models describe the mechanism of precursor recognition and entry across the outer membrane through the TOC complex. Model 1 suggests the newly synthesized precursor binds to the TOC receptor 159 and forms a complex.
 01:18
Protein Transport to the Inner Chloroplast Membrane
 01:12
Golgi Matrix Proteins
One of the first identified Golgi matrix proteins was GM130, a rod-like protein located in the cis-Golgi. Subsequently, many Golgi...
 01:20
Cotranslational Protein Translocation
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...