Related Experiment Video
Updated: May 8, 2026

Biotinylated Cell-penetrating Peptides to Study Intracellular Protein-protein Interactions
Published on: December 20, 2017
Effect of Janus kinase 3 on the peptide transporters PEPT1 and PEPT2
Jamshed Warsi1, Zohreh Hosseinzadeh, Luo Dong
1Department of Physiology I, University of Tübingen, Gmelinstr. 5, 72076, Tübingen, Germany.

The tyrosine kinase Janus kinase 3 (JAK3) contributes to signaling regulating the proliferation and apoptosis of lymphocytes and tumor cells. Replacement of lysine by alanine in the catalytic subunit yields the inactive (K851A)JAK3 mutant that underlies severe combined immune deficiency. The gain-of-function mutation (A572V)JAK3 is found in acute megakaryoplastic leukemia and T cell lymphoma. The excessive nutrient demand of tumor cells requires upregulation of transporters in the cell membrane including peptide transporters PEPT1 and PEPT2. The carriers further accomplish intestinal peptide transport. Little is known about signaling regulating peptide transport. The present study explored whether PEPT1 and PEPT2 are upregulated by JAK3. PEPT1 or PEPT2 was expressed in Xenopus oocytes with or without additional expression of JAK3, and electrogenic peptide (glycine-glycine) transport was determined by dual-electrode voltage clamp. PEPT2-HA membrane protein abundance was analyzed by chemiluminescence. Intestinal electrogenic peptide transport was estimated from peptide-induced current in Ussing chamber experiments. In PEPT1- and PEPT2-expressing oocytes, but not in water-injected oocytes, the dipeptide gly-gly generated an inward current, which was significantly increased following coexpression of JAK3. The effect of JAK3 on PEPT1 was mimicked by (A568V)JAK3 but not by (K851A)JAK3. JAK3 increased maximal peptide-induced current in PEPT1-expressing oocytes but rather decreased apparent affinity of the carrier. Coexpression of JAK3 enhanced the PEPT2-HA protein abundance in the cell membrane. In JAK3- and PEPT1-expressing oocytes, peptide-induced current was blunted by the JAK3 inhibitor WHI-P154, 4-[(3'-bromo-4'-hydroxyphenyl)amino]-6,7-dimethoxyquinazoline (22 μM). In intestinal segments gly-gly generated a current which was significantly smaller in JAK3-deficient mice (jak3⁻/⁻) than in wild-type mice (jak3⁺/⁺). In conclusion, JAK3 is a powerful regulator of peptide transporters PEPT1 and PEPT2.
The tyrosine kinase Janus kinase 3 (JAK3) contributes to signaling regulating the proliferation and apoptosis of lymphocytes and tumor cells. Replacement of lysine by alanine in the catalytic subunit yields the inactive (K851A)JAK3 mutant that underlies severe combined immune deficiency. The gain-of-function mutation (A572V)JAK3 is found in acute megakaryoplastic leukemia and T cell lymphoma. The excessive nutrient demand of tumor cells requires upregulation of transporters in the cell membrane including peptide transporters PEPT1 and PEPT2. The carriers further accomplish intestinal peptide transport. Little is known about signaling regulating peptide transport. The present study explored whether PEPT1 and PEPT2 are upregulated by JAK3. PEPT1 or PEPT2 was expressed in Xenopus oocytes with or without additional expression of JAK3, and electrogenic peptide (glycine-glycine) transport was determined by dual-electrode voltage clamp. PEPT2-HA membrane protein abundance was analyzed by chemiluminescence. Intestinal electrogenic peptide transport was estimated from peptide-induced current in Ussing chamber experiments. In PEPT1- and PEPT2-expressing oocytes, but not in water-injected oocytes, the dipeptide gly-gly generated an inward current, which was significantly increased following coexpression of JAK3. The effect of JAK3 on PEPT1 was mimicked by (A568V)JAK3 but not by (K851A)JAK3. JAK3 increased maximal peptide-induced current in PEPT1-expressing oocytes but rather decreased apparent affinity of the carrier. Coexpression of JAK3 enhanced the PEPT2-HA protein abundance in the cell membrane. In JAK3- and PEPT1-expressing oocytes, peptide-induced current was blunted by the JAK3 inhibitor WHI-P154, 4-[(3'-bromo-4'-hydroxyphenyl)amino]-6,7-dimethoxyquinazoline (22 μM). In intestinal segments gly-gly generated a current which was significantly smaller in JAK3-deficient mice (jak3⁻/⁻) than in wild-type mice (jak3⁺/⁺). In conclusion, JAK3 is a powerful regulator of peptide transporters PEPT1 and PEPT2.
Related Concept Videos
 01:20
The JAK-STAT Signaling Pathway
 01:19
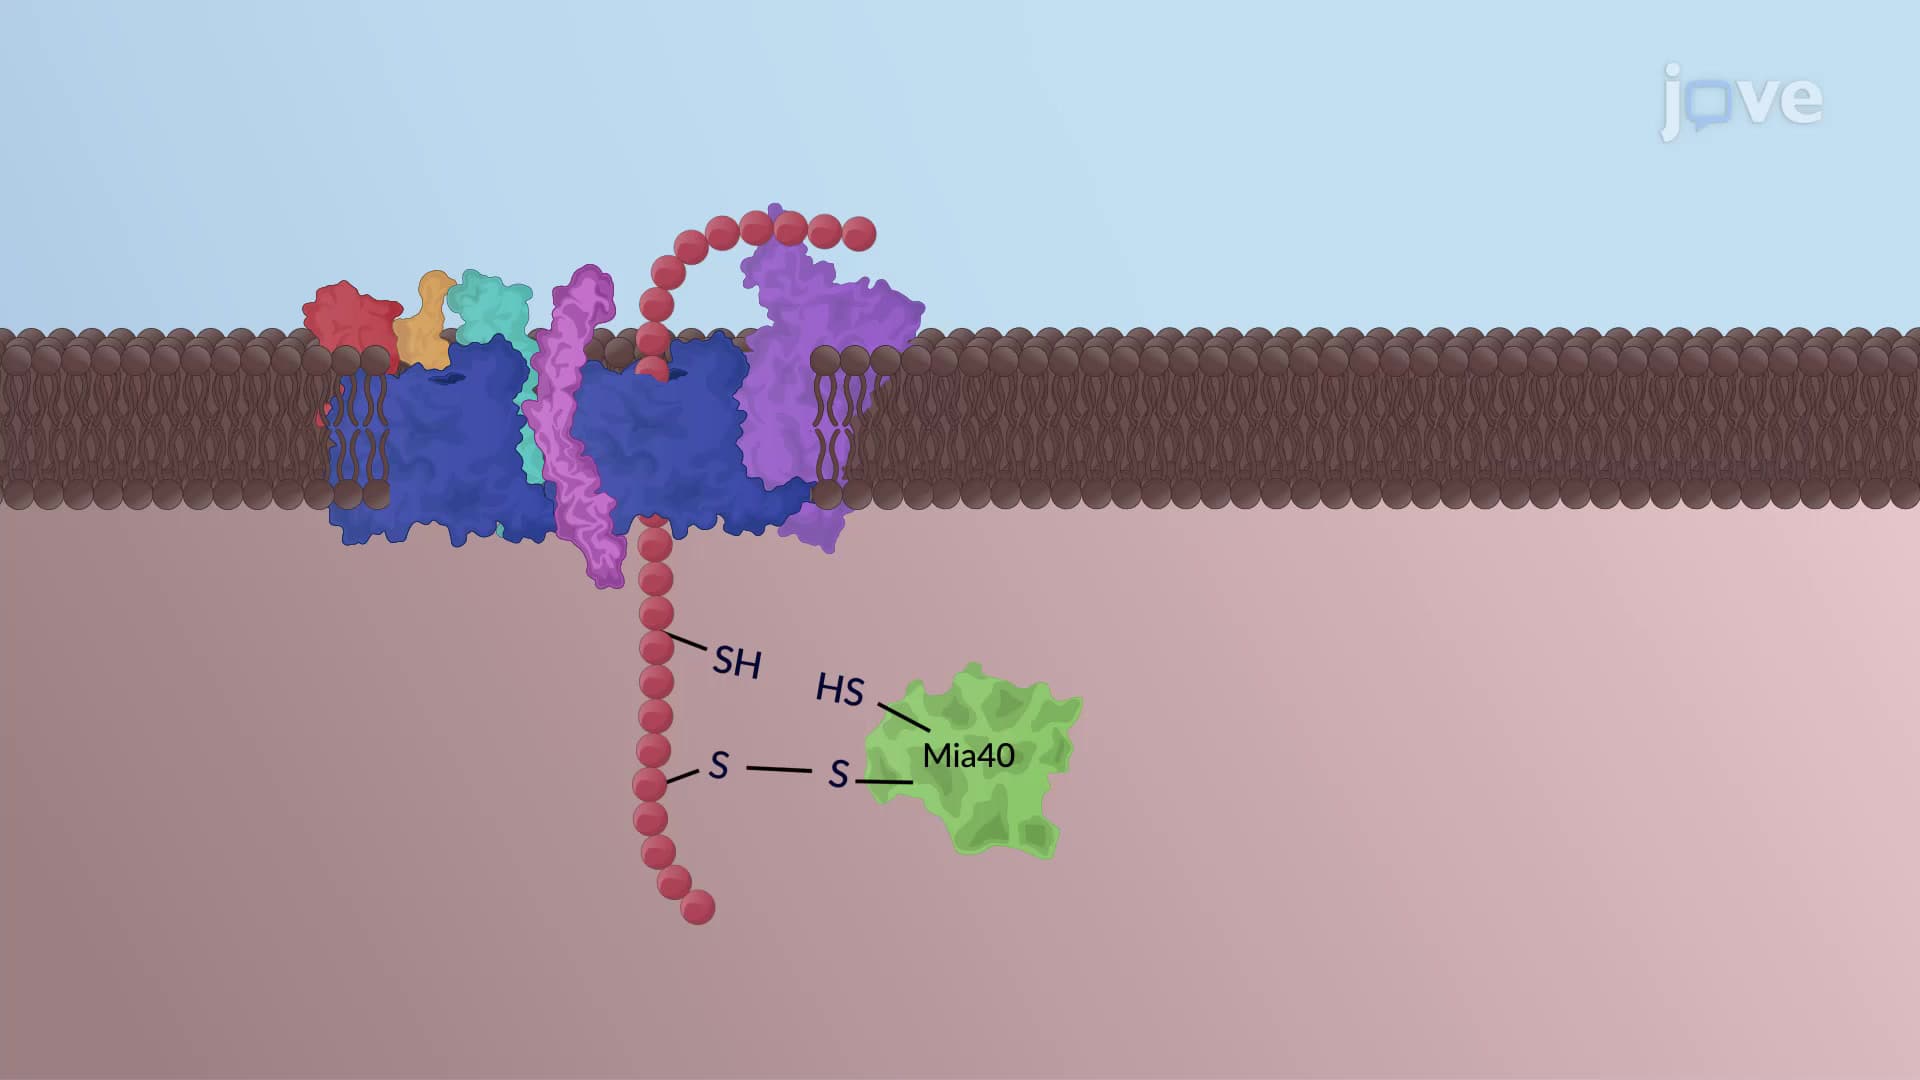
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:06
Carrier-Mediated Transport
Active transport involves two types of membrane-spanning transporters: uptake and efflux. Uptake transporters are expressed in the small...
 01:45
Regulation of Nuclear Protein Sorting
 01:34
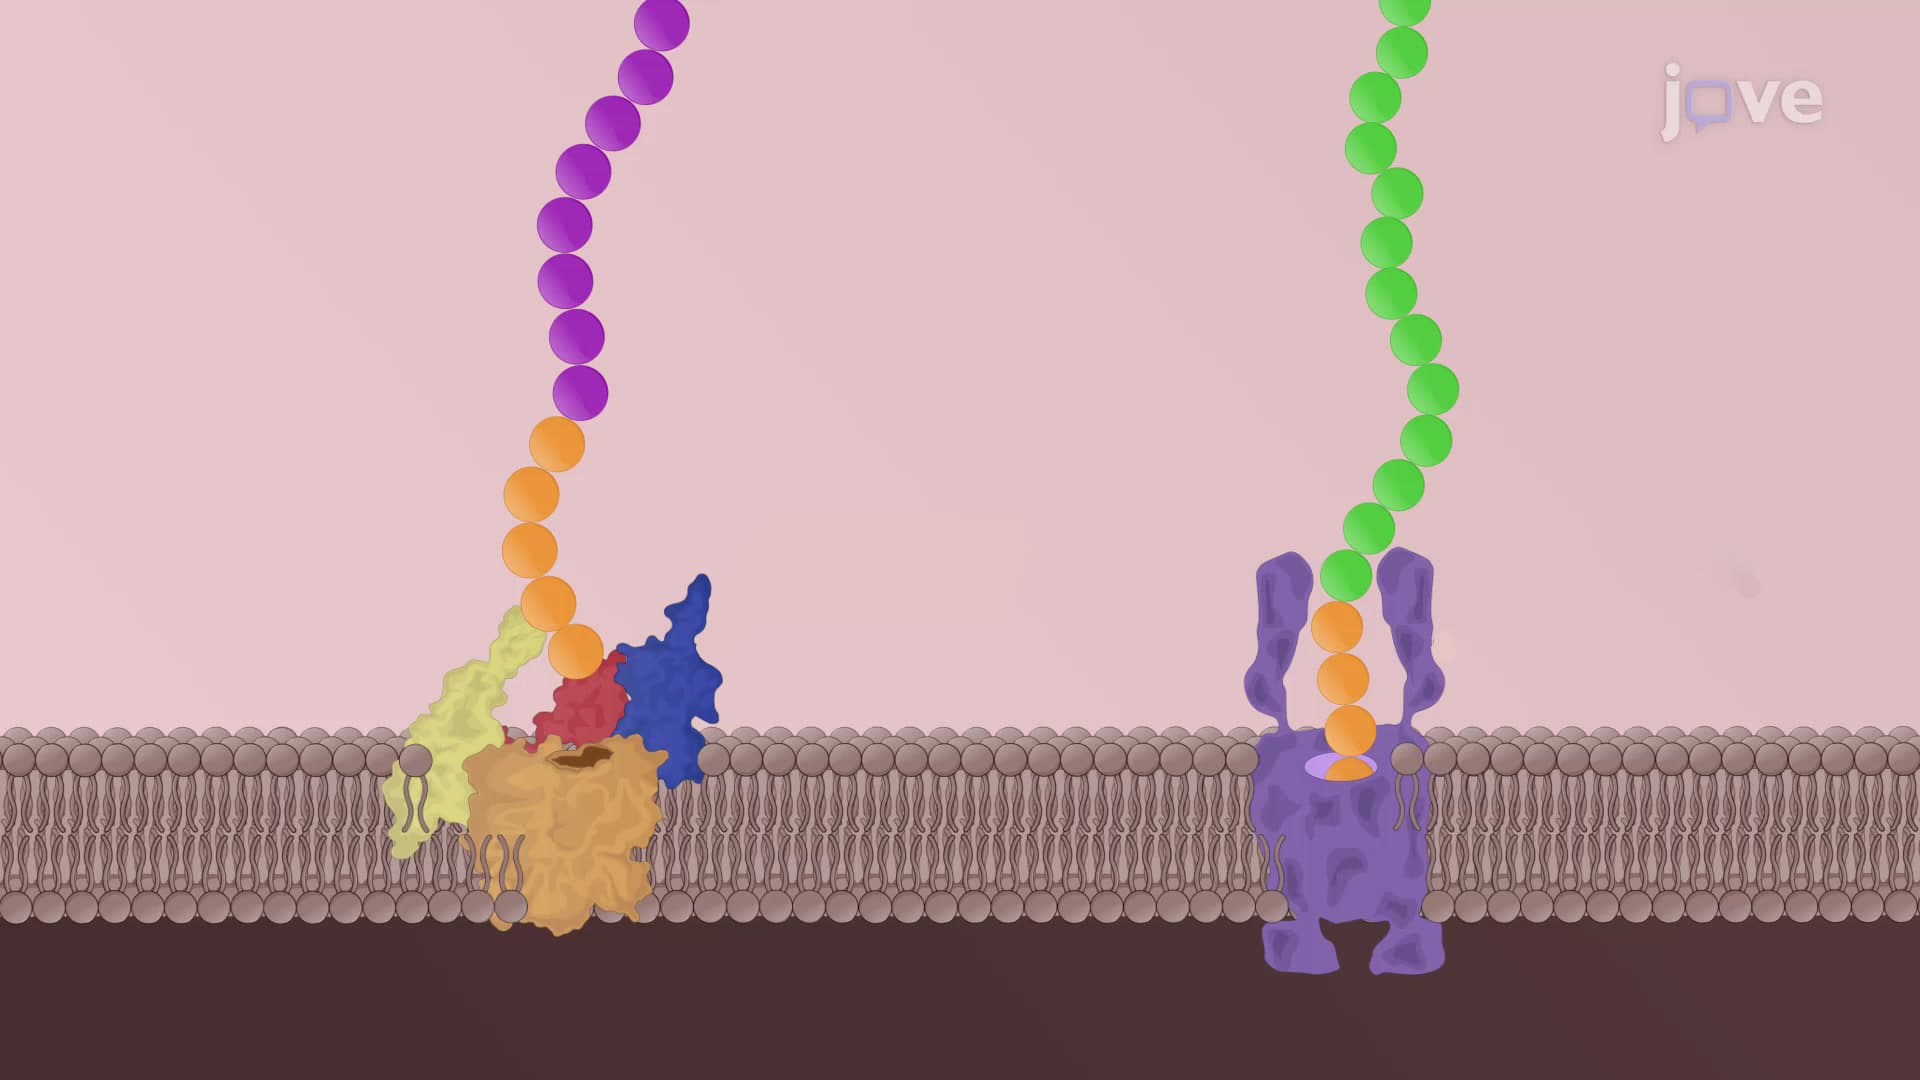
Protein Transport into the Inner Mitochondrial Membrane
Transport of mitochondrial precursors across the TIM23 channel is driven by...
 01:19
Membrane Asymmetry Regulating Transporters
Flippase
Eukaryotic flippases are type-IV P-type ATPases or P4-ATPases belonging to P-type ATPase family proteins that are membrane-bound pumps involved in the ATP-mediated transport of ions and molecules across the membrane. Flippases flip specific phospholipids from the outer to the inner leaflet of a membrane. All P4-ATPases have one...