Related Experiment Video
Updated: May 6, 2026
A Direct Force Probe for Measuring Mechanical Integration Between the Nucleus and the Cytoskeleton
Published on: July 29, 2018
Cohesiveness tunes assembly and morphology of FG nucleoporin domain meshworks - Implications for nuclear pore
Nico B Eisele1, Aksana A Labokha, Steffen Frey
1Biosurfaces Unit, CIC biomaGUNE, San Sebastian, Spain; Department of Cellular Logistics, Max Planck Institute for Biophysical Chemistry, Göttingen, Germany.

Abstract:
Nuclear pore complexes control the exchange of macromolecules between the cytoplasm and the nucleus. A selective permeability barrier that arises from a supramolecular assembly of intrinsically unfolded nucleoporin domains rich in phenylalanine-glycine dipeptides (FG domains) fills the nuclear pore. There is increasing evidence that selective transport requires cohesive FG domain interactions. To understand the functional roles of cohesive interactions, we studied monolayers of end-grafted FG domains as a bottom-up nanoscale model system of the permeability barrier. Based on detailed physicochemical analysis of the model films and comparison of the data with polymer theory, we propose that cohesiveness is tuned to promote rapid assembly of the permeability barrier and to generate a stable and compact pore-filling meshwork with a small mesh size. Our results highlight the functional importance of weak interactions, typically a few kBT per chain, and contribute important information to understand the mechanism of size-selective transport.
More Related Videos
Related Concept Videos
 01:34
Nuclear Protein Sorting
Proteins targeted to the nucleus carry nuclear localization signals or NLS recognized by import receptors in the cytosol. Similarly, proteins with nuclear export signals are recognized by export receptors. Import and export receptors are...
 00:59
Mechanisms of Membrane Domain Formation
Another mechanism for membrane domain formation involves membrane proteins interacting with...
 01:45
Regulation of Nuclear Protein Sorting
 01:32
Pinching-off of Coated Vesicles
 01:21
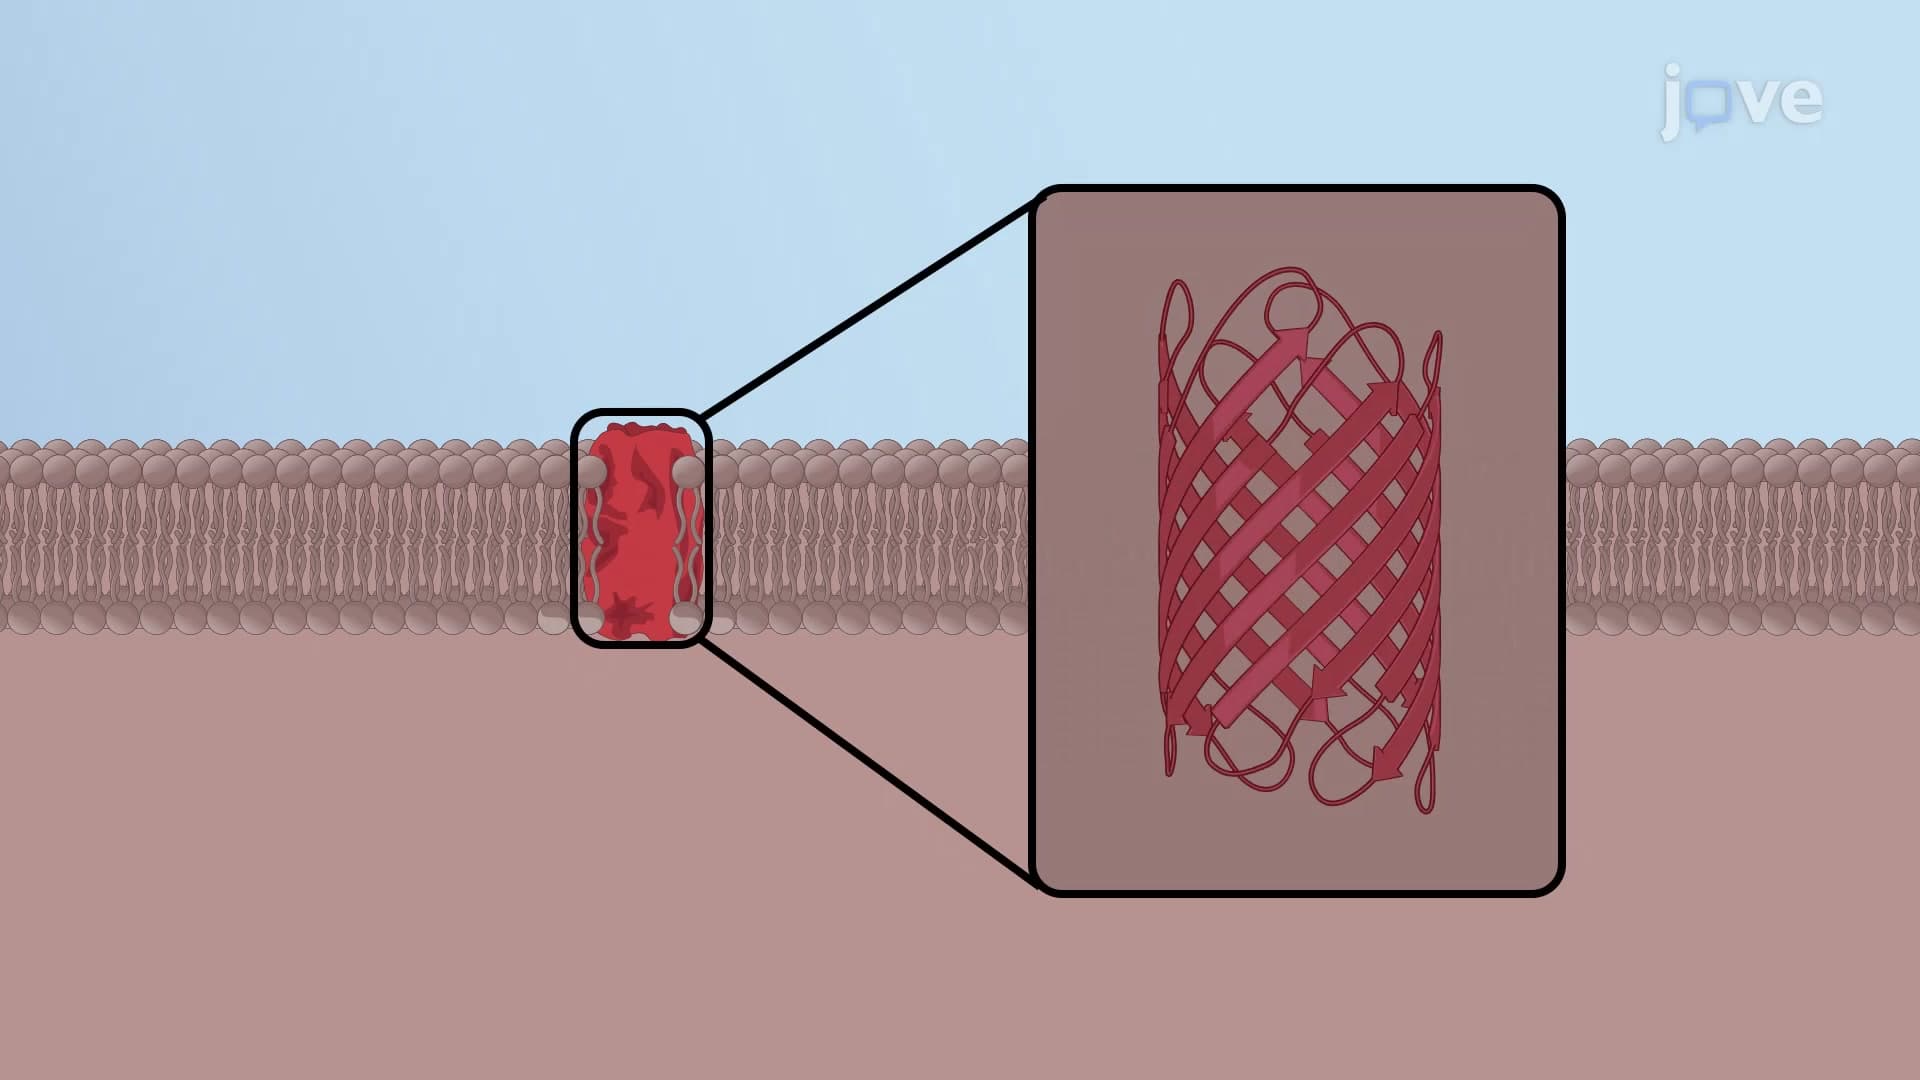
Structure of Porins
 01:46
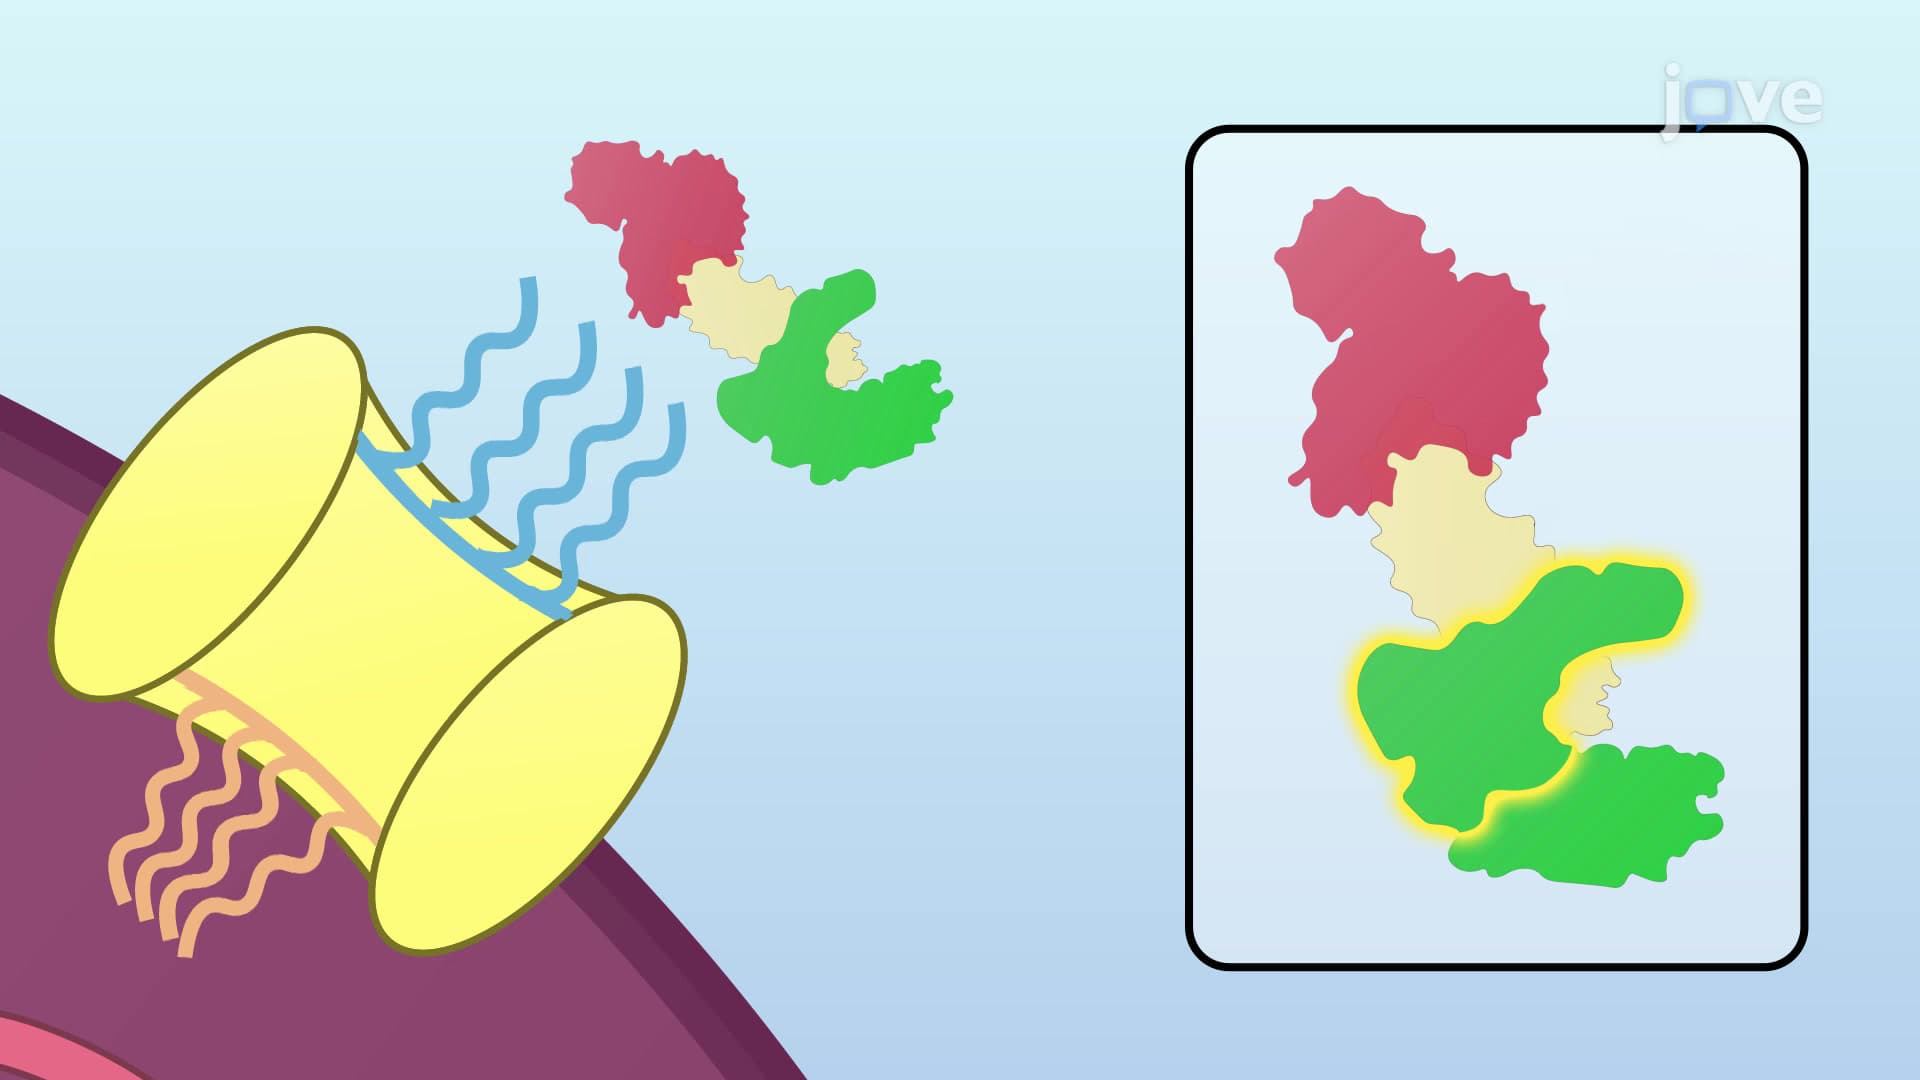
Nuclear Localization Signals and Import