Related Experiment Video
Updated: May 6, 2026
Fluorescent Leakage Assay to Investigate Membrane Destabilization by Cell-Penetrating Peptide
Published on: December 19, 2020
Mechanism of membrane permeation induced by synthetic β-hairpin peptides
Kshitij Gupta1, Hyunbum Jang, Kevin Harlen
1Basic Research Laboratory, Center for Cancer Research, National Cancer Institute, National Institutes of Health, Frederick, Maryland.

Abstract:
We have investigated the membrane destabilizing properties of synthetic amphiphilic cationic peptides, MAX1 and MAX35, which have the propensity to form β-hairpin structures under certain conditions, and a control non-β-hairpin-forming peptide MAX8V16E. All three peptides bind to liposomes containing a mixture of zwitterionic POPC and negatively charged POPS lipids as determined by Zeta potential measurements. Circular dichroism measurements indicated folding of MAX1 and MAX35 in the presence of the POPC/POPS liposomes, whereas no such folding was observed with MAX8V16E. There was no binding or folding of these peptides to liposomes containing only POPC. MAX1 and MAX35 induced release of contents from negatively charged liposomes, whereas MAX8V16E failed to promote solute release under identical conditions. Thus, MAX1 and MAX35 bind to, and fold at the surface of negatively charged liposomes adopting a lytic conformation. We ruled out leaky fusion as a mechanism of release by including 2 mol % PEG-PE in the liposomes, which inhibits aggregation/fusion but not folding of MAX or MAX-induced leakage. Using a concentration-dependent quenching probe (calcein), we determined that MAX-induced leakage of liposome contents was an all-or-none process. At MAX1 concentrations, which cause release of ~50% of the liposomes that contain small (R(h) <1.5 nm) markers, only ~15% of those liposomes release a fluorescent dextran of 40 kDa. A multimeric model of the pore is presented based on these results. Atomistic molecular dynamics simulations show that barrels consisting of 10 β-hairpin MAX1 and MAX35 peptides are relatively more stable than MAX8V16E barrels in the bilayer, suggesting that barrels of this size are responsible for the peptides lytic action.
Insights
Synthetic peptides MAX1 and MAX35 destabilize negatively charged liposomes by forming β-hairpin structures and inducing content release. This membrane-lytic action, distinct from fusion, involves pore formation by peptide barrels.
Area of Science:
- Biophysics
- Materials Science
- Biochemistry
Background:
- Synthetic amphiphilic cationic peptides are explored for their membrane interaction properties.
- Peptide structure, particularly β-hairpin formation, can influence membrane activity.
- Understanding peptide-membrane interactions is crucial for developing novel therapeutic or delivery agents.
Purpose of the Study:
- To investigate the membrane destabilizing properties of synthetic peptides MAX1 and MAX35, which can form β-hairpin structures.
- To compare the activity of β-hairpin-forming peptides with a control peptide (MAX8V16E) that does not form β-hairpins.
- To elucidate the mechanism of peptide-induced liposome content release.
Main Methods:
- Zeta potential measurements to assess peptide binding to liposomes.
- Circular dichroism spectroscopy to monitor peptide folding in the presence of liposomes.
- Solute release assays using quenching probes and fluorescent dextrans to quantify content leakage.
- Molecular dynamics simulations to model peptide barrel formation and stability.
Main Results:
- MAX1 and MAX35 bind to and fold at the surface of negatively charged liposomes (POPC/POPS), adopting a lytic conformation.
- MAX1 and MAX35 induce significant content release from negatively charged liposomes, unlike the control peptide MAX8V16E.
- Peptide-induced leakage is an all-or-none process and is not mediated by membrane fusion, as confirmed by PEG-PE experiments.
- Molecular dynamics simulations suggest stable barrels of 10 β-hairpin peptides (MAX1/MAX35) are responsible for lytic action.
Conclusions:
- The β-hairpin forming peptides MAX1 and MAX35 exhibit membrane lytic activity through binding and conformational changes at the liposome surface.
- The mechanism of action involves the formation of peptide barrels, creating pores that lead to content release.
- These findings provide insights into structure-activity relationships for membrane-lytic peptides and potential pore-forming mechanisms.
Related Concept Videos
 01:09
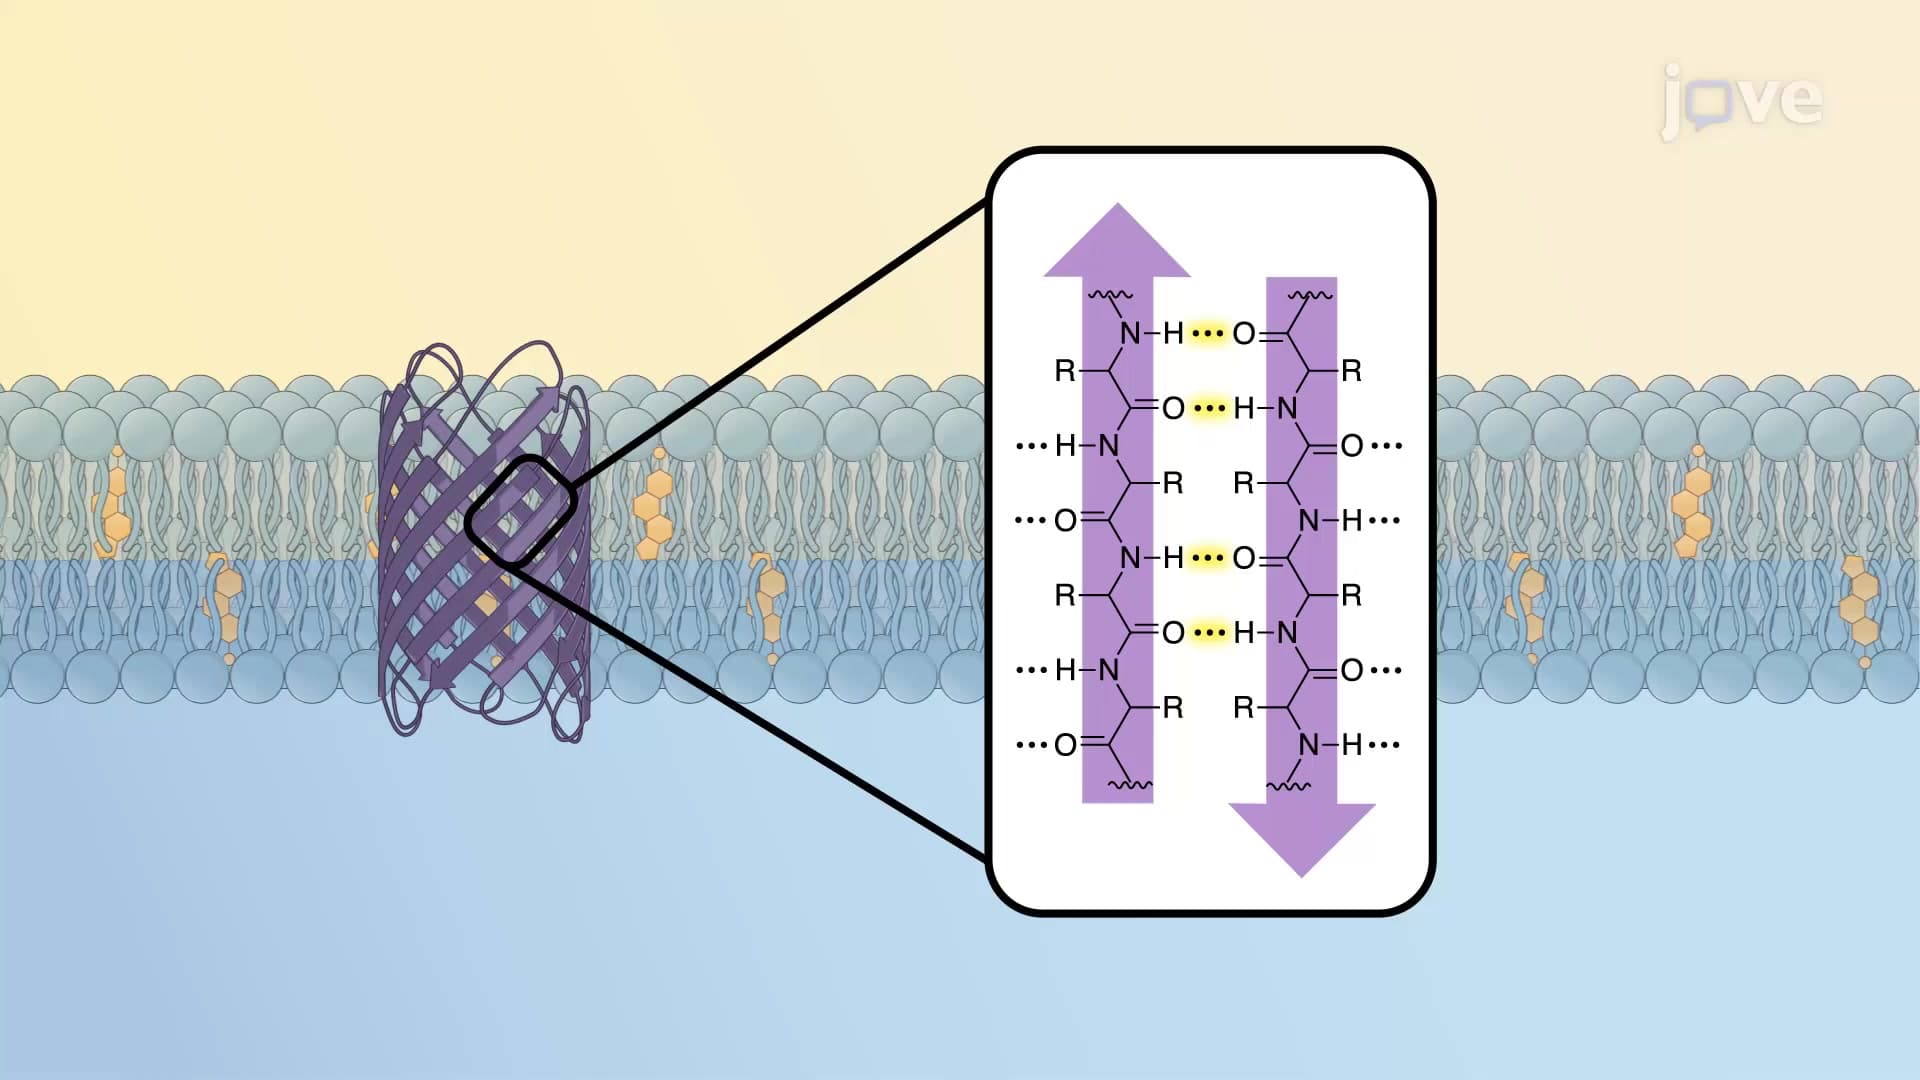
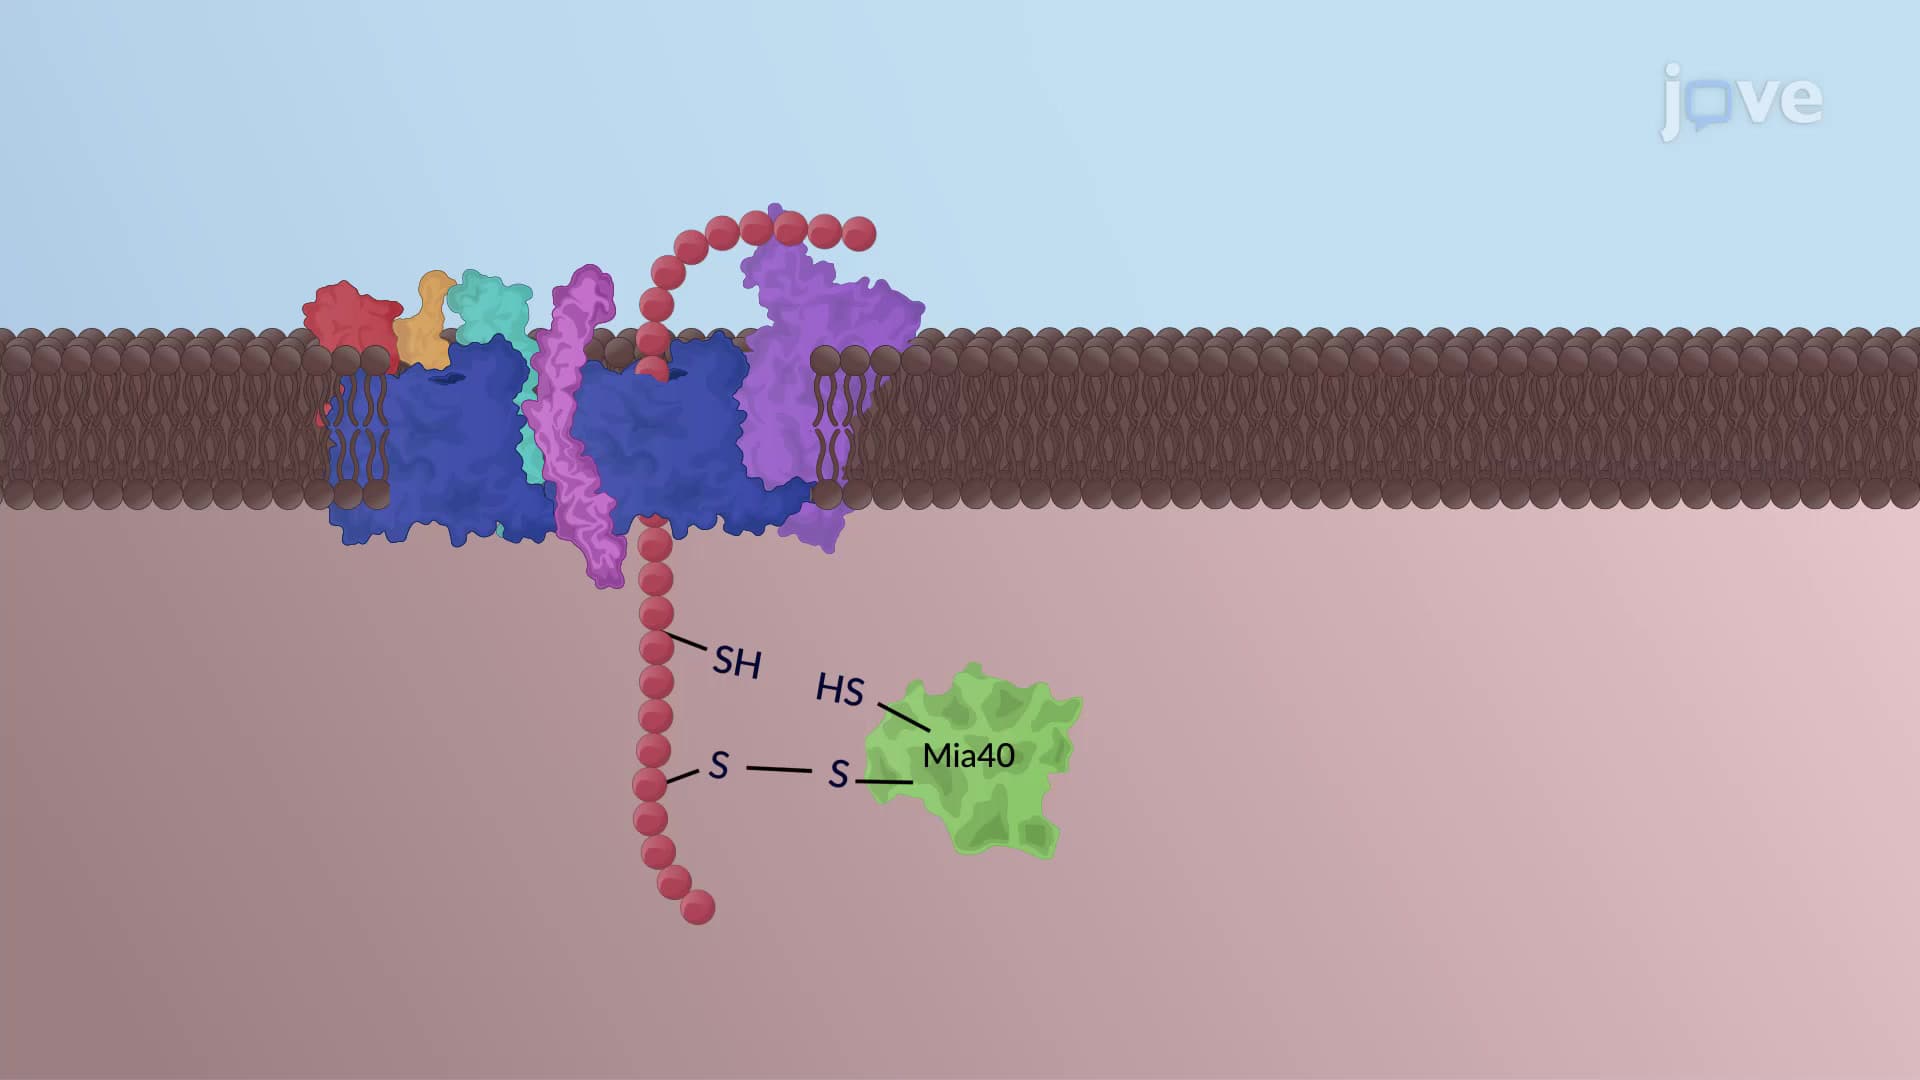
Multi-pass Transmembrane Proteins and β-barrels
α-Helix containing multi-pass transmembrane proteins
Multi-pass transmembrane proteins such as...
 01:19
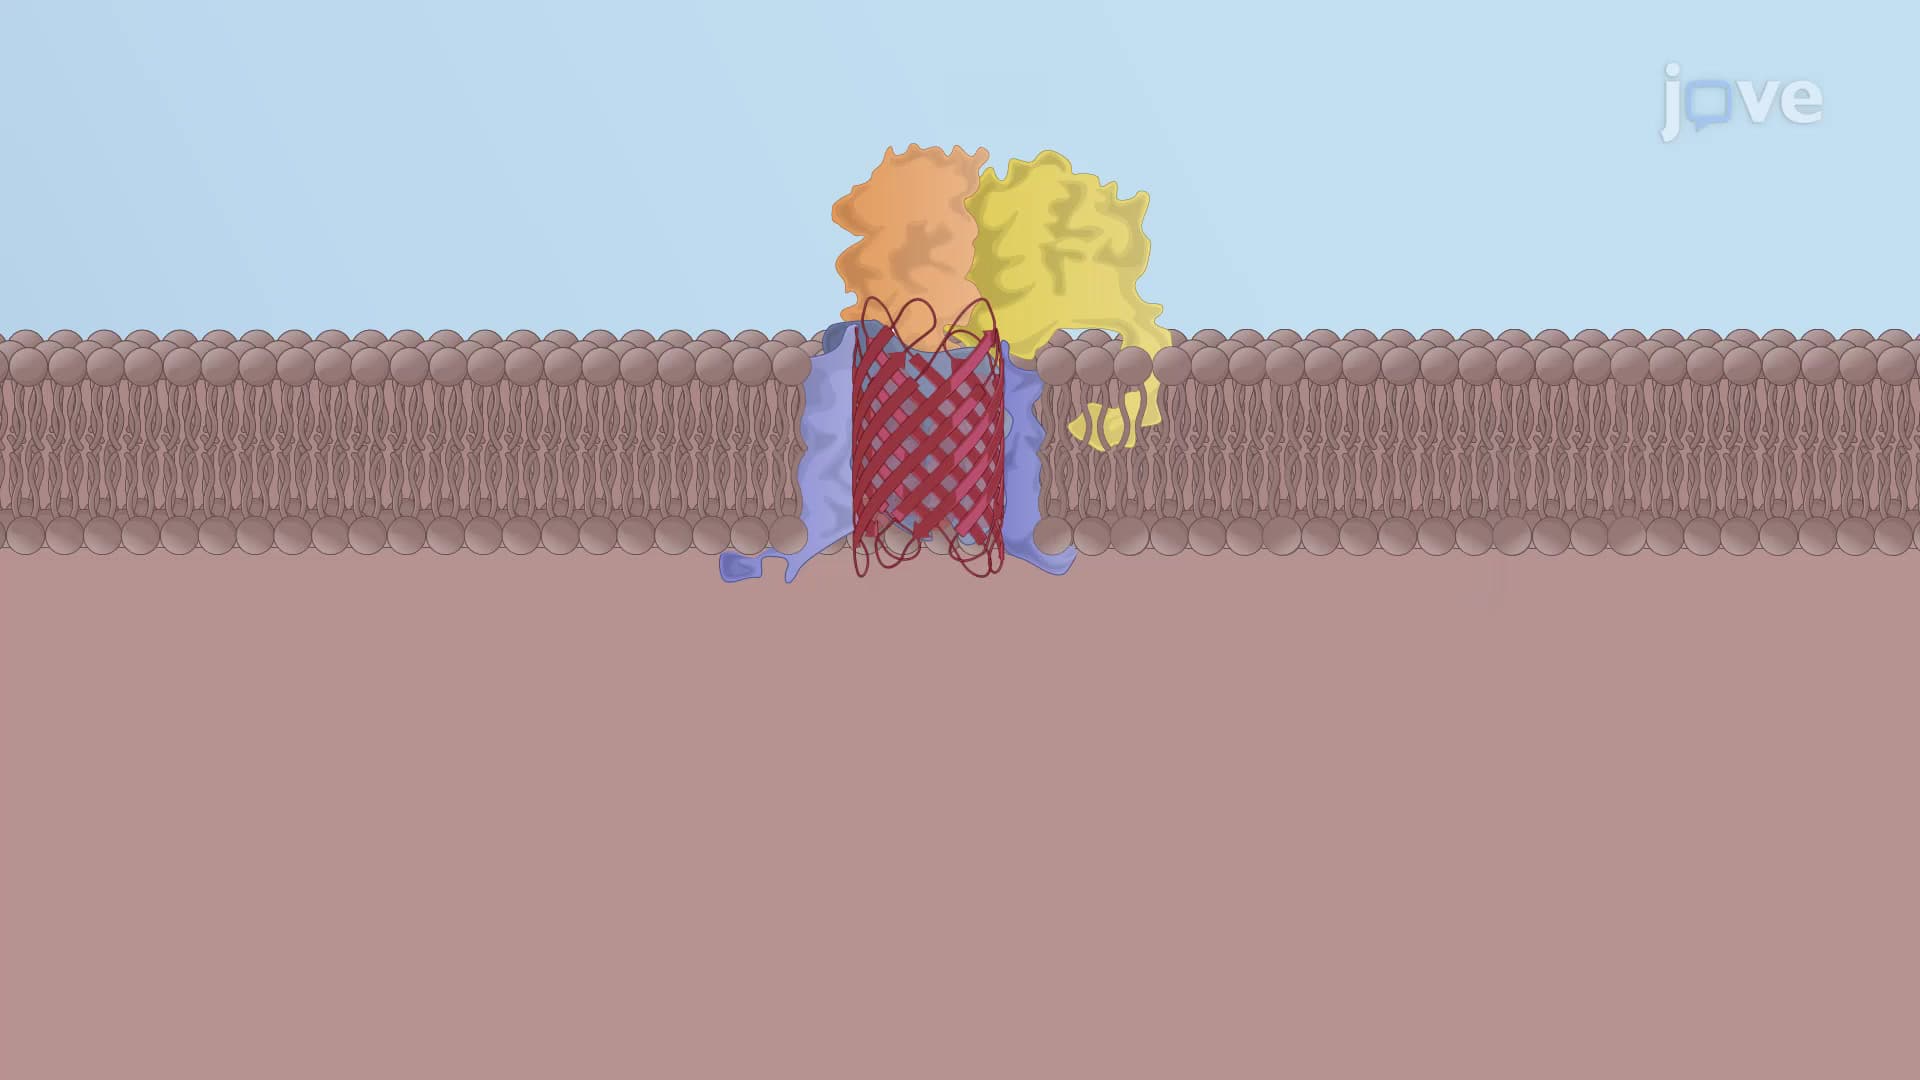
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:12
Porin Insertion in the Outer Mitochondrial Membrane
Three models describe the assembly of porins by the SAM complex and their insertion into the outer membrane. Model 1 suggests that porins are assembled outside the SAM channel as the...
 01:15
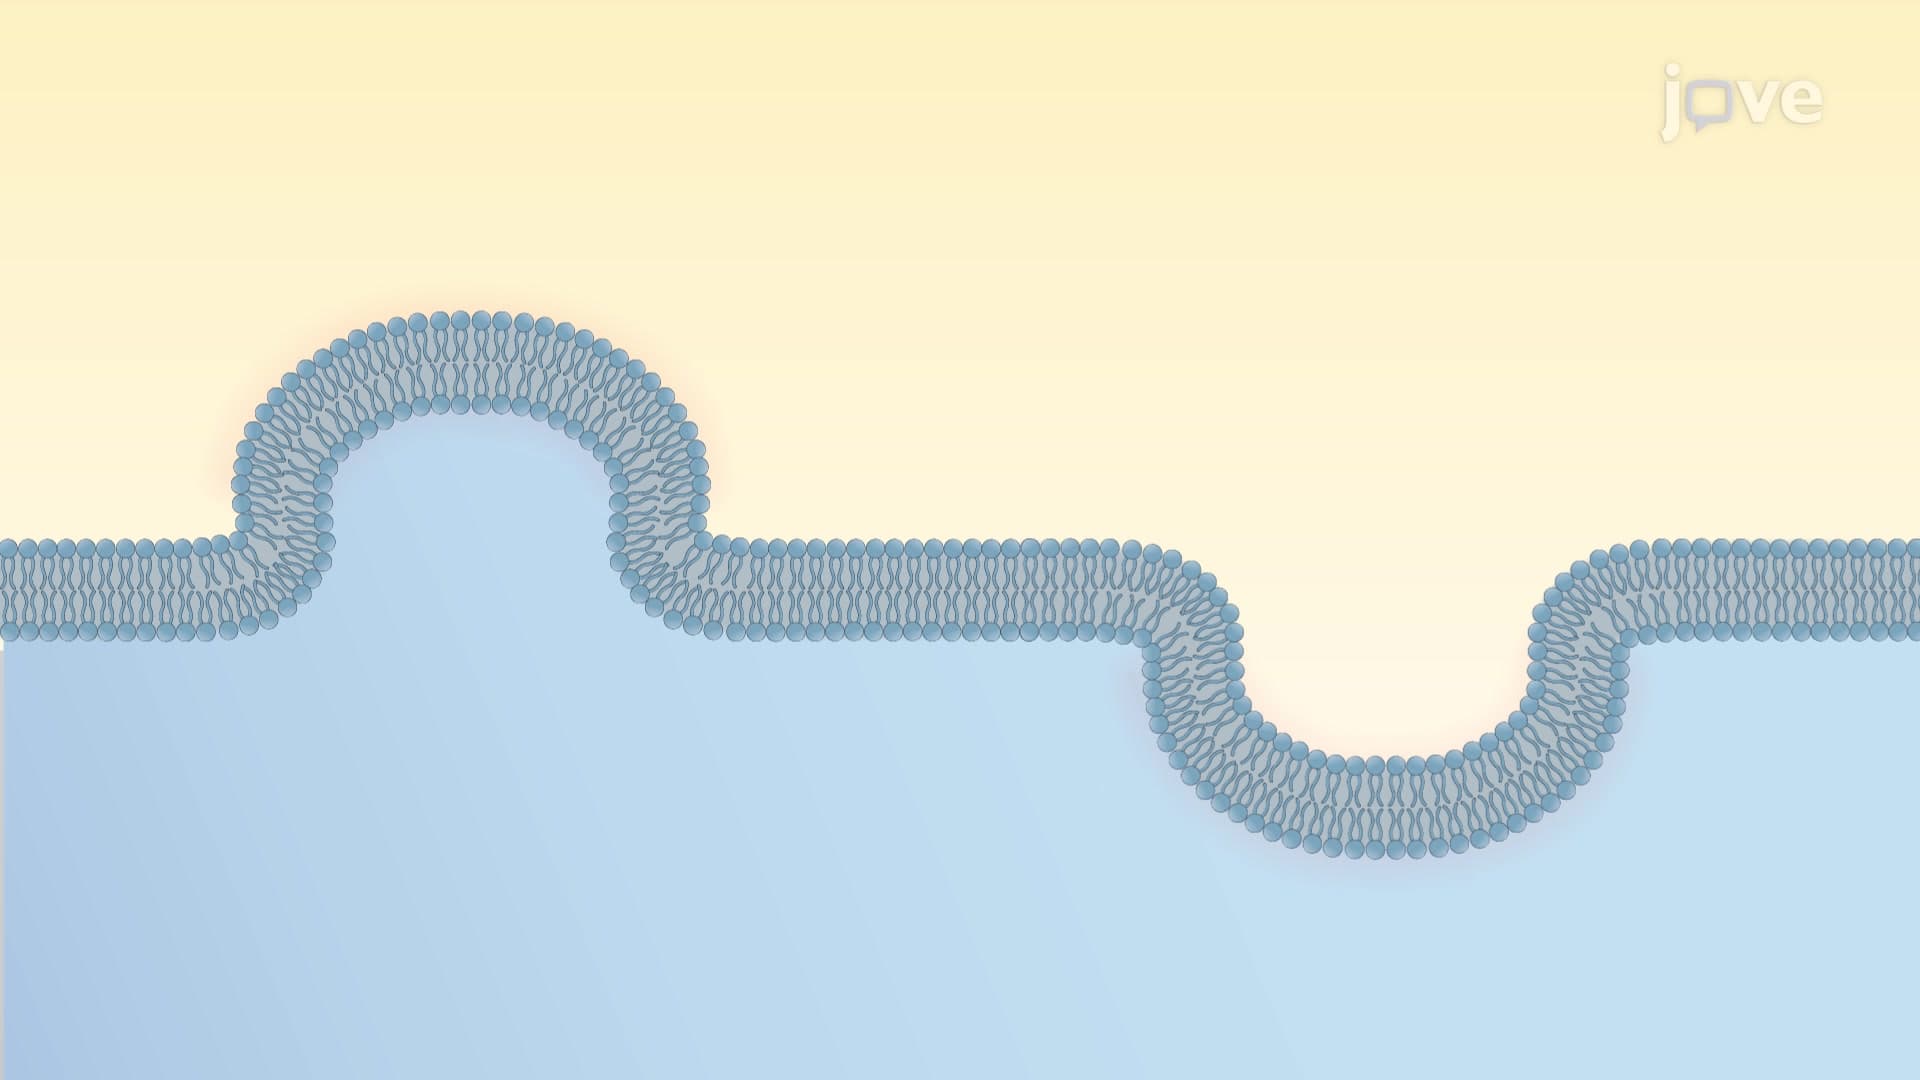
Mechanisms of Membrane-bending
Membrane bending can happen due to intrinsic changes in lipid composition or extrinsic association with different proteins. The proteins involved...
 01:26
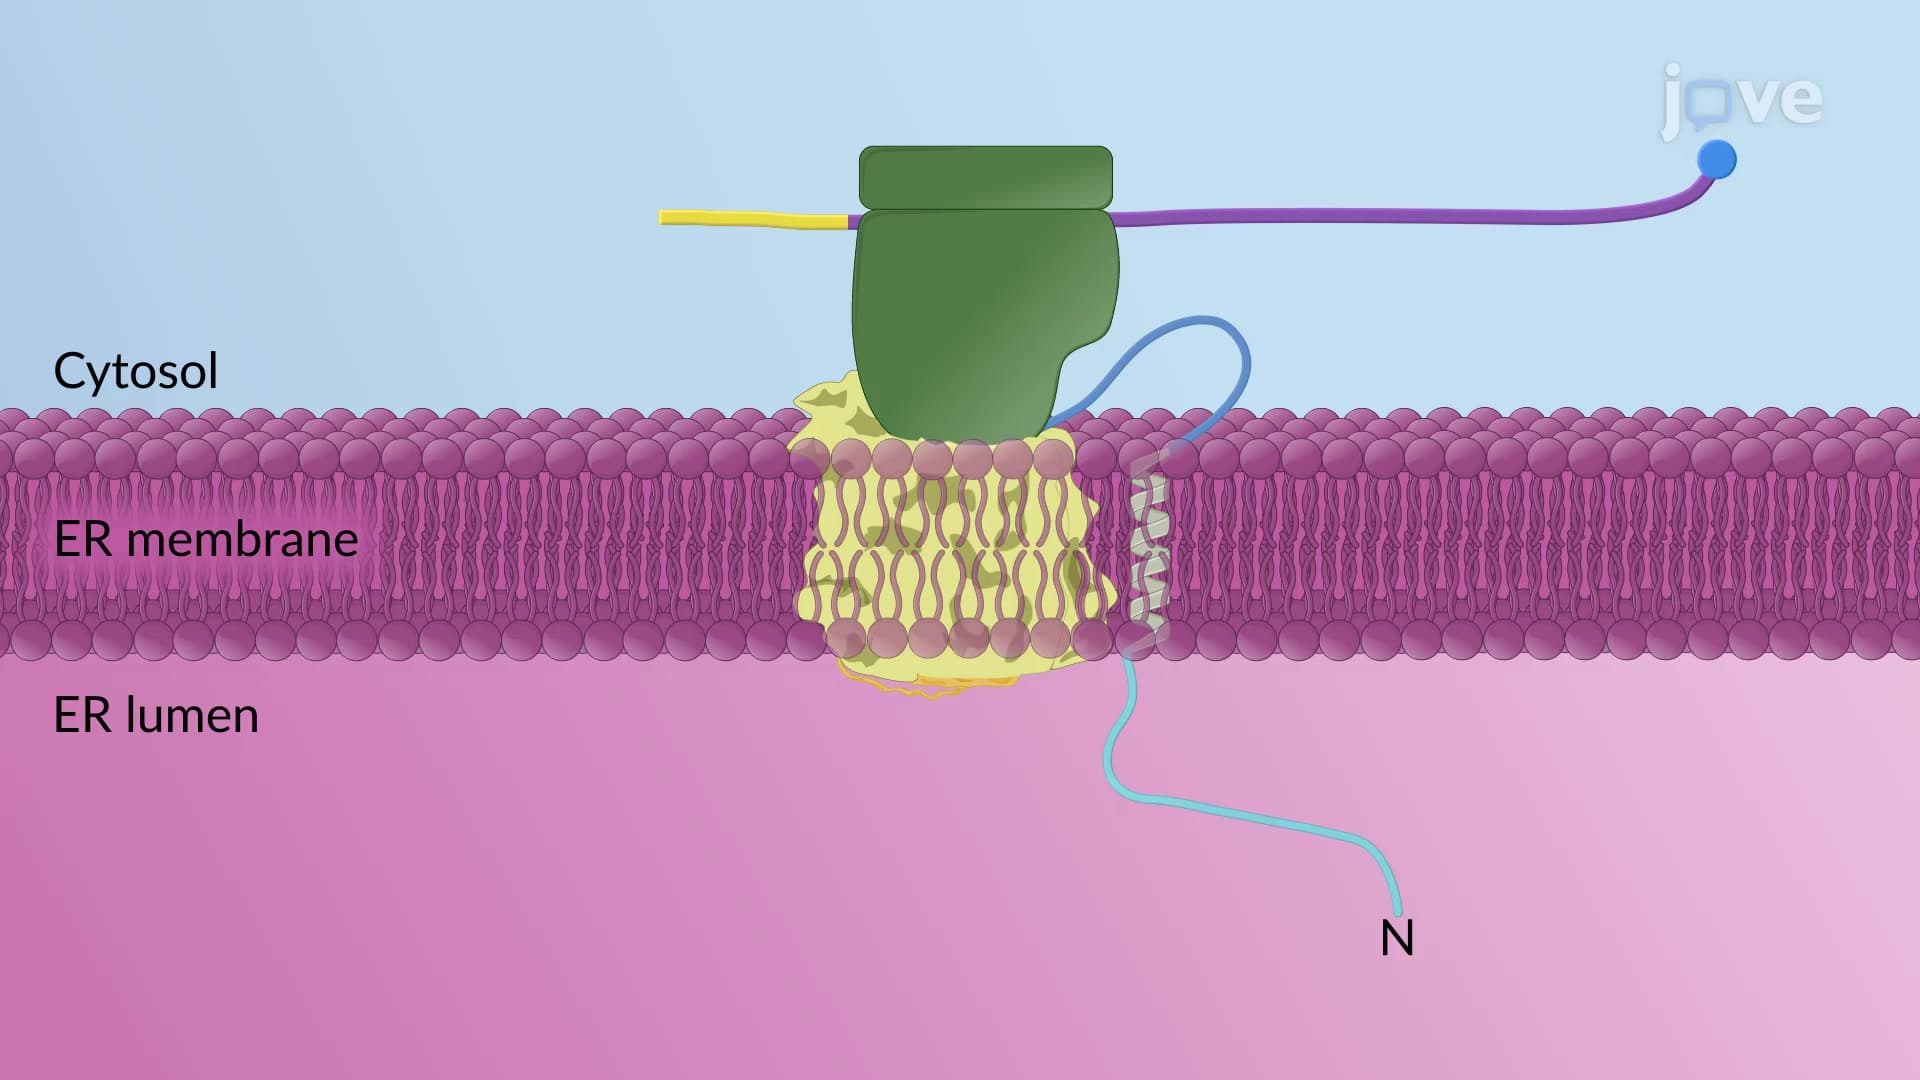
Insertion of Single-pass Transmembrane Proteins in the RER
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
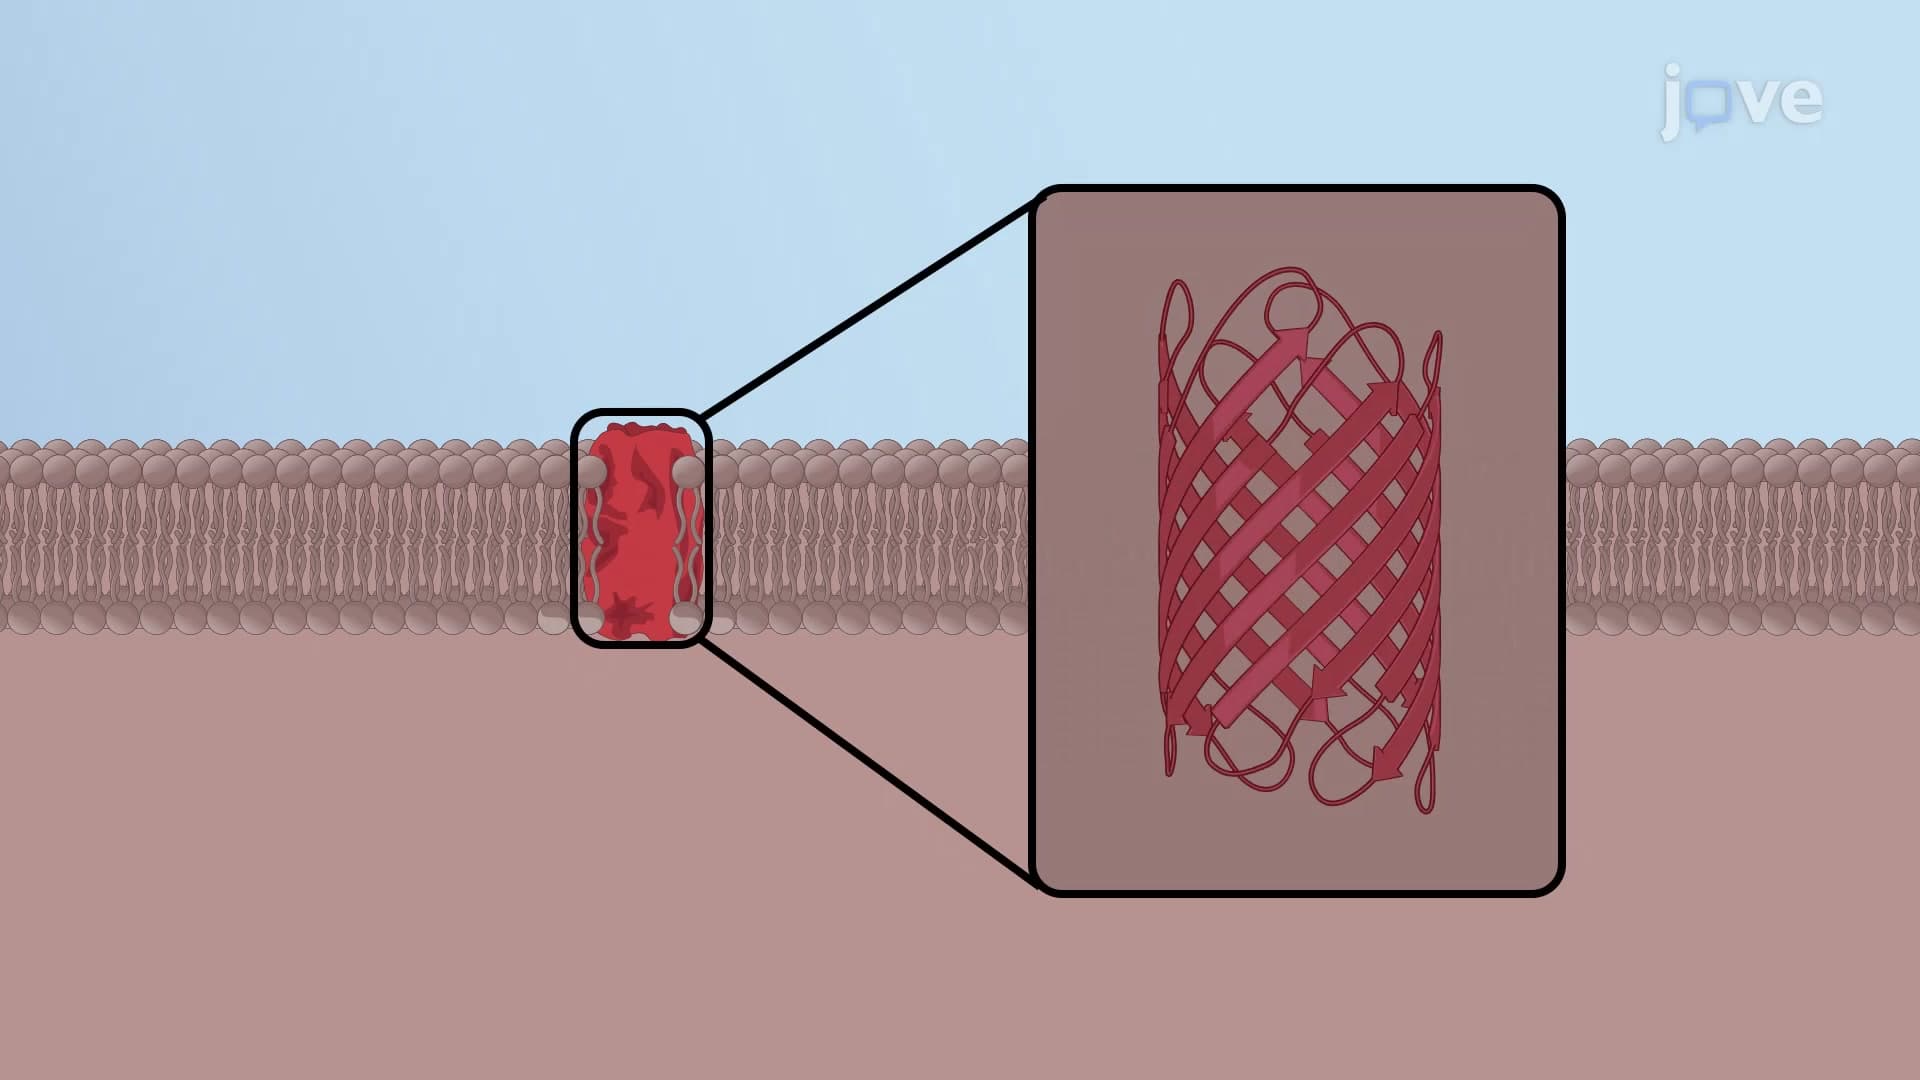 01:21
Structure of Porins