Related Experiment Video
Updated: May 5, 2026

Nanopodia - Thin, Fragile Membrane Projections with Roles in Cell Movement and Intercellular Interactions
Published on: April 3, 2014
The cytosolic N-terminus of CD317/tetherin is a membrane microdomain exclusion motif
Peter G Billcliff1, Oforiwa A Gorleku, Luke H Chamberlain
1School of Biochemistry, University of Bristol , Bristol BS8 1TD , UK ; Present address: Faculty of Life Sciences, University of Manchester, Manchester M13 9PL, UK.

Abstract:
The integral membrane protein CD317/tetherin has been associated with a plethora of biological processes, including restriction of enveloped virus release, regulation of B cell growth, and organisation of membrane microdomains. CD317 possesses both a conventional transmembrane (TM) domain and a glycophosphatidylinositol (GPI) anchor. We confirm that the GPI anchor is essential for CD317 to associate with membrane microdomains, and that the TM domain of CD44 is unable to rescue proper microdomain association of a ΔGPI-CD317 construct. Additionally, we demonstrate that the cytosolic amino terminal region of CD317 can function as a 'microdomain-excluding' motif, when heterologously expressed as part of a reporter construct. Finally, we show that two recently described isoforms of CD317 do not differ in their affinity for membrane microdomains. Together, these data help further our understanding of the fundamental cell biology governing membrane microdomain association of CD317.
Related Concept Videos
 01:45
Tail-anchoring of Proteins in the ER Membrane
 01:26
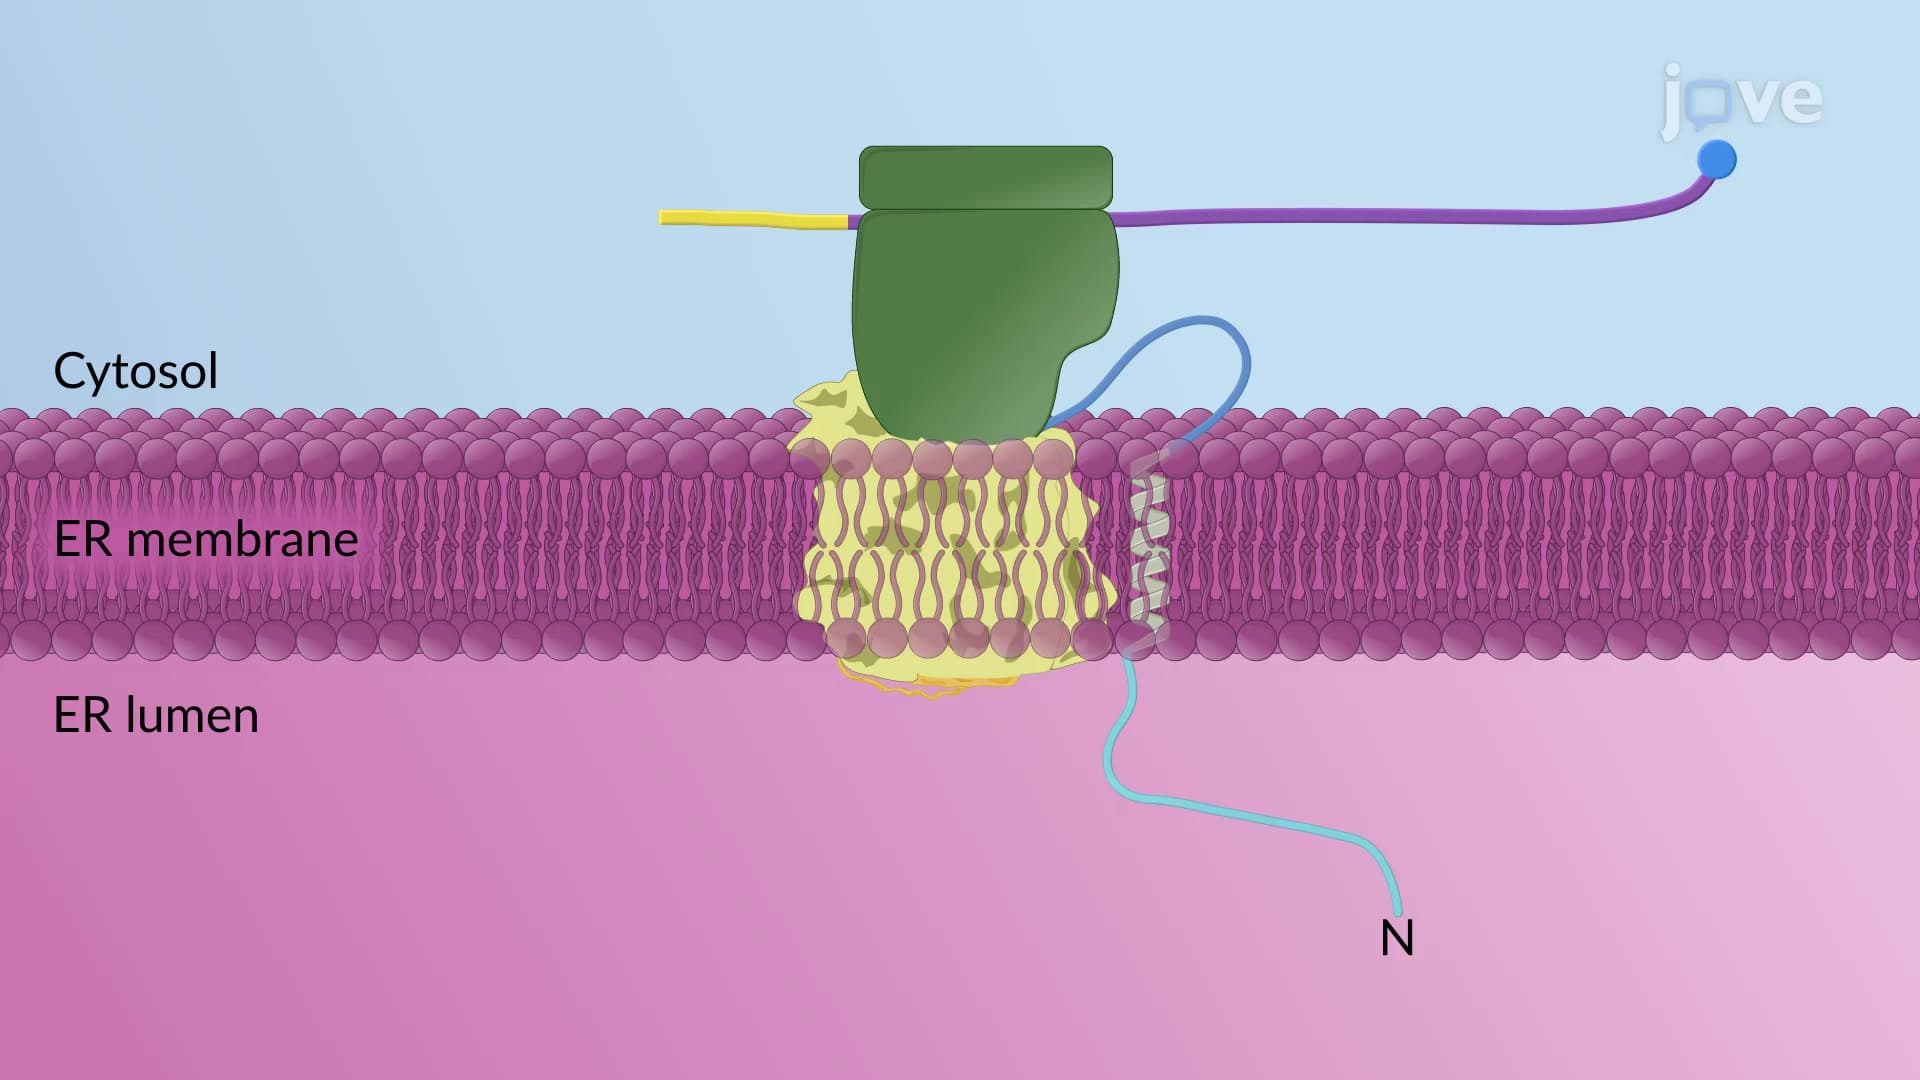
Insertion of Single-pass Transmembrane Proteins in the RER
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
 01:29
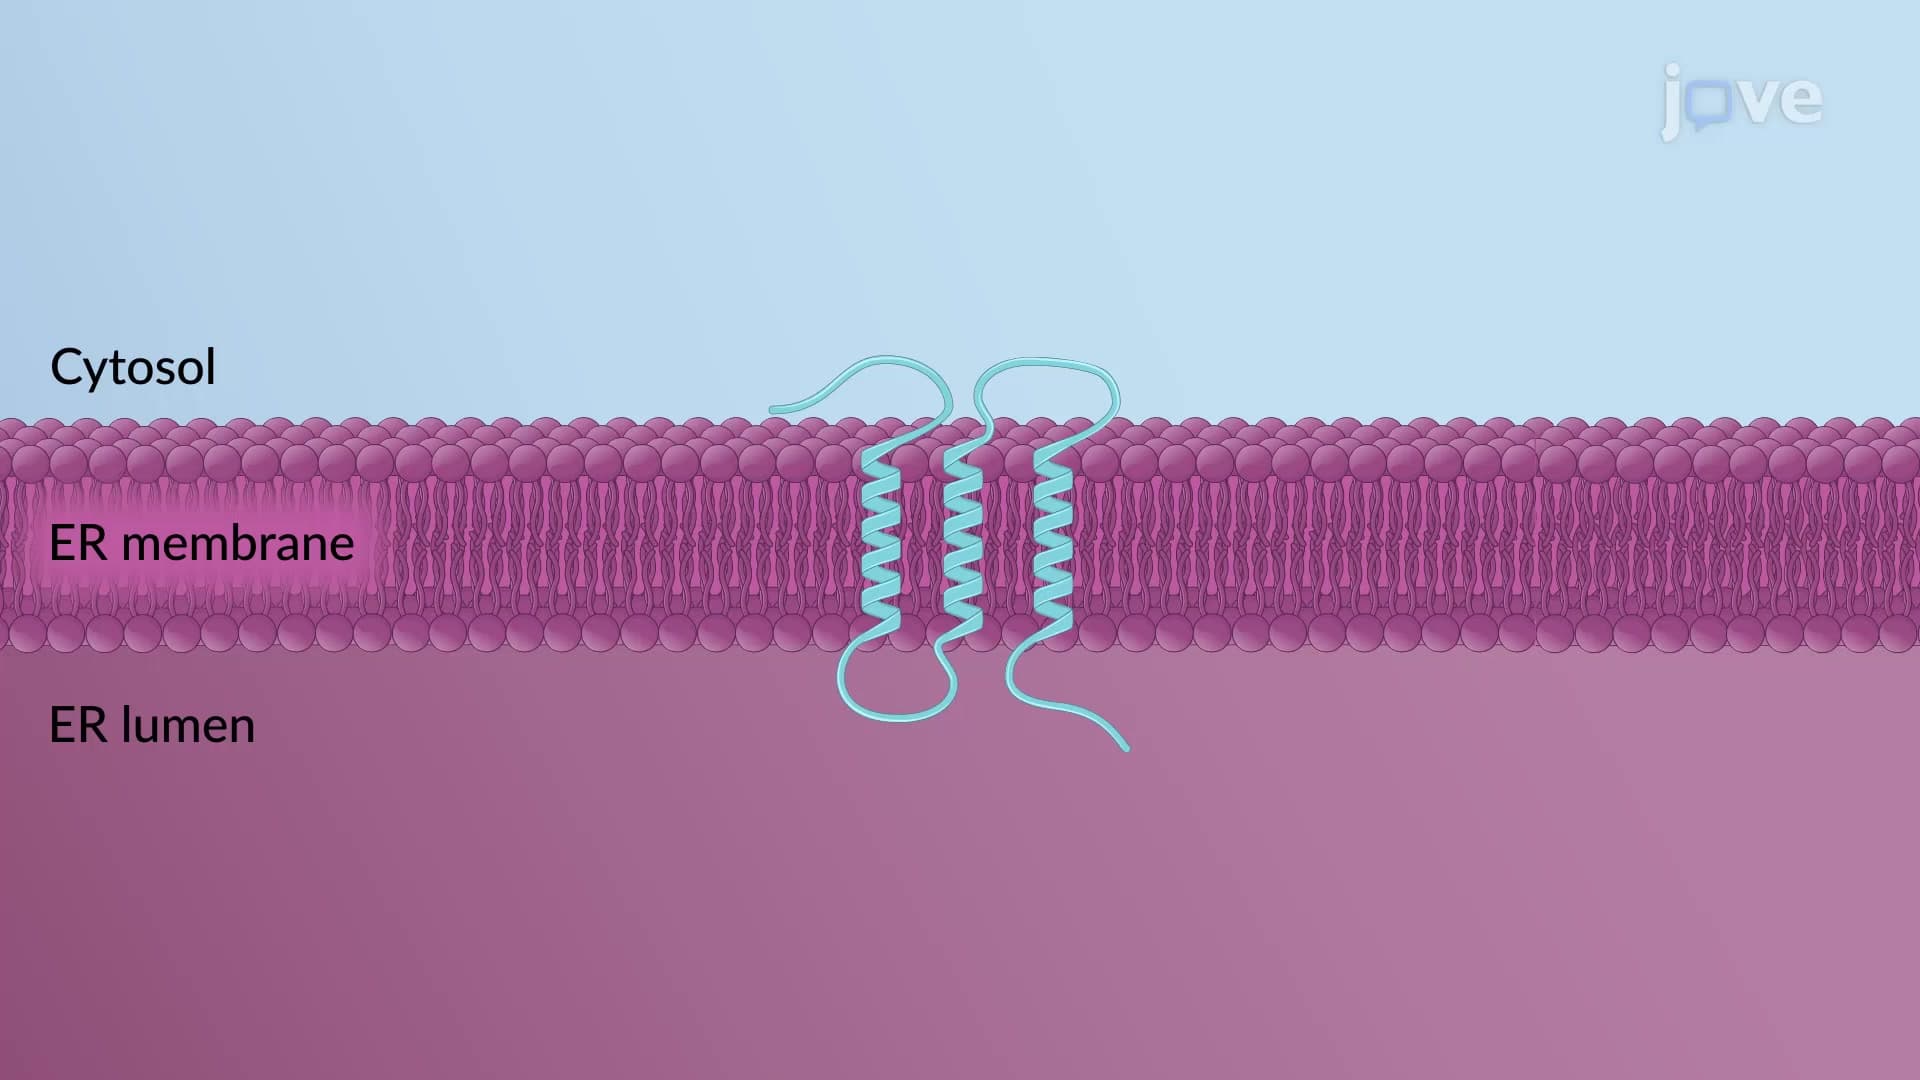
Insertion of Multi-pass Transmembrane Proteins in the RER
The multipass transmembrane proteins are the type IV integral membrane proteins with multiple topogenic sequences determining their spatial arrangement in the ER membrane. Nearly all multipass proteins lack a cleavable signal sequence and use...
 01:19
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:34
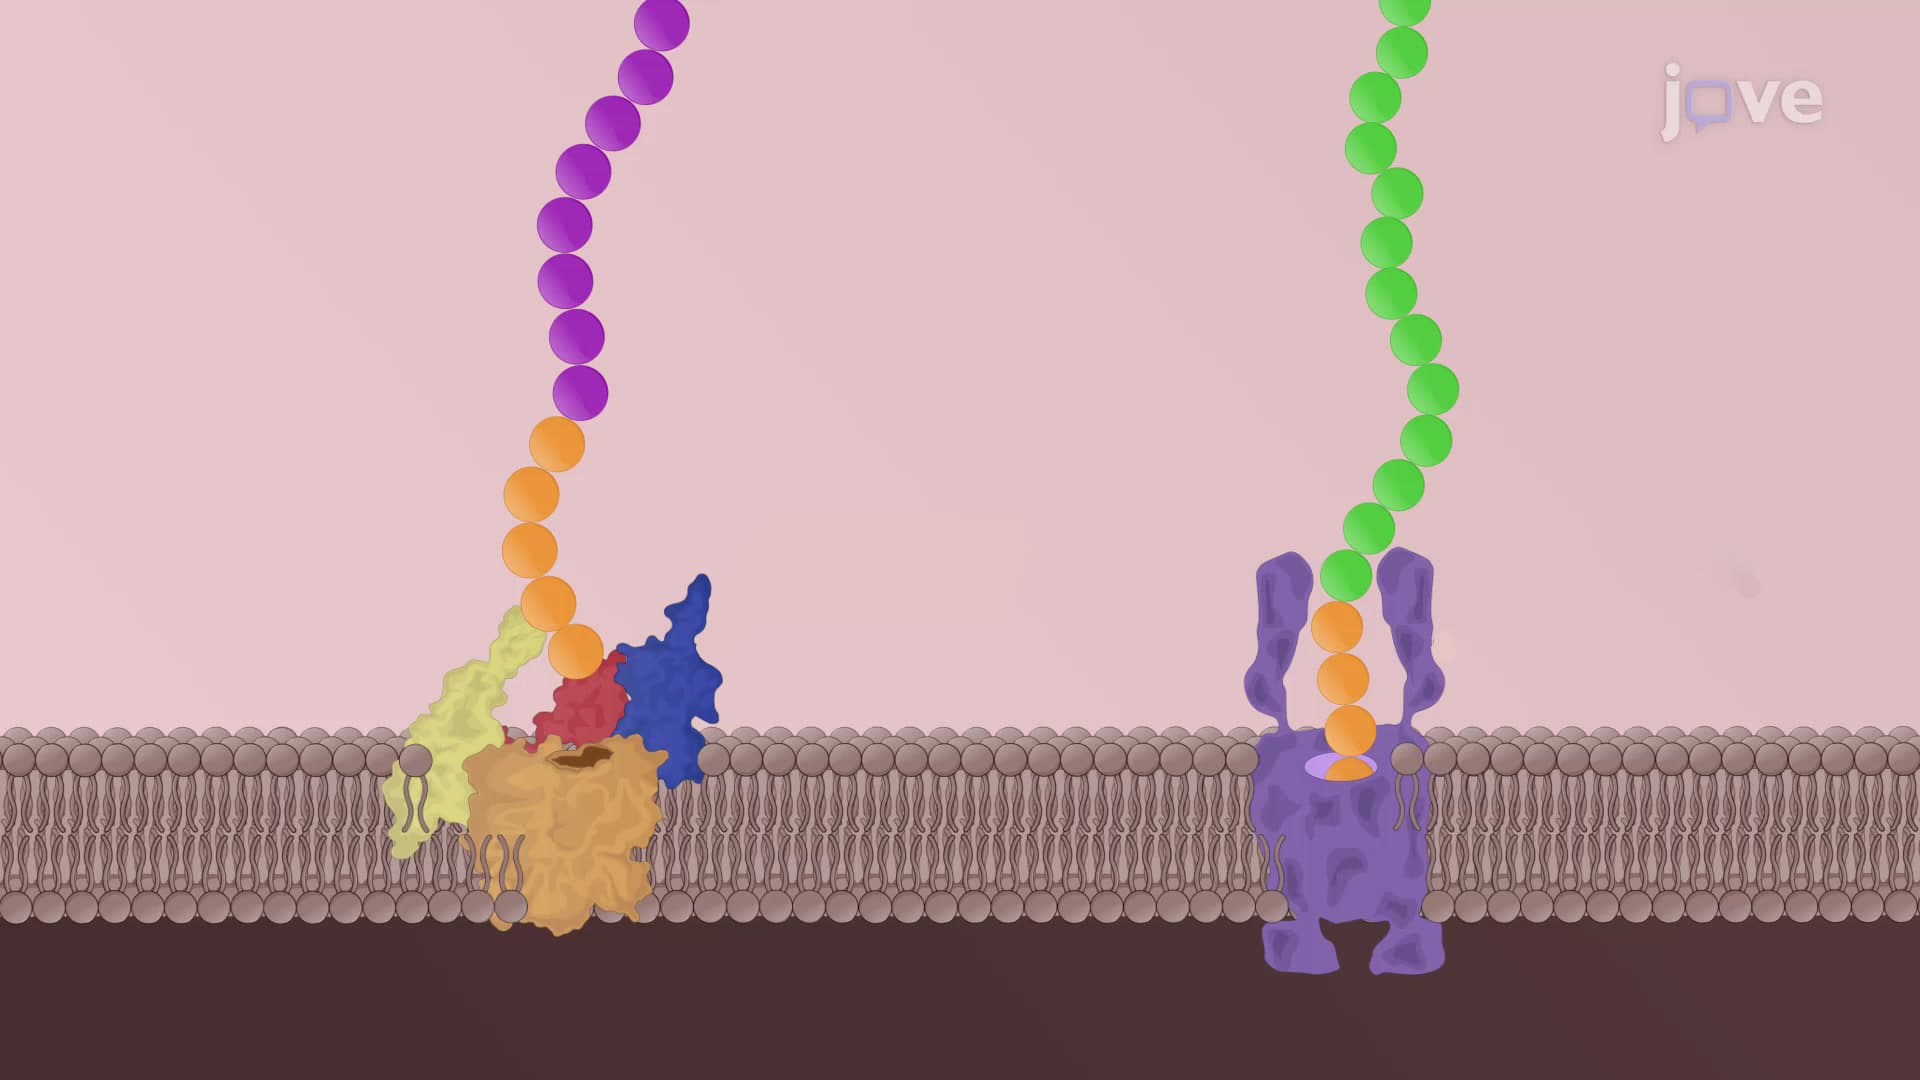
Protein Transport into the Inner Mitochondrial Membrane
Transport of mitochondrial precursors across the TIM23 channel is driven by...
 01:23
Catenins
Catenins in Cell Junctions
Catenins bind to cell adhesion molecules such as cadherins and link them to different cytoskeletal proteins depending on the type of cell junction. At the...