Related Experiment Video
Updated: Aug 3, 2026
Vibrodissociation of Neurons from Rodent Brain Slices to Study Synaptic Transmission and Image Presynaptic Terminals
Published on: May 25, 2011
Action of benzocaine on sodium channels of frog nodes of Ranvier treated with chloramine-T

Abstract:
Single myelinated nerve fibres of the frog Rana esculenta were voltage clamped in solutions containing 10 mM TEA to block potassium channels. Reduction of peak INa was measured after equilibrating the membrane in solution containing benzocaine between 0.025 and 2.0 mM. A Hill plot of this effect revealed a slope nH approximately 1 between 0.25 and 1.0 mM but showed deviations for the lowest concentrations (nH less than 1) and the highest concentration (nH greater than 1). Treatment with 0.6 mM chloramine-T irreversibly partially inhibited inactivation of sodium channels leading to a large INa component persisting during depolarization. After treatment the benzocaine effect on peak INa (tested with 0.25-1.0 mM) was unchanged but the persistent component was much more depressed. Benzocaine shifted the steady-state inactivation curve to more negative potentials. This was also observed after chloramine-T treatment which itself produced a curve of decreased slope, shifted to more positive potentials. Recovery from inactivation was studied at different levels of hyperpolarization; it was diphasic in anaesthetic-free solutions before and after chloramine-T treatment although slowed in the latter case. In benzocaine recovery started with a delay (less than 0.6 ms at 16-18 degrees C) and proceeded with a single time constant that decreased with increasing hyperpolarization, was independent of benzocaine concentration and not affected by chloramine-T. The results are compatible with the idea that the affinity of the binding site for benzocaine increases when the channel state changes from resting to open to inactivated with equilibrium dissociation constants of the reaction with resting channels, KR = 0.7 mM and with inactivated channels, KI = 0.04 mM.(ABSTRACT TRUNCATED AT 250 WORDS)
More Related Videos
 17:05
Loading a Calcium Dye into Frog Nerve Endings Through the Nerve Stump: Calcium Transient Registration in the Frog Neuromuscular Junction
Published on: July 8, 2017
 07:19
Recording of Inward Rectifying K+ Currents in Freshly Isolated Basilar Artery Smooth Muscle Cells by Patch Clamp Technique
Published on: February 7, 2025
Related Concept Videos
 01:24
Resting Membrane Potential
The Inside of a Neuron is More Negative
The membrane potential of a cell can be measured by inserting a microelectrode into a cell and comparing the charge to a reference electrode in the extracellular fluid. The...
 01:26
Voltage-gated Ion Channels
Generally, all voltage-gated ion channels have a 'voltage-sensing domain' that spans the lipid bilayer. The charged residues in the sensor move in response to the membrane potential changes that open the channel allowing ions movement. There are several types of...
 01:17
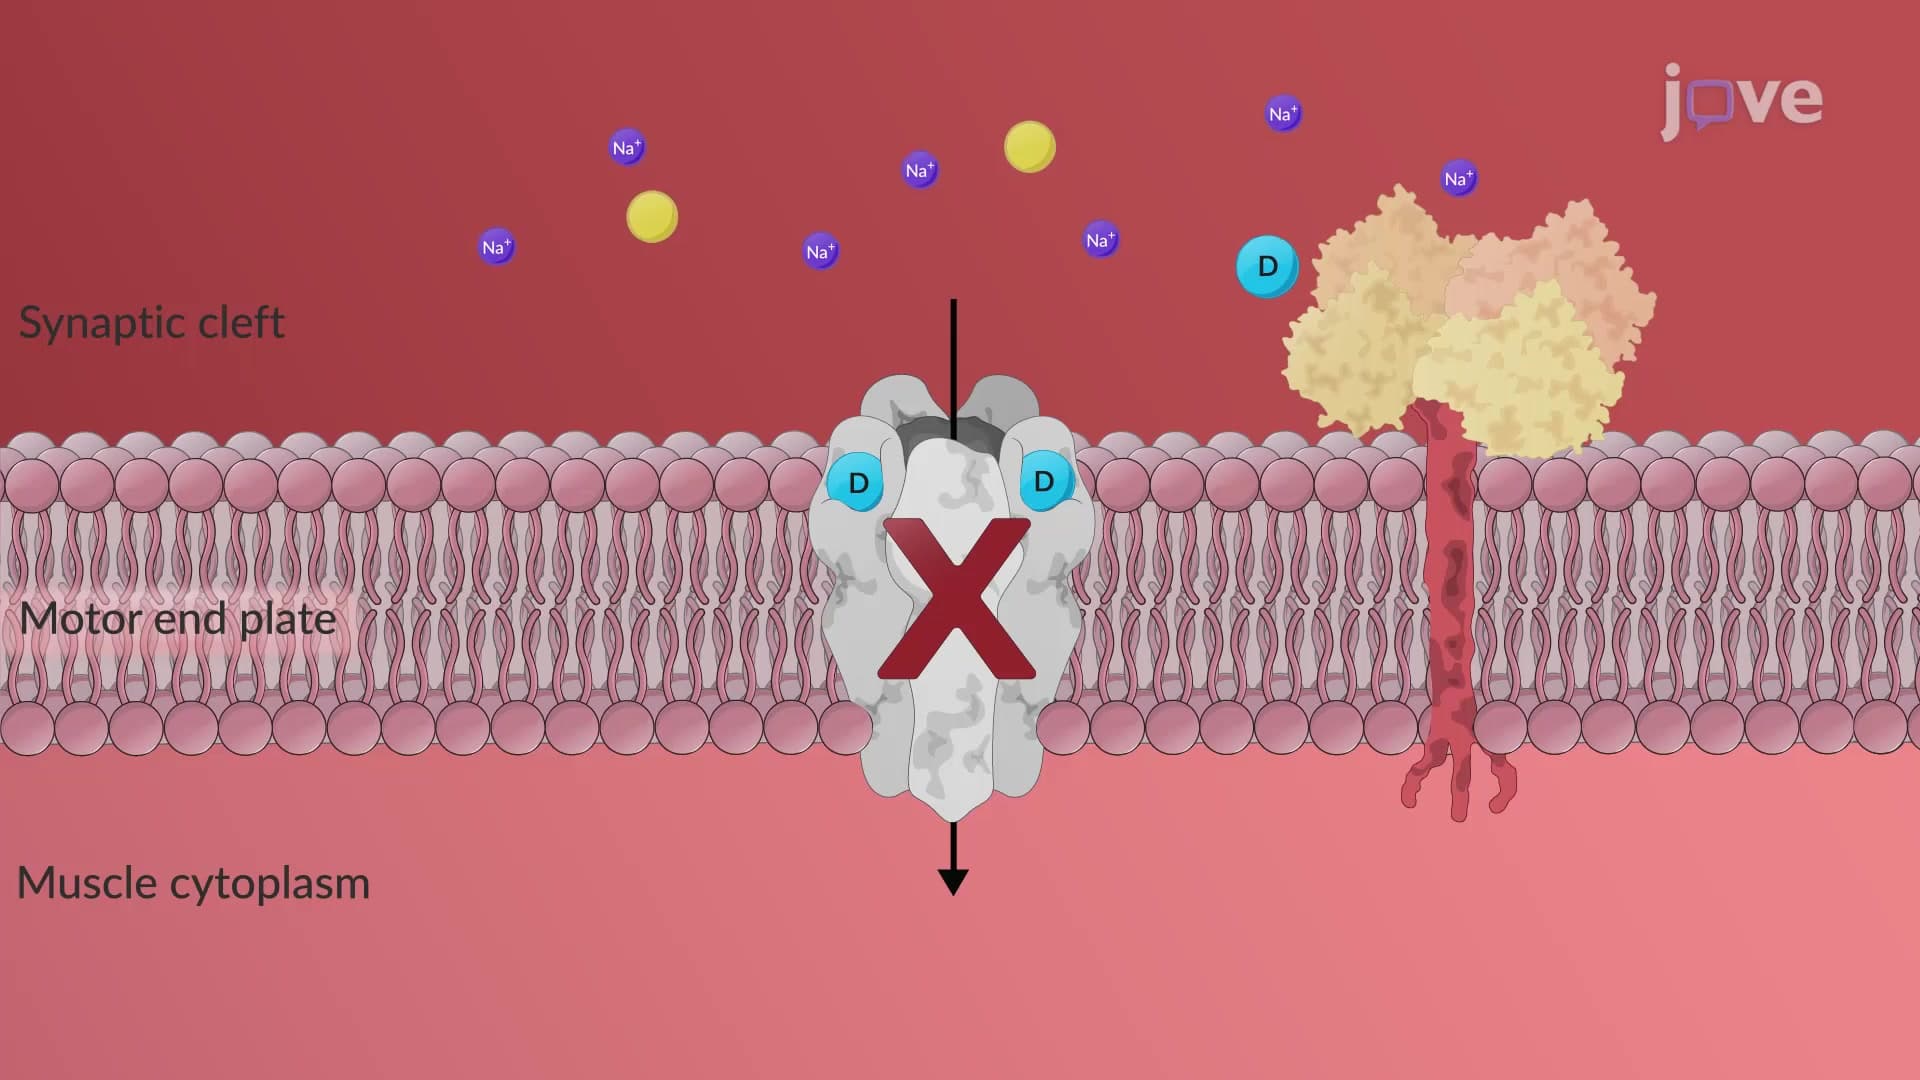
Nondepolarizing (Competitive) Neuromuscular Blockers: Mechanism of Action
Competitive antagonists prevent acetylcholine from binding to its receptor, inhibiting membrane depolarization. Without conformational changes or intrinsic...
 01:28
Depolarizing Blockers: Mechanism of Action
Succinylcholine is the most commonly used depolarizing blocker. Chemically, it constitutes two molecules of acetylcholine joined together by an acetate methyl group. They act on the receptors in the same way as acetylcholine. Because succinylcholine...
 01:23
Local Anesthetics: Mechanism of Action
Local anesthetics are amphiphilic molecules consisting of a hydrophobic aromatic part linked to a hydrophilic group by an ester or amide linkage. They are weak bases and are usually available as salts, which increases their solubility and stability. Once administered, LAs exist in the body either...
 01:22
Antiarrhythmic Drugs: Class I Agents as Sodium Channel Blockers
Class 1A Antiarrhythmic Drugs: These drugs work by moderately blocking sodium channels,...