Related Experiment Video
Updated: May 3, 2026
Application of Genetically Encoded Fluorescent Nitric Oxide (NO•) Probes, the geNOps, for Real-time Imaging of NO• Signals in Single Cells
Published on: March 16, 2017
Nitrite reductase and nitric-oxide synthase activity of the mitochondrial molybdopterin enzymes mARC1 and mARC2
Courtney E Sparacino-Watkins1, Jesús Tejero2, Bin Sun1
1Vascular Medicine Institute, University of Pittsburgh, Pittsburgh, Pennsylvania 15261; Division of Pulmonary, Allergy, and Critical Care Medicine, University of Pittsburgh, Pittsburgh, Pennsylvania 15213.

Abstract:
Mitochondrial amidoxime reducing component (mARC) proteins are molybdopterin-containing enzymes of unclear physiological function. Both human isoforms mARC-1 and mARC-2 are able to catalyze the reduction of nitrite when they are in the reduced form. Moreover, our results indicate that mARC can generate nitric oxide (NO) from nitrite when forming an electron transfer chain with NADH, cytochrome b5, and NADH-dependent cytochrome b5 reductase. The rate of NO formation increases almost 3-fold when pH was lowered from 7.5 to 6.5. To determine if nitrite reduction is catalyzed by molybdenum in the active site of mARC-1, we mutated the putative active site cysteine residue (Cys-273), known to coordinate molybdenum binding. NO formation was abolished by the C273A mutation in mARC-1. Supplementation of transformed Escherichia coli with tungsten facilitated the replacement of molybdenum in recombinant mARC-1 and abolished NO formation. Therefore, we conclude that human mARC-1 and mARC-2 are capable of catalyzing reduction of nitrite to NO through reaction with its molybdenum cofactor. Finally, expression of mARC-1 in HEK cells using a lentivirus vector was used to confirm cellular nitrite reduction to NO. A comparison of NO formation profiles between mARC and xanthine oxidase reveals similar Kcat and Vmax values but more sustained NO formation from mARC, possibly because it is not vulnerable to autoinhibition via molybdenum desulfuration. The reduction of nitrite by mARC in the mitochondria may represent a new signaling pathway for NADH-dependent hypoxic NO production.
Insights
Mitochondrial amidoxime reducing component (mARC) enzymes reduce nitrite to nitric oxide (NO) using their molybdenum cofactor. This discovery reveals a new mitochondrial signaling pathway for hypoxic NO production.
Area of Science:
- Biochemistry
- Cellular Biology
- Enzymology
Background:
- Mitochondrial amidoxime reducing component (mARC) proteins are molybdopterin-containing enzymes with an unknown physiological role.
- Human mARC-1 and mARC-2 isoforms can reduce nitrite when in their reduced state.
Purpose of the Study:
- To investigate the physiological function of mARC proteins.
- To determine if mARC enzymes catalyze the reduction of nitrite to nitric oxide (NO).
Main Methods:
- Enzymatic assays measuring NO production from nitrite reduction by mARC-1 and mARC-2.
- Site-directed mutagenesis of the mARC-1 active site (Cys-273).
- Recombinant expression of mARC-1 in Escherichia coli with molybdenum or tungsten cofactor.
- Cellular expression of mARC-1 in HEK cells.
Main Results:
- mARC enzymes generate NO from nitrite via an electron transfer chain involving NADH, cytochrome b5, and NADH-dependent cytochrome b5 reductase.
- NO formation is dependent on the molybdenum cofactor, as demonstrated by abolished NO production in C273A mutated mARC-1 and tungsten-substituted mARC-1.
- Lowering pH from 7.5 to 6.5 increased the rate of NO formation.
- Cellular reduction of nitrite to NO by mARC-1 was confirmed in HEK cells.
- mARC exhibited sustained NO formation compared to xanthine oxidase, potentially due to resistance to autoinhibition.
Conclusions:
- Human mARC-1 and mARC-2 catalyze the reduction of nitrite to NO, utilizing their molybdenum cofactor.
- This enzymatic activity suggests a novel mitochondrial signaling pathway for NADH-dependent hypoxic NO production.
More Related Videos
Related Concept Videos
 01:46
Electron Transport Chain: Complex I and II
ROS generation is regulated and maintained at moderate levels necessary...
 01:30
The Electron Transport Chain
Inhibitors of the electron transport chain
Rotenone, a widely used pesticide, prevents electron transfer from Fe-S cluster to ubiquinone or Q...
 01:19
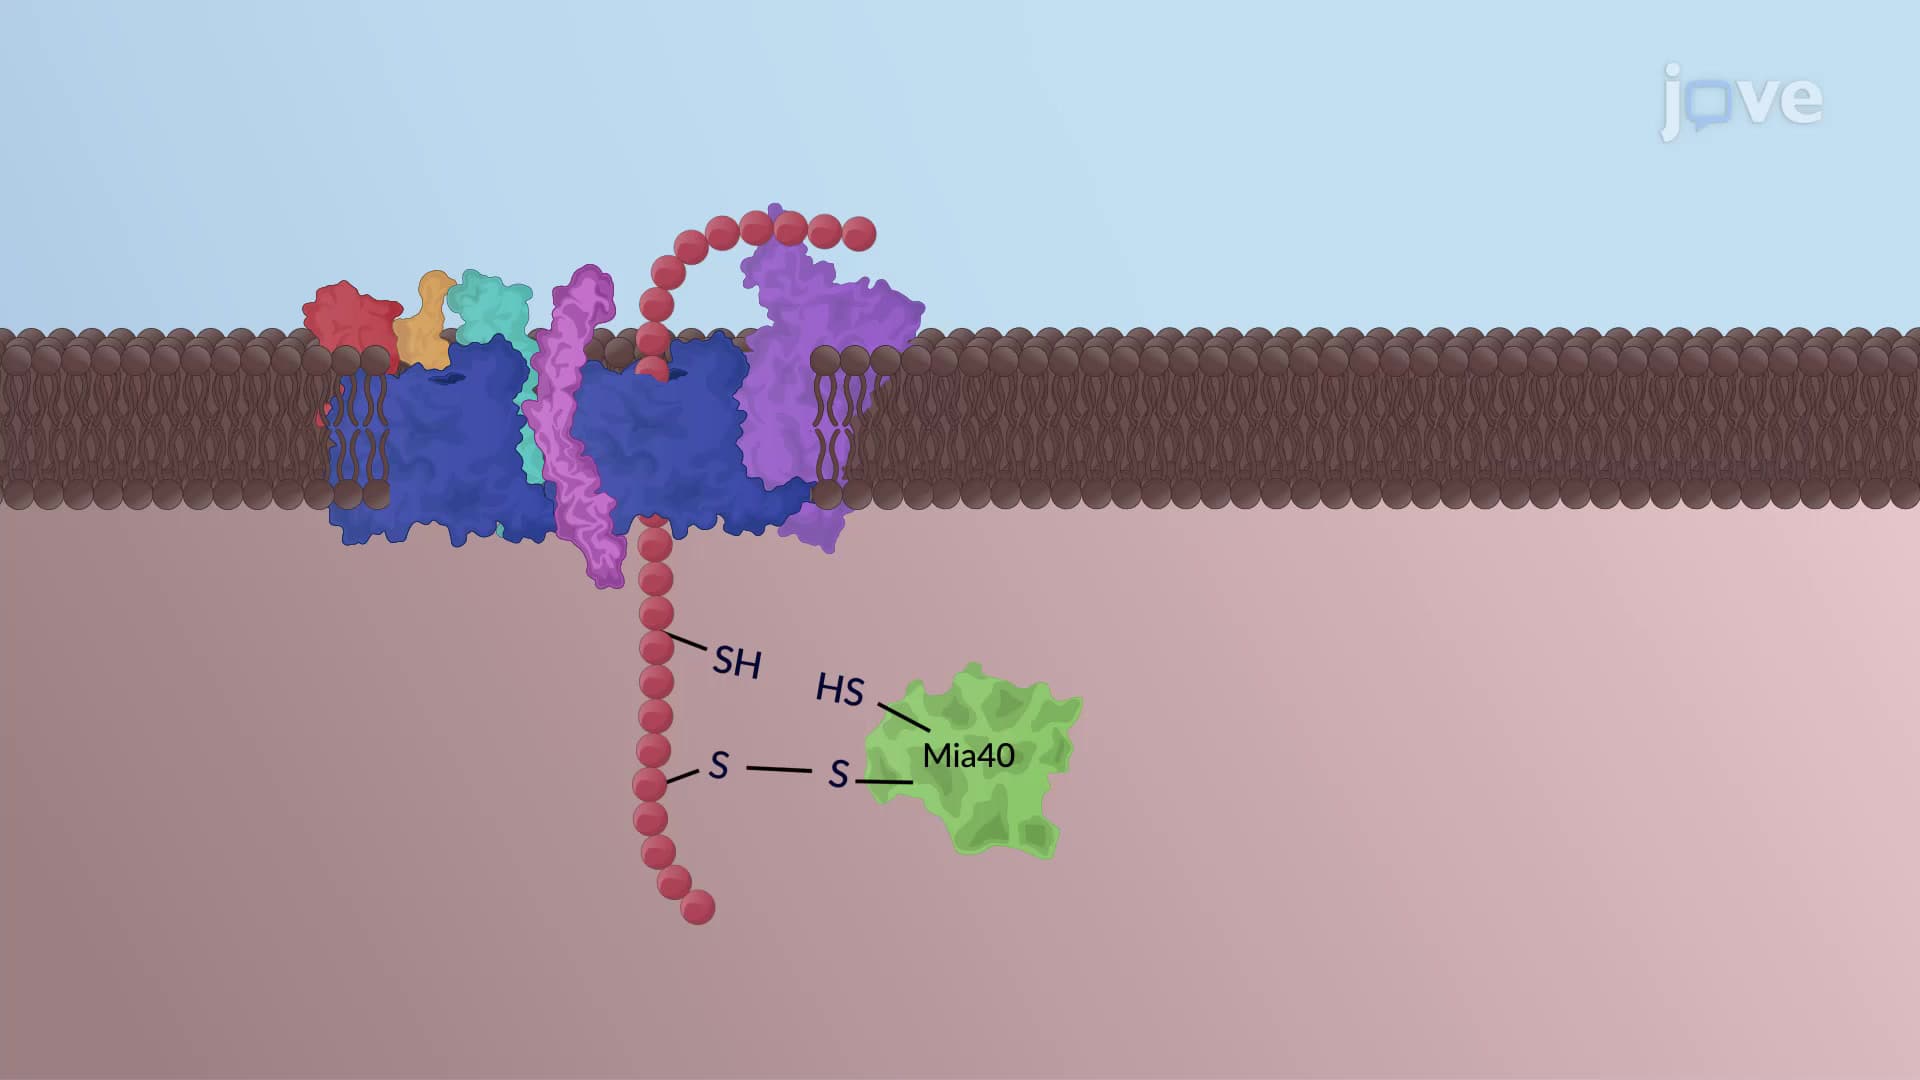
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:43
Electron Transport Chain: Complex III and IV
 01:41
The Supercomplexes in the Crista Membrane
 01:29
Role of Reduced Coenzymes NADH and FADH₂