Related Experiment Video
Updated: May 2, 2026
Reconstitution of Msp1 Extraction Activity with Fully Purified Components
Published on: August 10, 2021
A unique C-terminal domain allows retention of matrix metalloproteinase-27 in the endoplasmic reticulum
Antoine Cominelli1, Mathias Halbout, Francisca N'Kuli
1Cell Biology Unit, de Duve Institute, Université catholique de Louvain, Avenue Hippocrate 75, Box B1.75.05, B-1200, Brussels, Belgium.

Abstract:
Matrix metalloproteinase-27 (MMP-27) is poorly characterized. Sequence comparison suggests that a C-terminal extension (CTE) includes a potential transmembrane domain as in some membrane-type (MT)-MMPs. Having noticed that MMP-27 was barely secreted, we investigated its subcellular localization and addressed CTE contribution for MMP-27 retention. Intracellular MMP-27 was sensitive to endoglycosidase H. Subcellular fractionation and confocal microscopy evidenced retention of endogenous MMP-27 or recombinant rMMP-27 in the endoplasmic reticulum (ER) with locked exit across the intermediate compartment (ERGIC). Conversely, truncated rMMP-27 without CTE accessed downstream secretory compartments (ERGIC and Golgi) and was constitutively secreted. CTE addition to rMMP-10 (a secreted MMP) caused ER retention and blocked secretion. Addition of a PKA target sequence to the cytosolic C-terminus of transmembrane MT1-MMP/MMP-14 led to effective phosphorylation upon forskolin stimulation, but not for MMP-27, excluding transmembrane anchorage. Moreover, MMP-27 was protected from digestion by proteinase K. Finally, MT1-MMP/MMP-14 but neither endogenous nor recombinant MMP-27 partitioned in the detergent phase after Triton X-114 extraction, indicating that MMP-27 is not an integral membrane protein. In conclusion, MMP-27 is efficiently retained within the ER due to its unique CTE, which does not lead to stable membrane insertion. This could represent a novel ER retention system.
Insights
Matrix metalloproteinase-27 (MMP-27) is retained in the endoplasmic reticulum (ER) due to its C-terminal extension (CTE). This unique CTE prevents secretion and suggests a novel ER retention mechanism.
Area of Science:
- Biochemistry
- Cell Biology
- Molecular Biology
Background:
- Matrix metalloproteinase-27 (MMP-27) is poorly characterized.
- Sequence analysis suggests MMP-27 may possess a transmembrane domain via its C-terminal extension (CTE).
- MMP-27 exhibits minimal secretion, prompting investigation into its localization.
Purpose of the Study:
- Investigate the subcellular localization of MMP-27.
- Determine the role of the CTE in MMP-27 retention.
- Clarify the membrane association status of MMP-27.
Main Methods:
- Endoglycosidase H sensitivity assay.
- Subcellular fractionation and confocal microscopy.
- Recombinant protein expression and manipulation (CTE deletion/addition).
- Proteinase K digestion and Triton X-114 extraction.
Main Results:
- Endogenous and recombinant MMP-27 are retained in the endoplasmic reticulum (ER) and ER-Golgi intermediate compartment (ERGIC).
- Deletion of the CTE allows MMP-27 to access downstream secretory compartments and be secreted.
- Addition of the CTE to a secreted MMP (MMP-10) causes ER retention.
- MMP-27 lacks transmembrane anchorage and is not an integral membrane protein.
Conclusions:
- MMP-27 is efficiently retained within the ER via its unique CTE.
- The CTE mediates ER retention without stable membrane insertion, representing a novel ER retention system.
- MMP-27's localization is distinct from typical membrane-type matrix metalloproteinases.
More Related Videos
 07:32
Bacterial Expression and Purification of Human Matrix Metalloproteinase-3 using Affinity Chromatography
Published on: March 30, 2022
 13:40
Live Cell Calcium Imaging Combined with siRNA Mediated Gene Silencing Identifies Ca2+ Leak Channels in the ER Membrane and their Regulatory Mechanisms
Published on: July 7, 2011
Related Concept Videos
 01:26
Insertion of Single-pass Transmembrane Proteins in the RER
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
 01:19
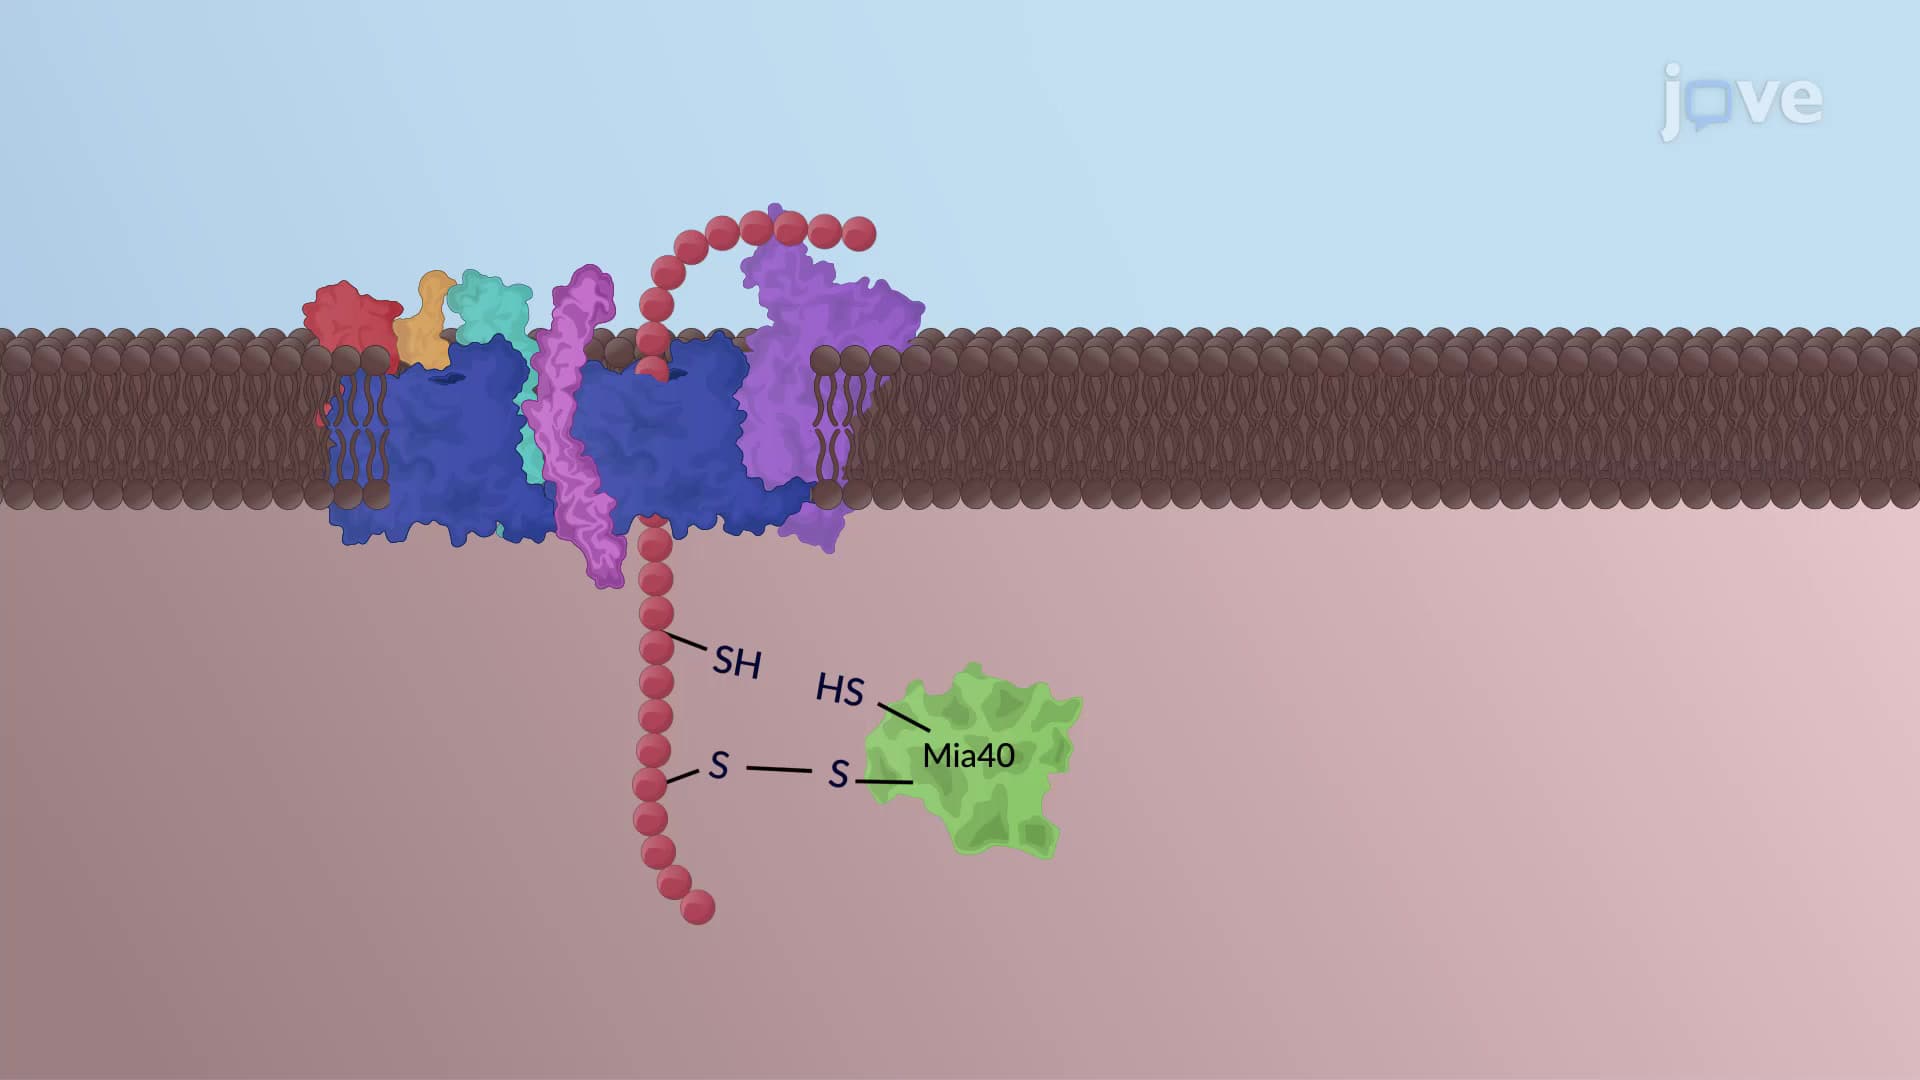
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:23
Role of Matrix Metalloproteases in Degradation of ECM
 01:29
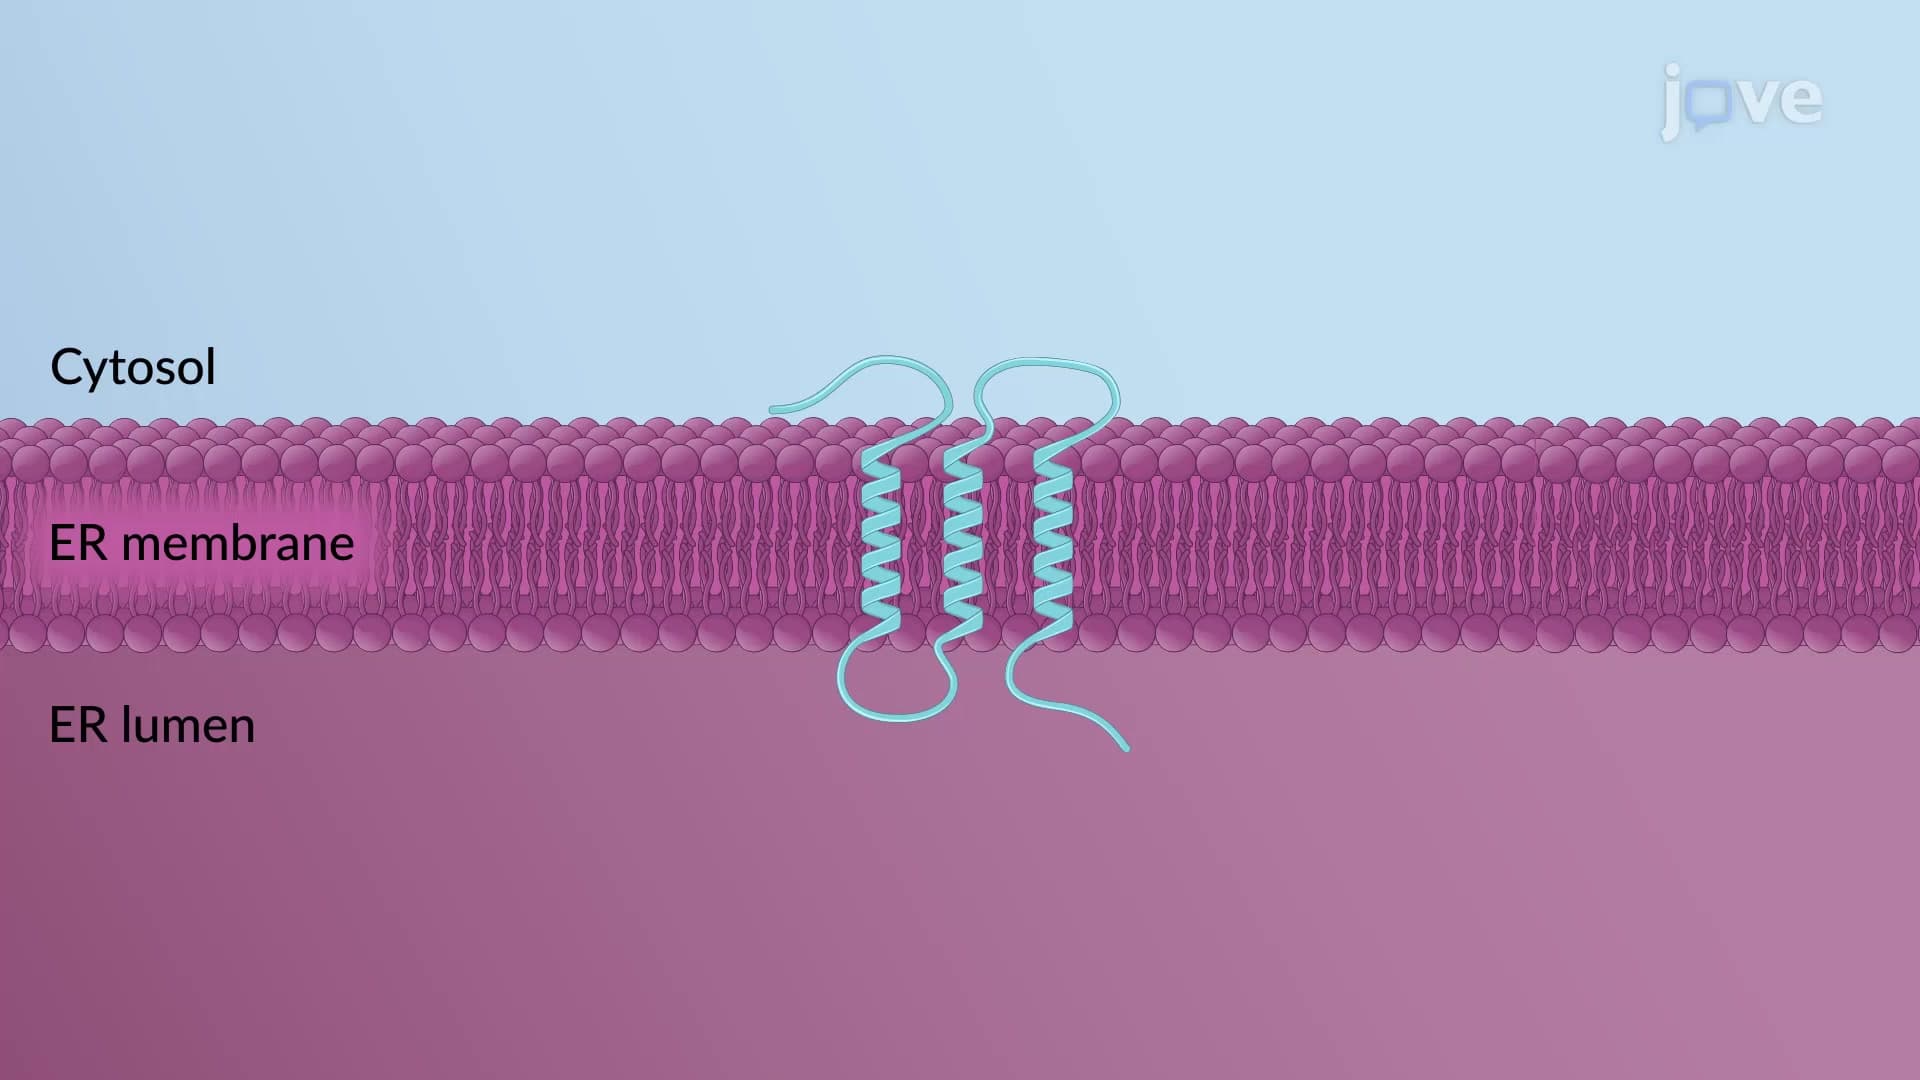
Insertion of Multi-pass Transmembrane Proteins in the RER
The multipass transmembrane proteins are the type IV integral membrane proteins with multiple topogenic sequences determining their spatial arrangement in the ER membrane. Nearly all multipass proteins lack a cleavable signal sequence and use...
 01:45
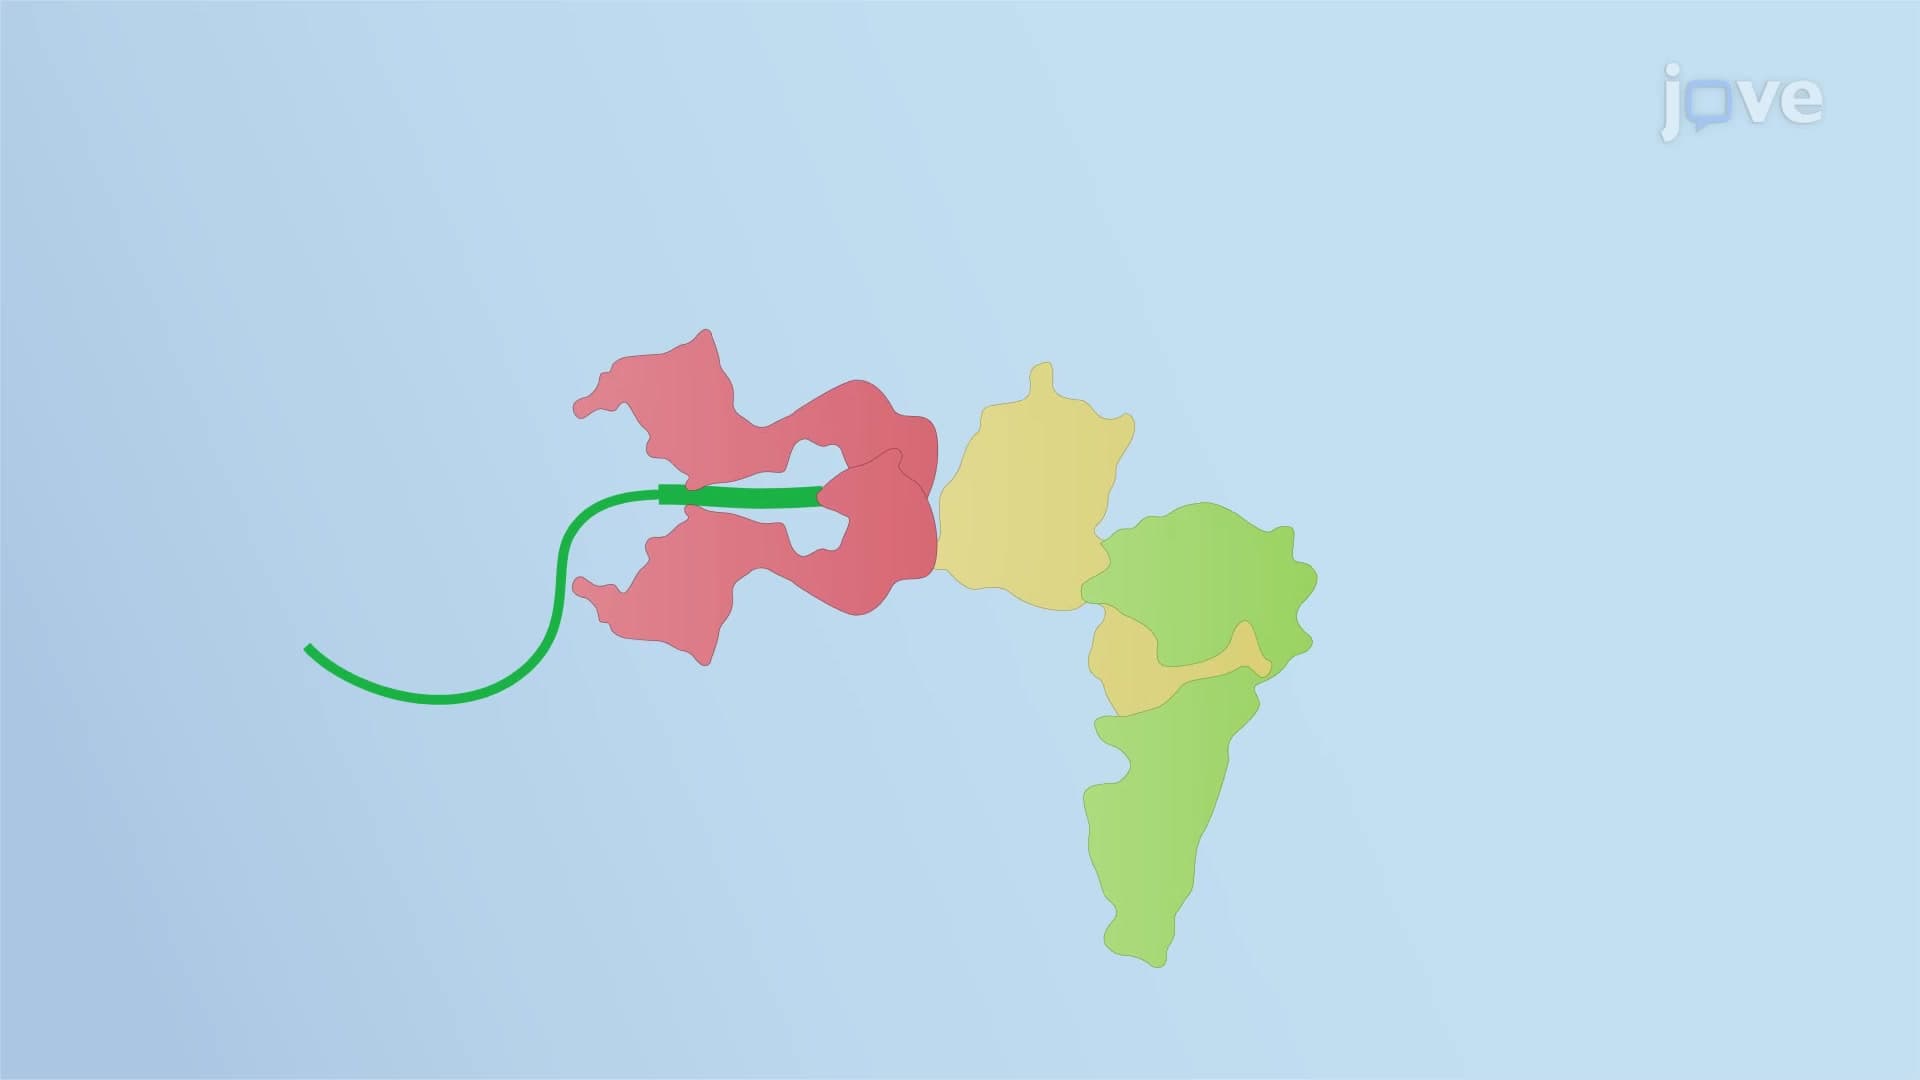
Tail-anchoring of Proteins in the ER Membrane
 01:12
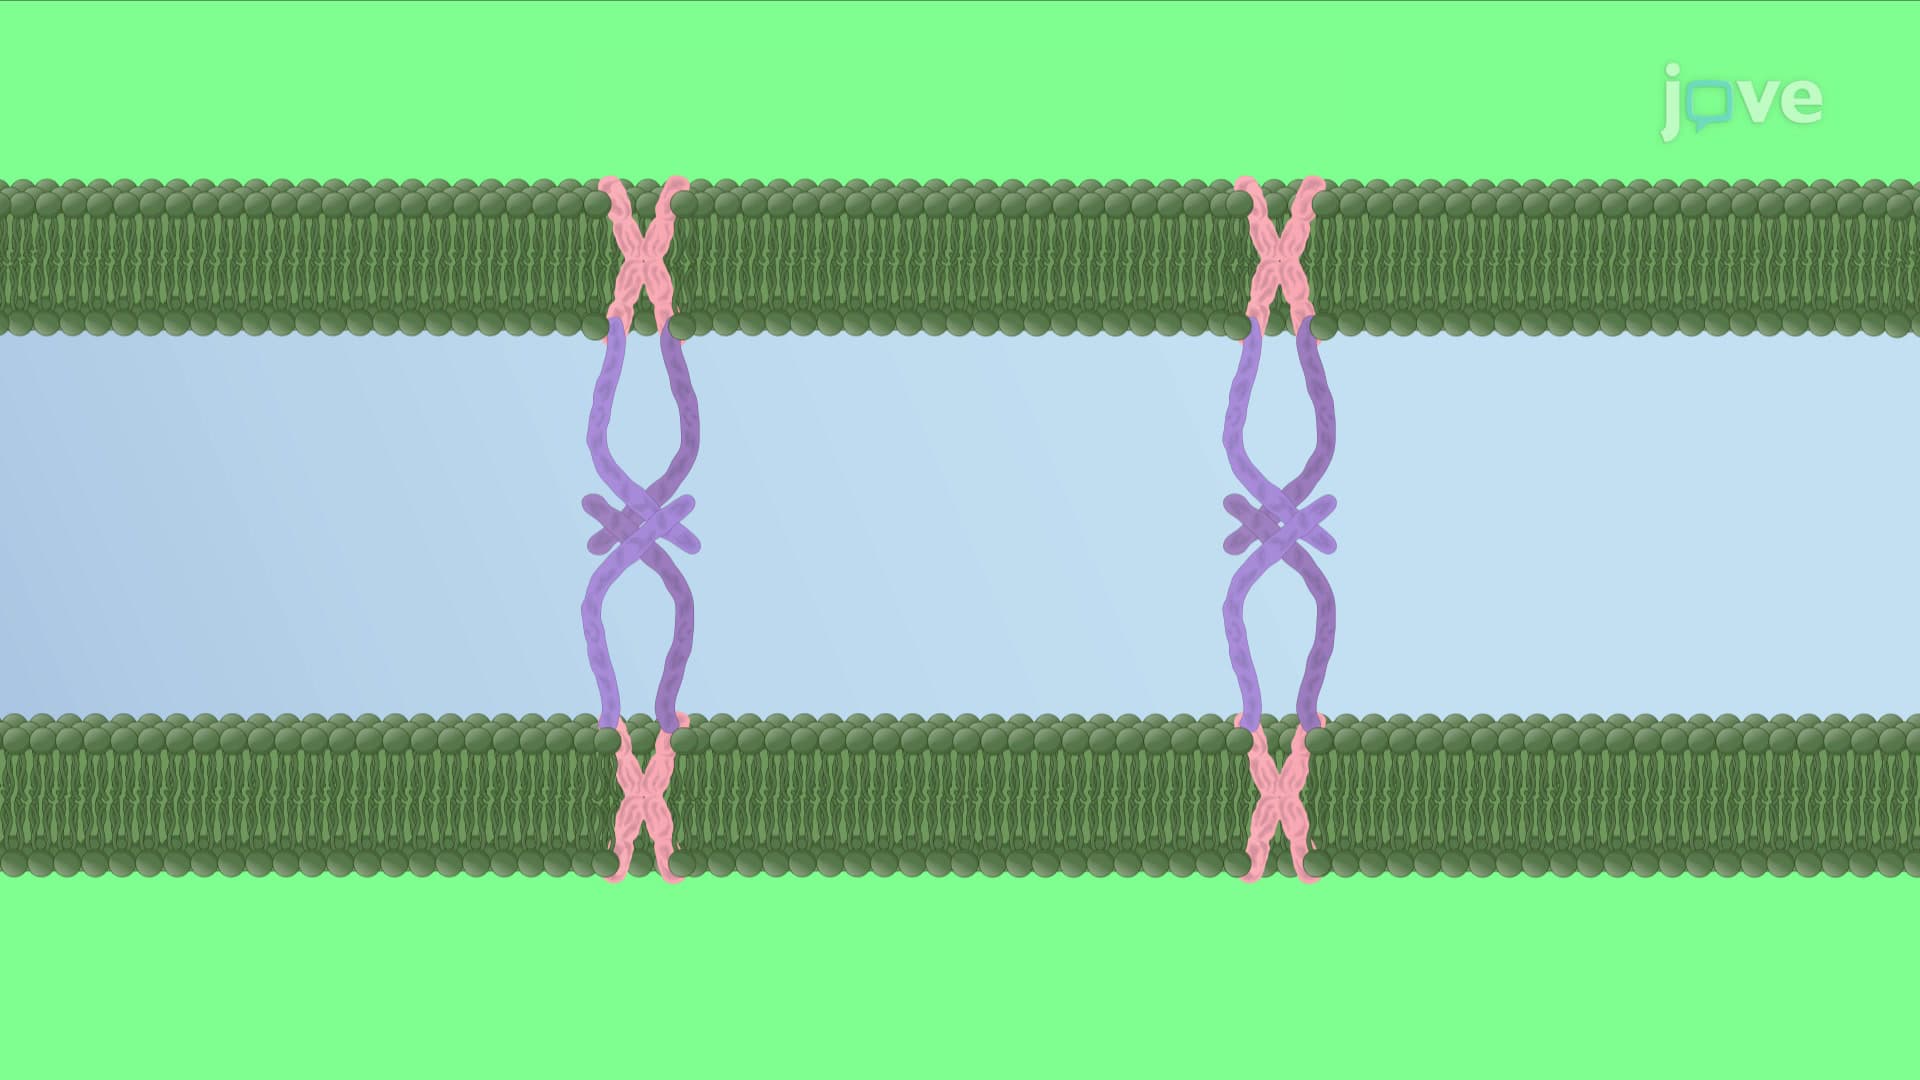
Golgi Matrix Proteins
One of the first identified Golgi matrix proteins was GM130, a rod-like protein located in the cis-Golgi. Subsequently, many Golgi...