Related Experiment Video
Updated: Mar 30, 2026
Using Scaffold Liposomes to Reconstitute Lipid-proximal Protein-protein Interactions In Vitro
Published on: January 11, 2017
Phosphatidylserine-Dependent Catalysis of Stalk and Pore Formation by Synaptobrevin JMR-TMD Peptide
Pradip K Tarafdar1, Hirak Chakraborty1, Michael J Bruno1
1Department of Biochemistry and Biophysics, University of North Carolina at Chapel Hill, Chapel Hill, North Carolina; Molecular and Cellular Biophysics Program, University of North Carolina at Chapel Hill, Chapel Hill, North Carolina.

Abstract:
Although the importance of a SNARE complex in neurotransmitter release is widely accepted, there exist different views on how the complex promotes fusion. One hypothesis is that the SNARE complex's ability to bring membranes into contact is sufficient for fusion, another points to possible roles of juxtamembrane regions (JMRs) and transmembrane domains (TMDs) in catalyzing lipid rearrangement, and another notes the complex's presumed ability to bend membranes near the point of contact. Here, we performed experiments with highly curved vesicles brought into contact using low concentrations of polyethylene glycol (PEG) to investigate the influence of the synaptobrevin (SB) TMD with an attached JMR (SB-JMR-TMD) on the rates of stalk and pore formation during vesicle fusion. SB-JMR-TMD enhanced the rates of stalk and fusion pore (FP) formation in a sharply sigmoidal fashion. We observed an optimal influence at an average of three peptides per vesicle, but only with phosphatidylserine (PS)-containing vesicles. Approximately three SB-JMR-TMDs per vesicle optimally ordered the bilayer interior and excluded water in a similar sigmoidal fashion. The catalytic influences of hexadecane and SB-JMR-TMD on fusion kinetics showed little in common, suggesting different mechanisms. Both kinetic and membrane structure measurements support the hypotheses that SB-JMR-TMD 1) catalyzes initial intermediate formation as a result of its basic JMR disrupting ordered interbilayer water and permitting closer interbilayer approach, and 2) catalyzes pore formation by forming a membrane-spanning complex that increases curvature stress at the circumference of the hemifused diaphragm of the prepore intermediate state.
More Related Videos
 09:19
Analysis of SNARE-mediated Membrane Fusion Using an Enzymatic Cell Fusion Assay
Published on: October 19, 2012
 10:58
SNARE-mediated Fusion of Single Proteoliposomes with Tethered Supported Bilayers in a Microfluidic Flow Cell Monitored by Polarized TIRF Microscopy
Published on: August 24, 2016
Related Concept Videos
 01:43
SNAREs and Membrane Fusion
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
 01:32
Pinching-off of Coated Vesicles
 00:59
Mechanisms of Membrane Domain Formation
Another mechanism for membrane domain formation involves membrane proteins interacting with...
 01:18
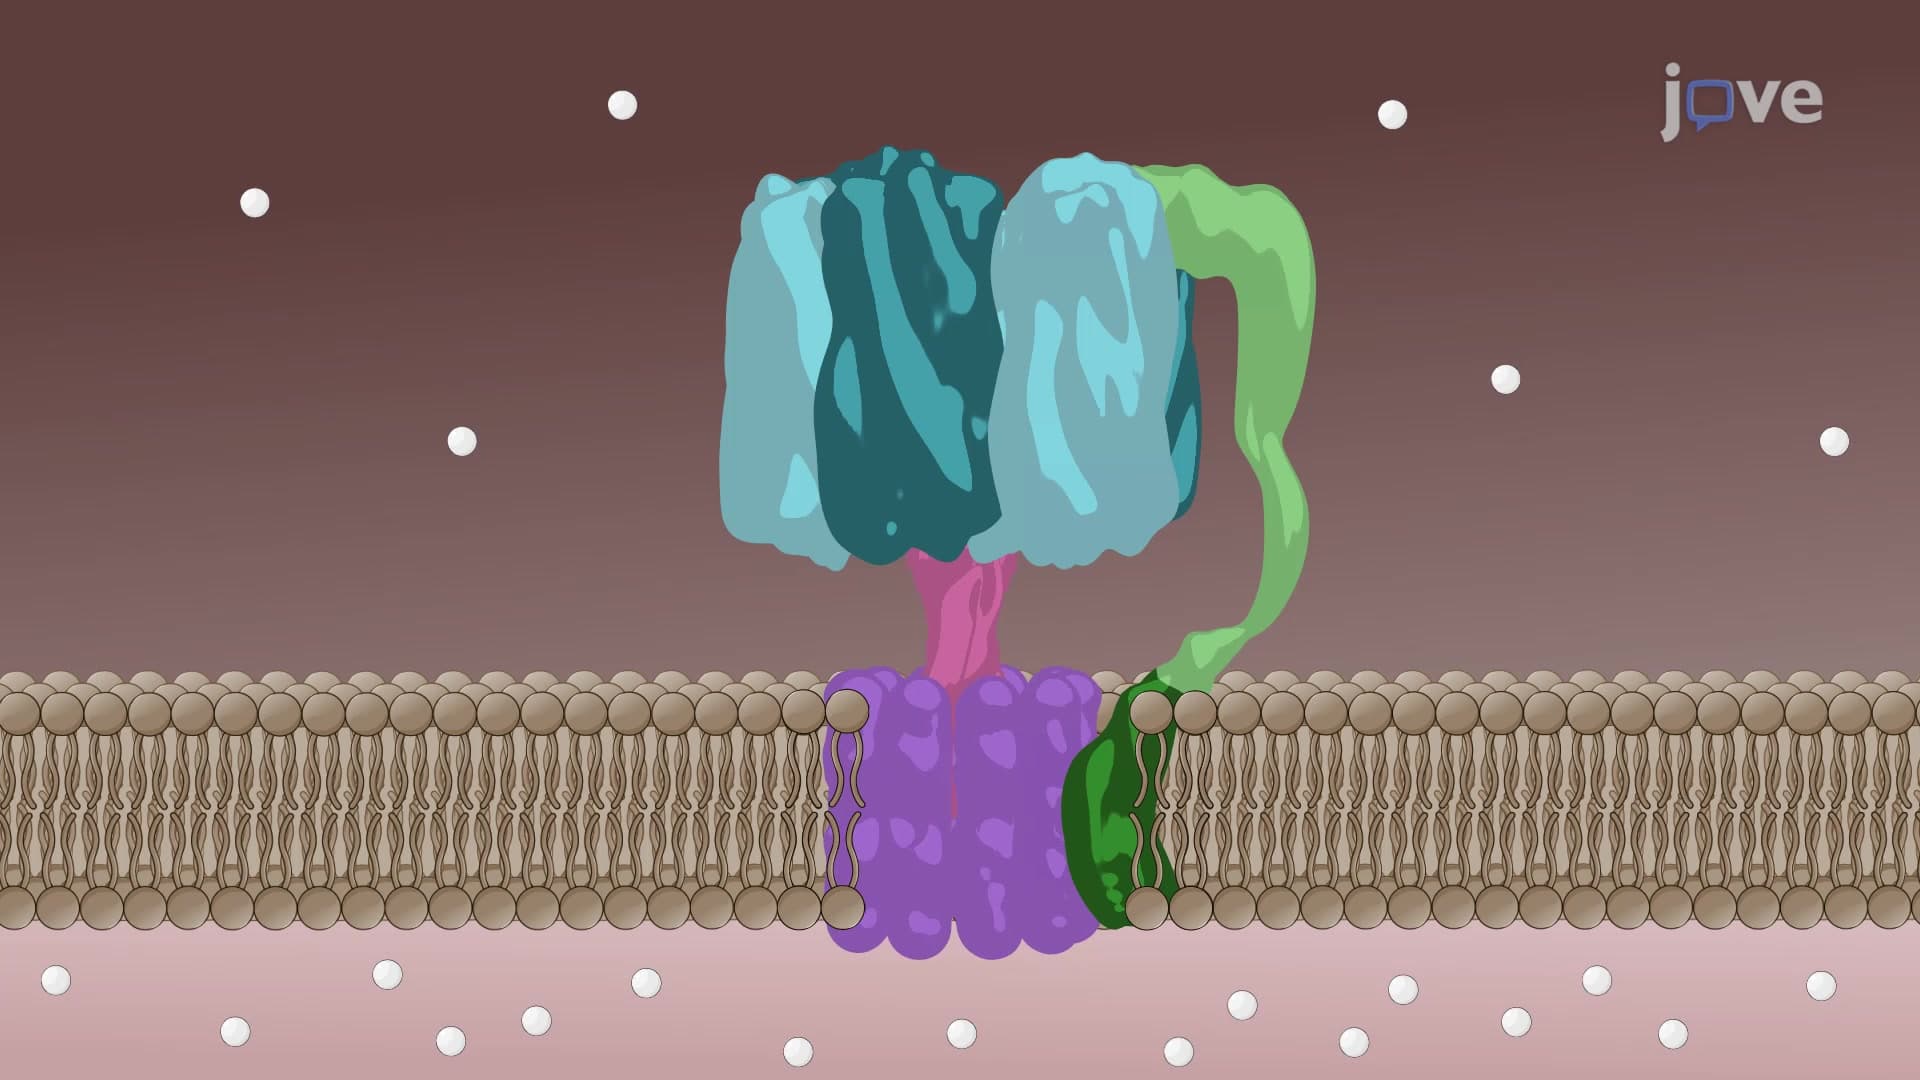
ATP Synthase: Structure
 01:12
Clathrin Coated Vesicles
 01:28
Protein Translocation Machinery on the ER Membrane
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the...