Related Experiment Video
Updated: Mar 12, 2026

A Fluorogenic Peptide Cleavage Assay to Screen for Proteolytic Activity: Applications for coronavirus spike protein activation
Published on: January 9, 2019
SARS-CoV 3CL protease cleaves its C-terminal autoprocessing site by novel subsite cooperativity
Tomonari Muramatsu1,2, Chie Takemoto3,4, Yong-Tae Kim3
1RIKEN Systems and Structural Biology Center, Tsurumi, Yokohama 230-0045, Japan; tomonari.muramatsu@riken.jp yokoyama@riken.jp.

Abstract:
The 3C-like protease (3CLpro) of severe acute respiratory syndrome coronavirus (SARS-CoV) cleaves 11 sites in the polyproteins, including its own N- and C-terminal autoprocessing sites, by recognizing P4-P1 and P1'. In this study, we determined the crystal structure of 3CLpro with the C-terminal prosequence and the catalytic-site C145A mutation, in which the enzyme binds the C-terminal prosequence of another molecule. Surprisingly, Phe at the P3' position [Phe(P3')] is snugly accommodated in the S3' pocket. Mutations of Phe(P3') impaired the C-terminal autoprocessing, but did not affect N-terminal autoprocessing. This difference was ascribed to the P2 residue, Phe(P2) and Leu(P2), in the C- and N-terminal sites, as follows. The S3' subsite is formed by Phe(P2)-induced conformational changes of 3CLpro and the direct involvement of Phe(P2) itself. In contrast, the N-terminal prosequence with Leu(P2) does not cause such conformational changes for the S3' subsite formation. In fact, the mutation of Phe(P2) to Leu in the C-terminal autoprocessing site abolishes the dependence on Phe(P3'). These mechanisms explain why Phe is required at the P3' position when the P2 position is occupied by Phe rather than Leu, which reveals a type of subsite cooperativity. Moreover, the peptide consisting of P4-P1 with Leu(P2) inhibits protease activity, whereas that with Phe(P2) exhibits a much smaller inhibitory effect, because Phe(P3') is missing. Thus, this subsite cooperativity likely exists to avoid the autoinhibition of the enzyme by its mature C-terminal sequence, and to retain the efficient C-terminal autoprocessing by the use of Phe(P2).
Related Concept Videos
 01:33
Coat Assembly and GTPases
Coat assembly depends on the local availability of phosphatidylinositol phosphates or PIPs and GTP-binding proteins. Adaptor proteins, which link the coat proteins to the membrane, bind to these PIPs and play a crucial role in controlling...
 01:17
The Proteasome Structure
The proteasome is an...
 02:18
The Proteasome
In this pathway, the target proteins are first tagged with small proteins called ubiquitin. A series of enzymes carry out the ubiquitination of the target proteins - E1 (ubiquitin-activating enzyme), E2 (ubiquitin-conjugating enzyme), and E3...
 01:13
The Proteasome
In this pathway, the target proteins are first tagged with small proteins called ubiquitin. This involves participation of a series of enzymes including— E1 (ubiquitin-activating enzyme), E2 (ubiquitin-conjugating enzyme), and E3...
 01:19
Allosteric Proteins-ATCase
Aspartate transcarbamoylase (ATCase) is a cytosolic enzyme that catalyzes the condensation of L-aspartate and carbamoyl phosphate to N-carbamoyl-L-aspartate. This reaction is the first step in pyrimidine biosynthesis. UTP and CTP, the end products of the pyrimidine synthesis...
 01:14
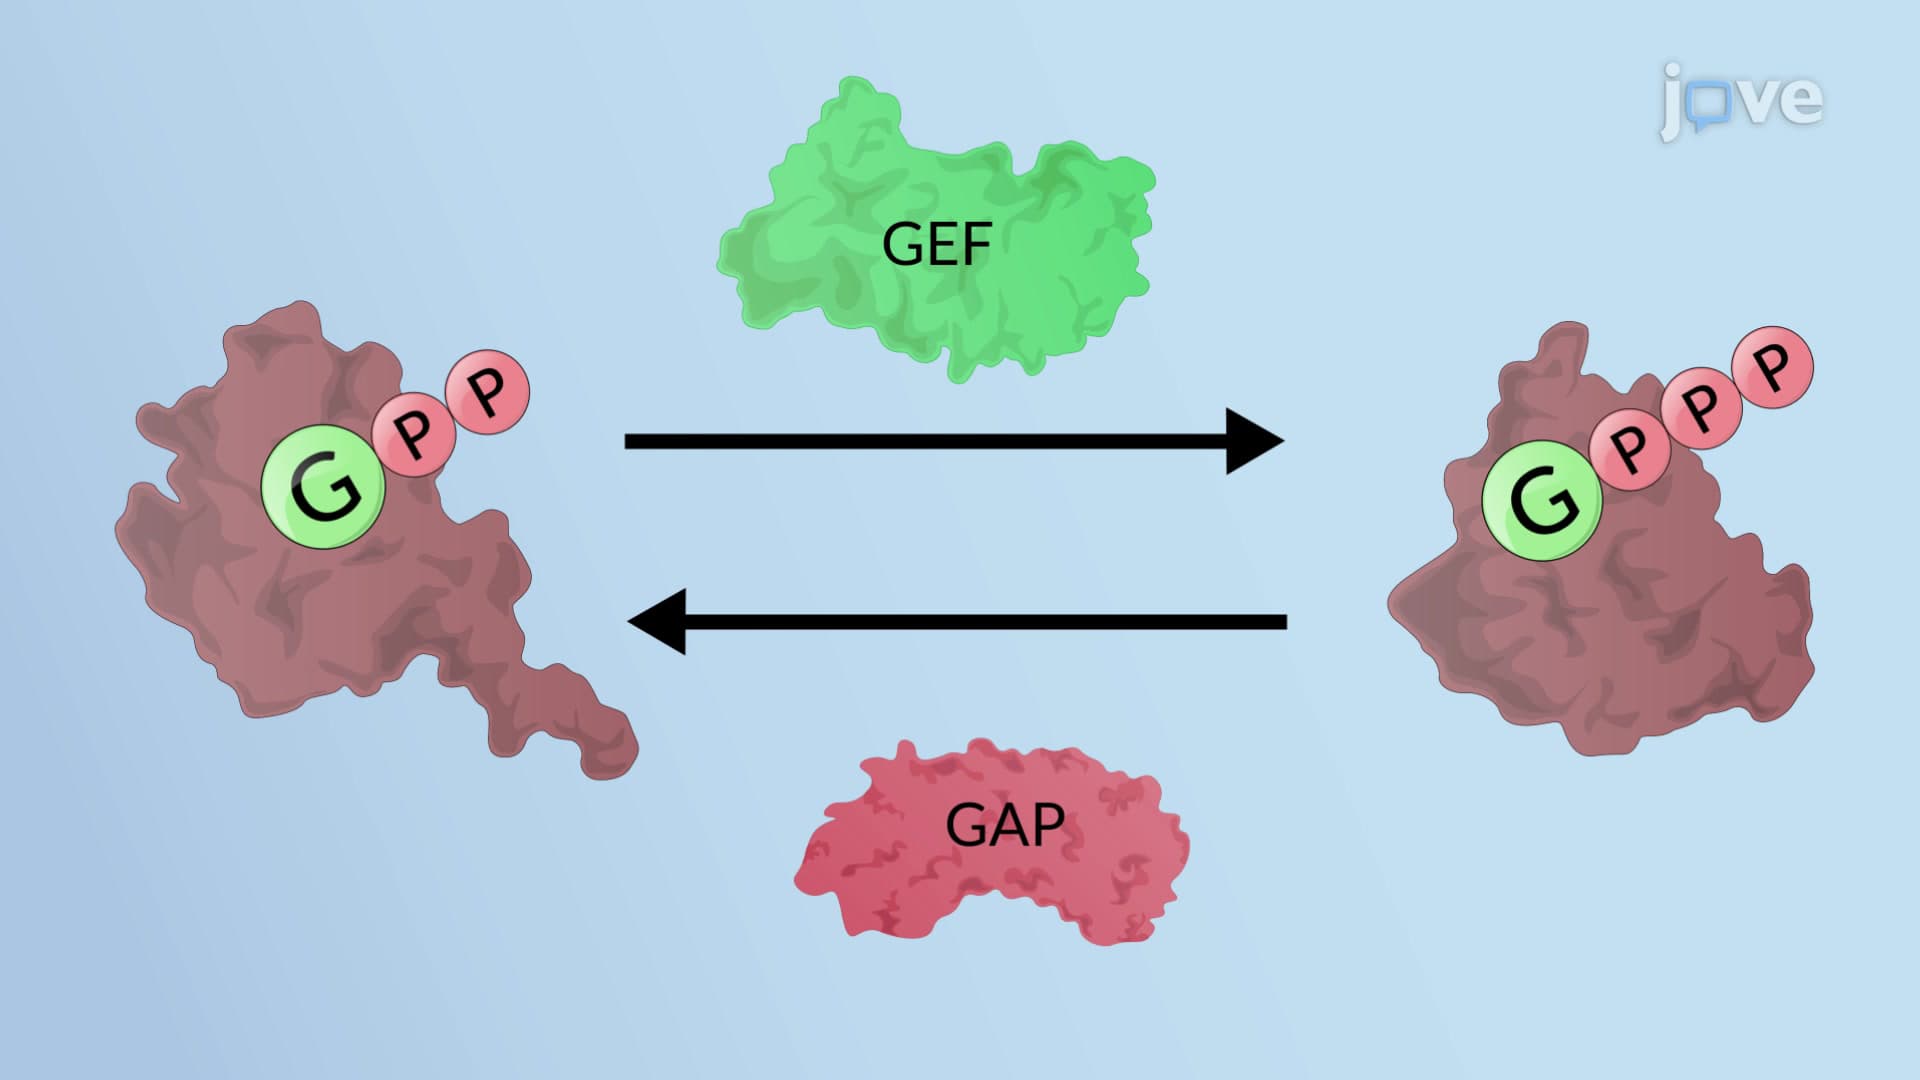
Rab Proteins
Rab proteins switch between a cytosolic, GDP-bound inactive state and a membrane-anchored, GTP-bound active state. By themselves, Rabs show slow rates of GDP/GTP exchange and GTP hydrolysis. Thus, Rab proteins are considered...