Related Experiment Video
Updated: Jul 21, 2026

Sedimentation Equilibrium of a Small Oligomer-forming Membrane Protein: Effect of Histidine Protonation on Pentameric Stability
Published on: April 2, 2015
The dynamics of multimer formation of the amphiphilic hydrophobin protein HFBII
M S Grunér1, A Paananen2, G R Szilvay2
1Department of Bioproducts and Biosystems, Aalto University, Kemistintie 1, 02150 Espoo, Finland; VTT Technical Research Centre of Finland Ltd, Tietotie 2, 02150 Espoo, Finland.

Abstract:
Hydrophobins are surface-active proteins produced by filamentous fungi. They have amphiphilic structures and form multimers in aqueous solution to shield their hydrophobic regions. The proteins rearrange at interfaces and self-assemble into films that can show a very high degree of structural order. Little is known on dynamics of multimer interactions in solution and how this is affected by other components. In this work we examine the multimer dynamics by stopped-flow fluorescence measurements and Förster Resonance Energy Transfer (FRET) using the class II hydrophobin HFBII. The half-life of exchange in the multimer state was 0.9s at 22°C with an activation energy of 92kJ/mol. The multimer exchange process of HFBII was shown to be significantly affected by the closely related HFBI hydrophobin, lowering both activation energy and half-life for exchange. Lower molecular weight surfactants interacted in very selective ways, but other surface active proteins did not influence the rates of exchange. The results indicate that the multimer formation is driven by specific molecular interactions that distinguish different hydrophobins from each other.
Related Concept Videos
 02:41
Protein Complex Assembly
Many viruses self-assemble into a fully functional unit using the infected host cell to...
 01:57
Protein Complexes with Interchangeable Parts
The SCF ubiquitin ligase is a protein complex of five individual proteins. This complex attaches ubiquitin to other target proteins to mark them for degradation. In order to...
 01:11
Formation of Higher-order Actin Filaments
The high-order actin networks...
 00:57
Formation of Intermediate Filaments
 01:09
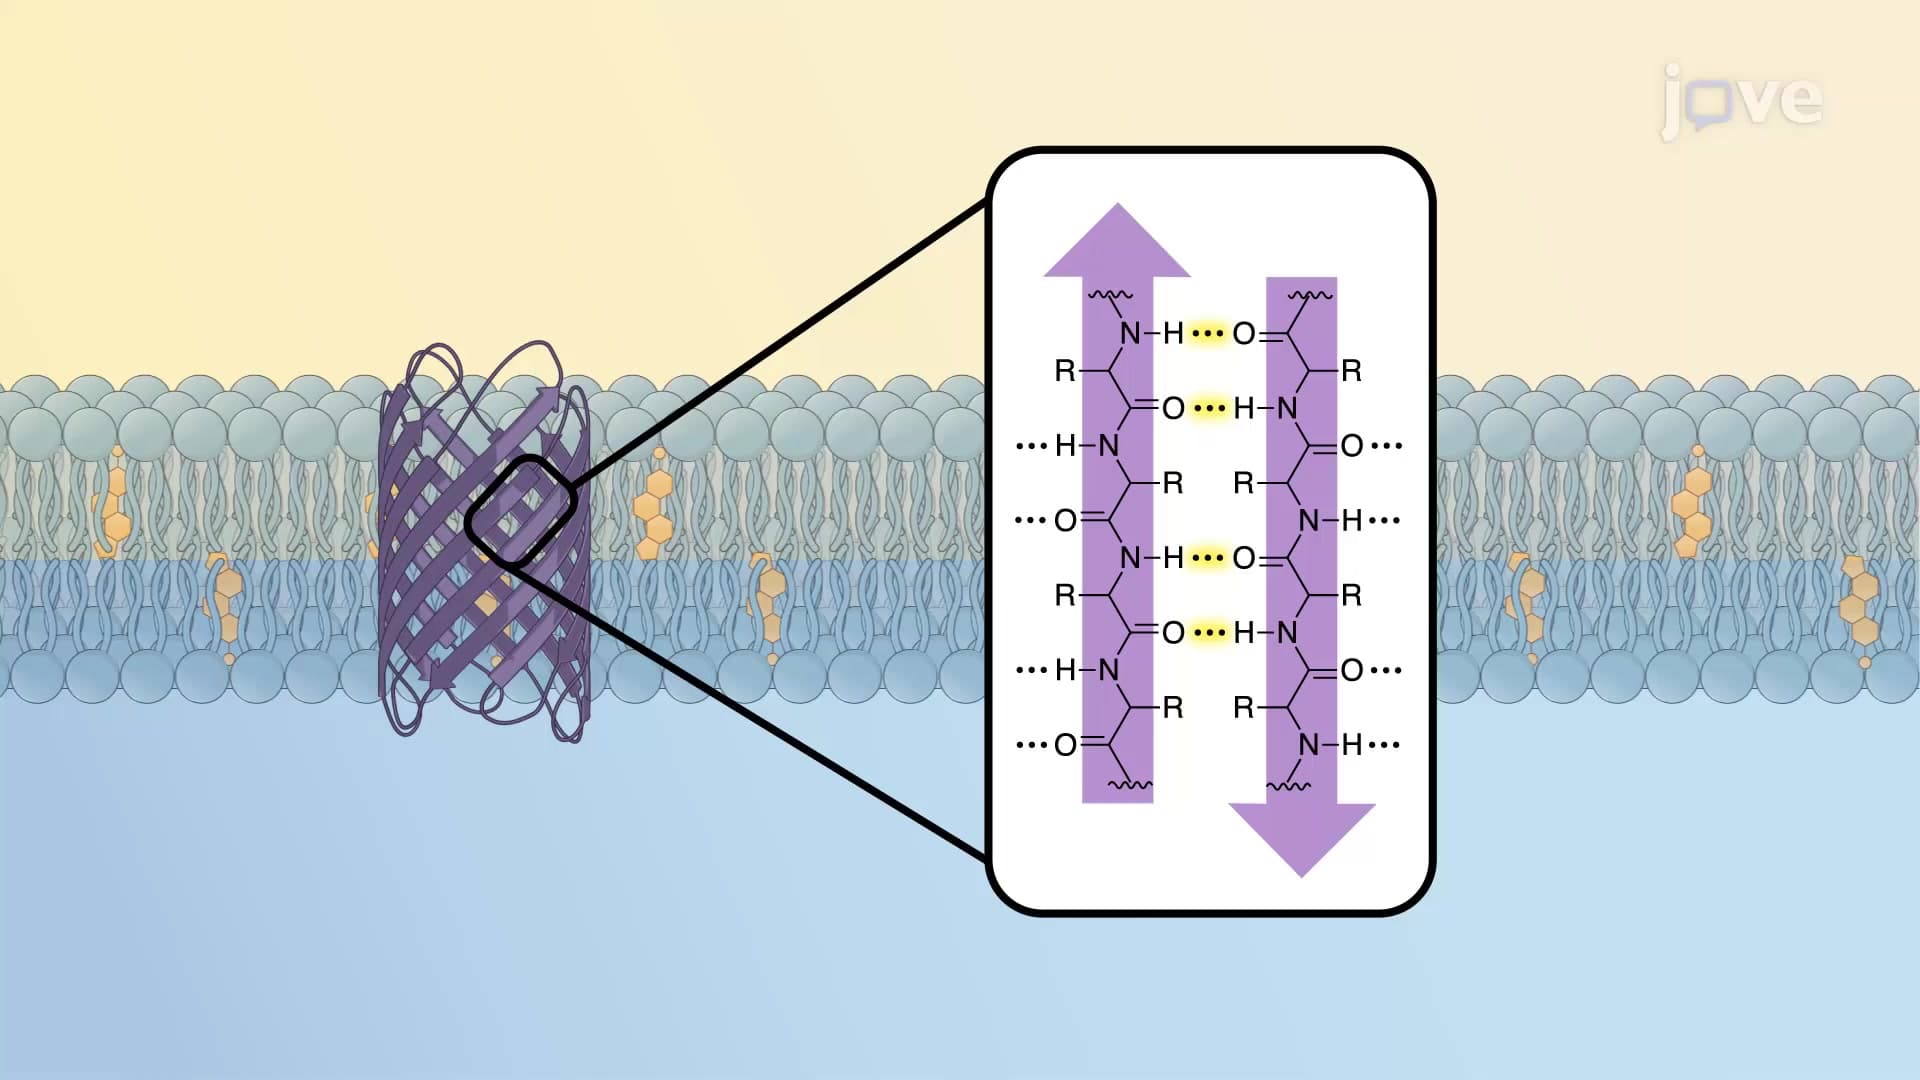
Multi-pass Transmembrane Proteins and β-barrels
α-Helix containing multi-pass transmembrane proteins
Multi-pass transmembrane proteins such as G-protein-linked receptors (GPCRs) and...
 00:59
Mechanisms of Membrane Domain Formation
Another mechanism for membrane domain formation involves membrane proteins interacting with cytoskeletal...