Related Experiment Video
Updated: Feb 25, 2026
Functional Characterization of RING-Type E3 Ubiquitin Ligases In Vitro and In Planta
Published on: December 5, 2019
Structural insights into the mechanism and E2 specificity of the RBR E3 ubiquitin ligase HHARI
Lingmin Yuan1,2, Zongyang Lv1,2, James H Atkison1,2
1Department of Biochemistry & Molecular Biology, Medical University of South Carolina, Charleston, SC, 29425, USA.

RING-in-between-RING (RBR) ubiquitin (Ub) E3 ligases function with Ub E2s through a RING/HECT hybrid mechanism to conjugate Ub to target proteins. Here, we report the crystal structure of the RBR E3, HHARI, in complex with a UbcH7 ~ Ub thioester mimetic which reveals the molecular basis for the specificity of this cognate E2/RBR E3 pair. The structure also reveals mechanistically important conformational changes in the RING1 and UBA-like domains of HHARI that accompany UbcH7 ~ Ub binding and provides a molecular basis by which HHARI recruits E2 ~ Ub in an 'open' conformation. In addition to optimally functioning with an E2 that solely performs transthiolation, our data suggests that HHARI prevents spurious discharge of Ub from E2 to lysine residues by: (1) harboring structural elements that block E2 ~ Ub from adopting a 'closed' conformation and (2) participating in contacts to ubiquitin that promote an open E2 ~ Ub conformation.HHARI is a RING-in-between-RING (RBR) ubiquitin (Ub) E3 ligase. Here the authors present the crystal structure of HHARI with the UbcH7 ~ Ub thioester intermediate mimetic, which reveals that HHARI binds this E2 ~ Ub in an open conformation and explains the specificity of this cognate RBR E3/E2 pair.
RING-in-between-RING (RBR) ubiquitin (Ub) E3 ligases function with Ub E2s through a RING/HECT hybrid mechanism to conjugate Ub to target proteins. Here, we report the crystal structure of the RBR E3, HHARI, in complex with a UbcH7 ~ Ub thioester mimetic which reveals the molecular basis for the specificity of this cognate E2/RBR E3 pair. The structure also reveals mechanistically important conformational changes in the RING1 and UBA-like domains of HHARI that accompany UbcH7 ~ Ub binding and provides a molecular basis by which HHARI recruits E2 ~ Ub in an 'open' conformation. In addition to optimally functioning with an E2 that solely performs transthiolation, our data suggests that HHARI prevents spurious discharge of Ub from E2 to lysine residues by: (1) harboring structural elements that block E2 ~ Ub from adopting a 'closed' conformation and (2) participating in contacts to ubiquitin that promote an open E2 ~ Ub conformation.HHARI is a RING-in-between-RING (RBR) ubiquitin (Ub) E3 ligase. Here the authors present the crystal structure of HHARI with the UbcH7 ~ Ub thioester intermediate mimetic, which reveals that HHARI binds this E2 ~ Ub in an open conformation and explains the specificity of this cognate RBR E3/E2 pair.
Related Concept Videos
 02:04
Covalently Linked Protein Regulators
These groups modify specific amino acids in a protein....
 01:32
Export of Misfolded Proteins out of the ER
 02:58
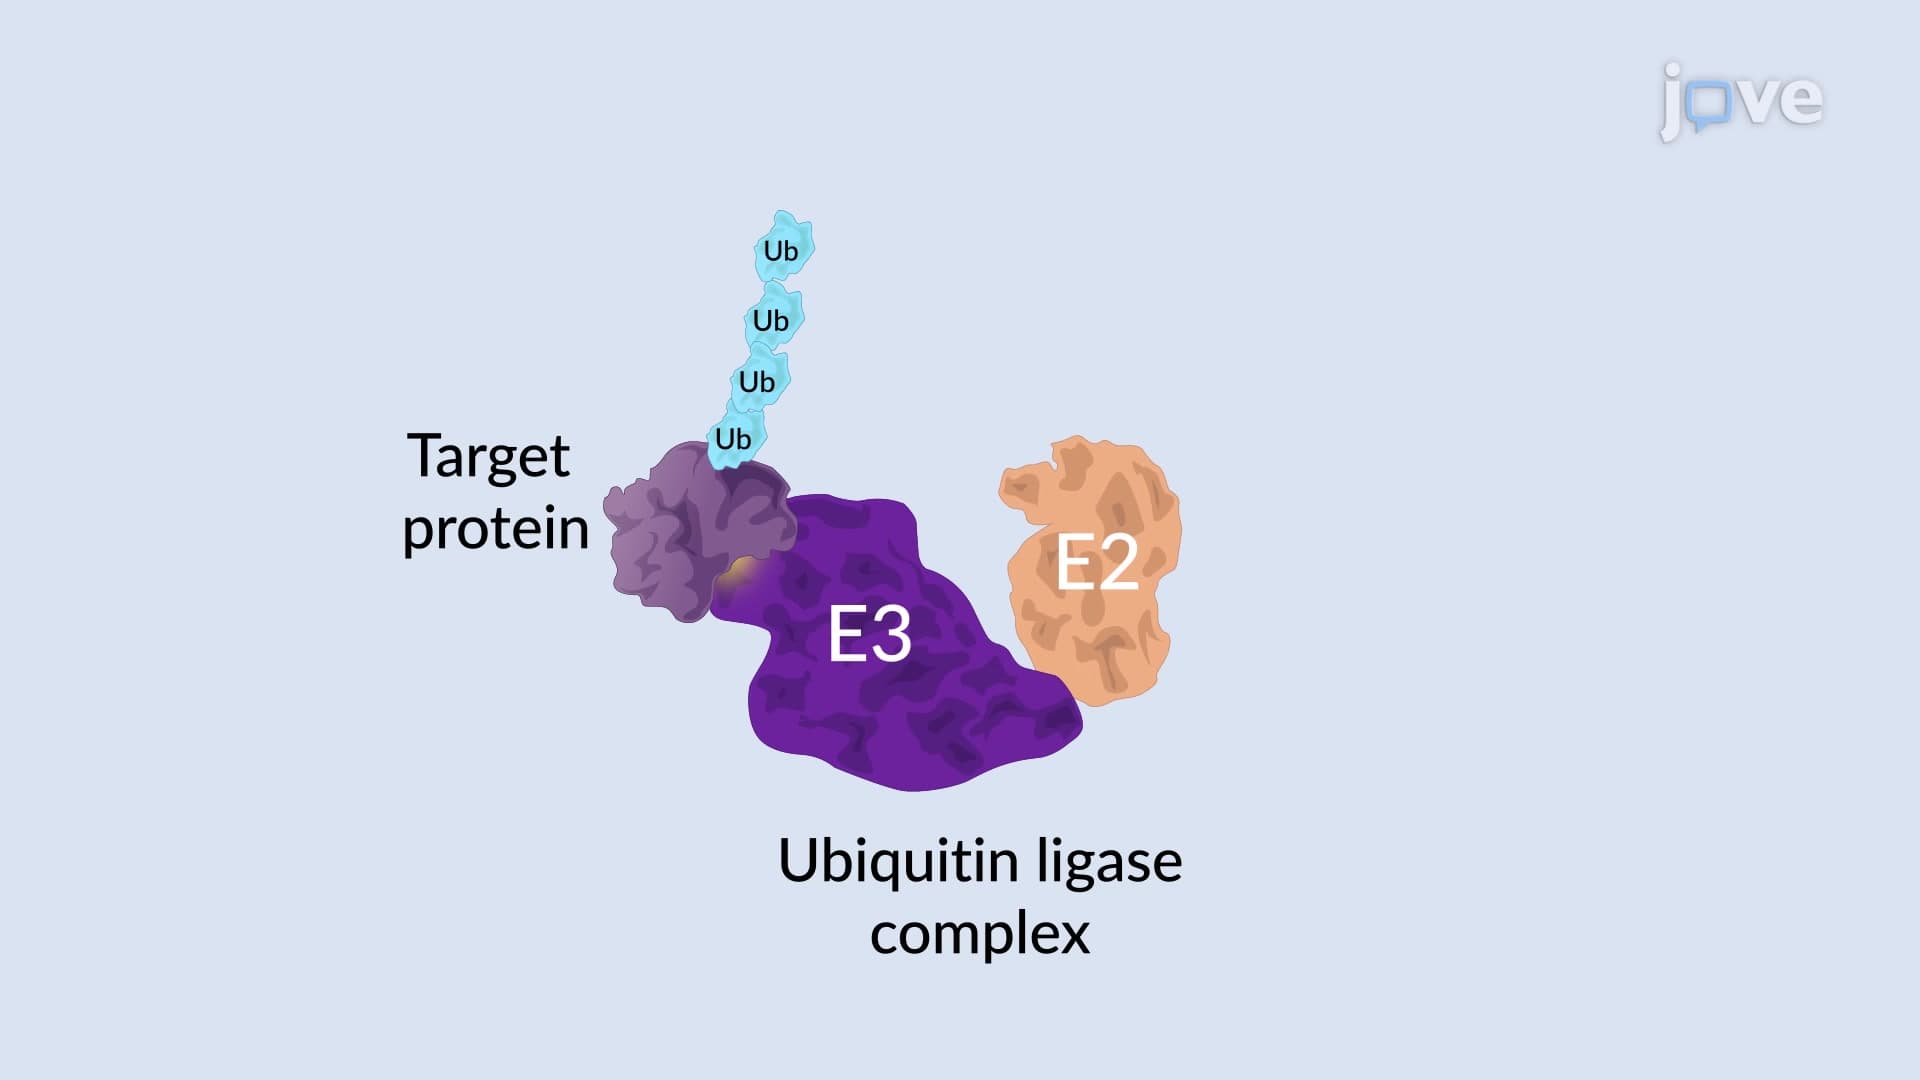
Regulated Protein Degradation
Protein degradation plays two important roles in the cells. It helps to protect cells from misfolded or damaged proteins before they lead to a...
 02:45
E2 Reaction: Kinetics and Mechanism
 01:31
Regulation of the Unfolded Protein Response
 02:46
E1 Reaction: Kinetics and Mechanism