
Vps13-Mcp1 interact at vacuole-mitochondria interfaces and bypass ER-mitochondria contact sites
Arun T John Peter1, Beatrice Herrmann1, Diana Antunes2
1ETH Zürich, Institute of Biochemistry, Zürich, Switzerland.

Abstract:
Membrane contact sites between endoplasmic reticulum (ER) and mitochondria, mediated by the ER-mitochondria encounter structure (ERMES) complex, are critical for mitochondrial homeostasis and cell growth. Defects in ERMES can, however, be bypassed by point mutations in the endosomal protein Vps13 or by overexpression of the mitochondrial protein Mcp1. How this bypass operates remains unclear. Here we show that the mitochondrial outer membrane protein Mcp1 functions in the same pathway as Vps13 by recruiting it to mitochondria and promoting its association to vacuole-mitochondria contacts. Our findings support a model in which Mcp1 and Vps13 work as functional effectors of vacuole-mitochondria contact sites, while tethering is mediated by other factors, including Vps39. Tethered and functionally active vacuole-mitochondria interfaces then compensate for the loss of ERMES-mediated ER-mitochondria contact sites.
Insights
Mitochondrial protein Mcp1 recruits Vps13 to vacuole-mitochondria contacts, bypassing defects in endoplasmic reticulum-mitochondria encounter structure (ERMES) complexes. This pathway compensates for lost ERMES function, maintaining mitochondrial homeostasis.
Area of Science:
- Cell Biology
- Mitochondrial Biology
- Membrane Biology
Background:
- Membrane contact sites (MCS) between the endoplasmic reticulum (ER) and mitochondria, facilitated by the ER-mitochondria encounter structure (ERMES) complex, are vital for cellular functions.
- Disruptions in ERMES can be compensated by specific mutations or protein overexpressions, but the underlying mechanisms are not fully understood.
Purpose of the Study:
- To elucidate the bypass mechanism for ERMES defects involving the endosomal protein Vps13 and the mitochondrial protein Mcp1.
- To define the roles of Mcp1 and Vps13 in maintaining mitochondrial homeostasis when ERMES function is compromised.
Main Methods:
- Investigated the interaction and functional relationship between Mcp1 and Vps13 using cellular and molecular biology techniques.
- Analyzed the localization and recruitment of Vps13 to mitochondria in the presence and absence of functional ERMES.
- Examined the role of Mcp1 in mediating vacuole-mitochondria contacts and compensating for ERMES loss.
Main Results:
- Mitochondrial outer membrane protein Mcp1 actively recruits the endosomal protein Vps13 to mitochondria.
- Mcp1 promotes the association of Vps13 with vacuole-mitochondria contact sites.
- Vps13 and Mcp1 function together as effectors at vacuole-mitochondria contacts, compensating for the absence of ERMES-mediated ER-mitochondria contacts.
Conclusions:
- Mcp1 and Vps13 act as key functional components at vacuole-mitochondria contact sites, independent of ERMES.
- These proteins establish alternative contact sites that maintain mitochondrial homeostasis when ERMES is impaired.
- The findings reveal a novel compensatory pathway for ERMES dysfunction crucial for cell survival and mitochondrial health.
Related Concept Videos
 01:19
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
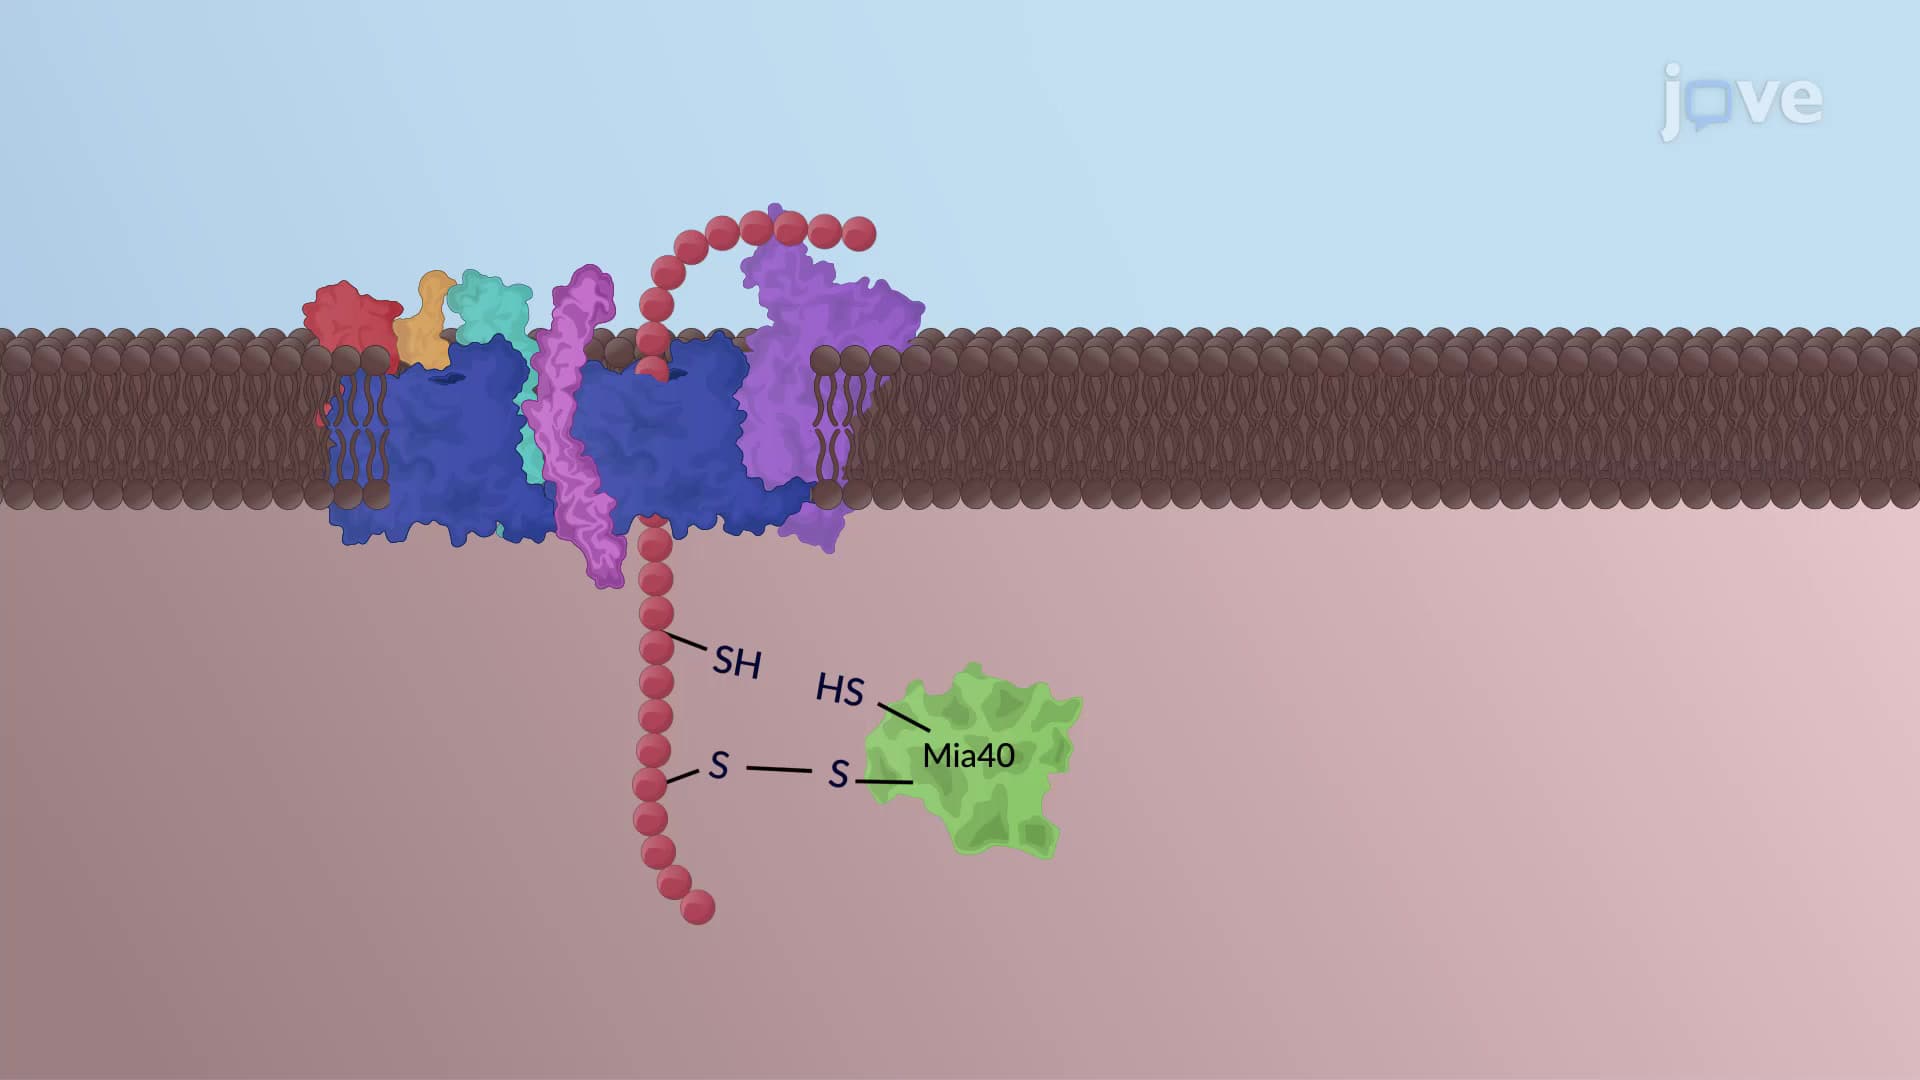
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:38
Intralumenal Vesicles and Multivesicular Bodies
 01:34
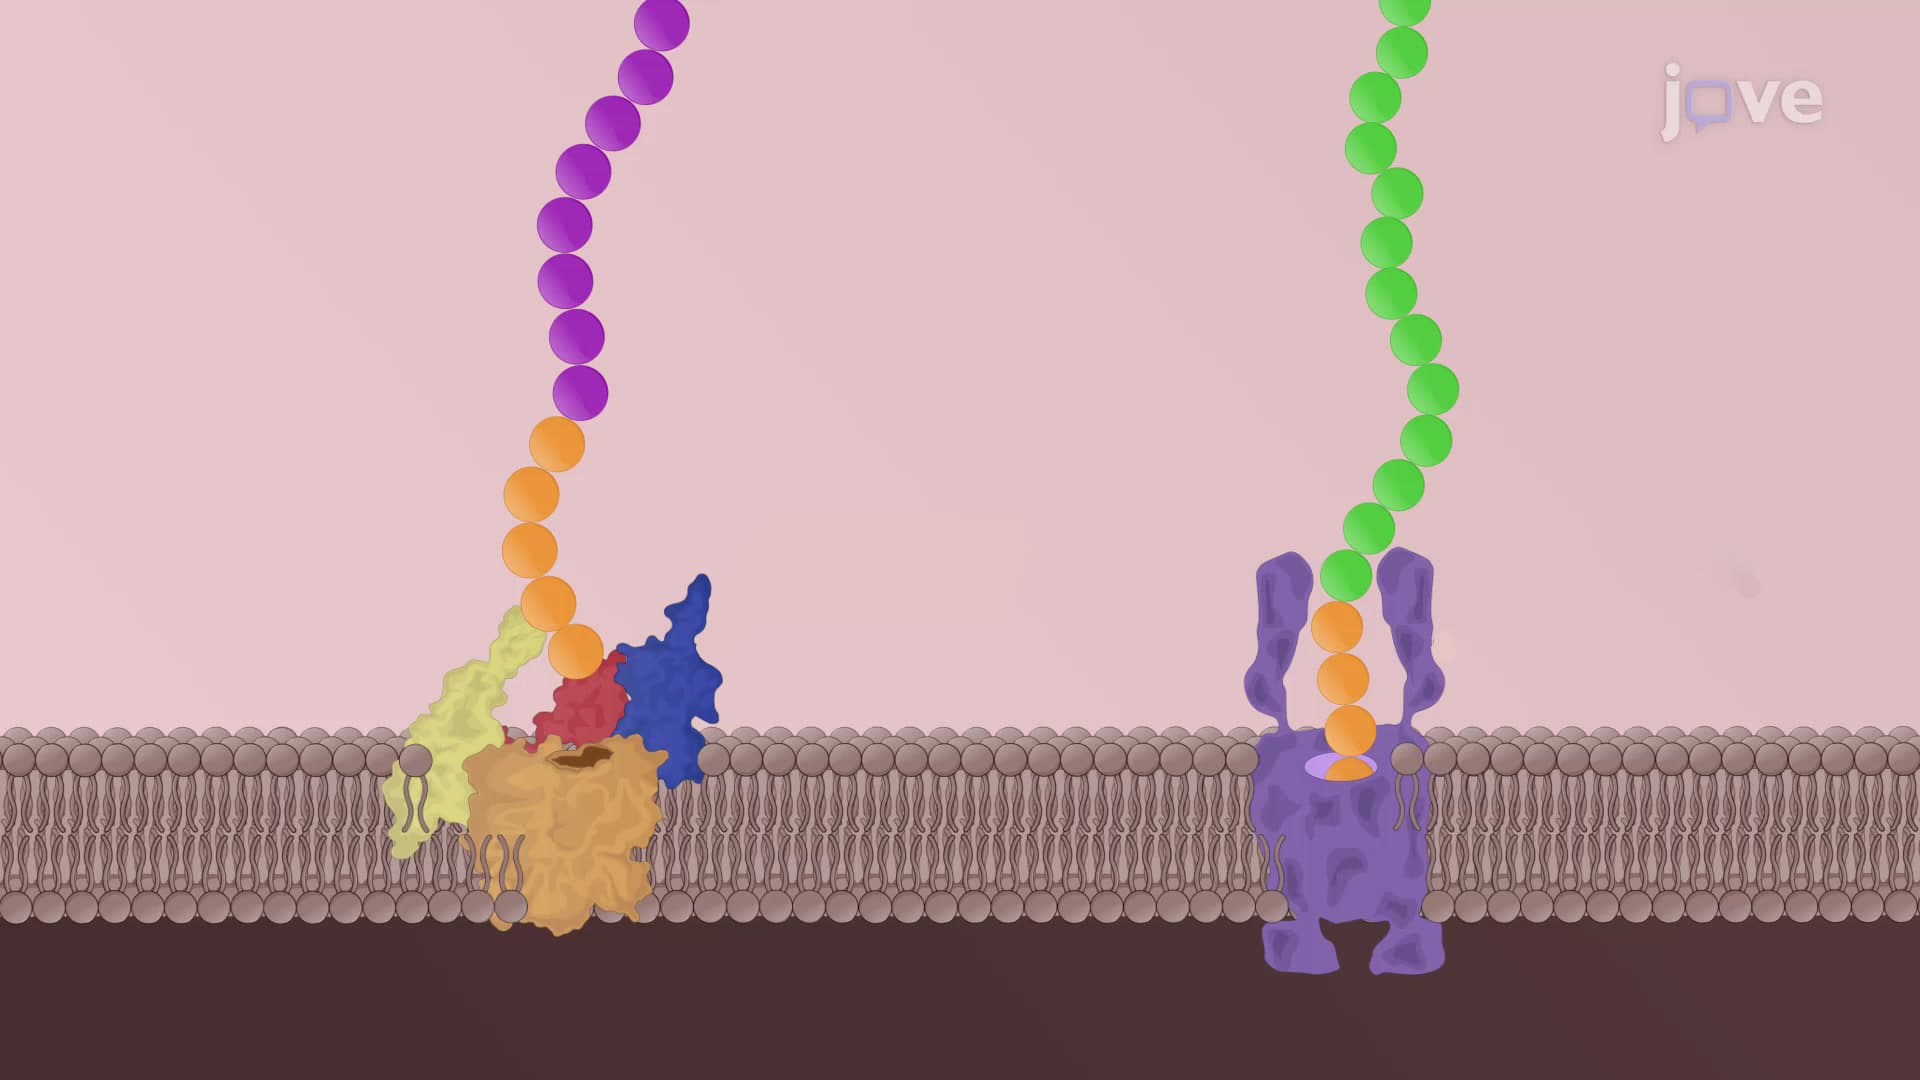
Protein Transport into the Inner Mitochondrial Membrane
Transport of mitochondrial precursors across the TIM23 channel is driven by...
 01:12
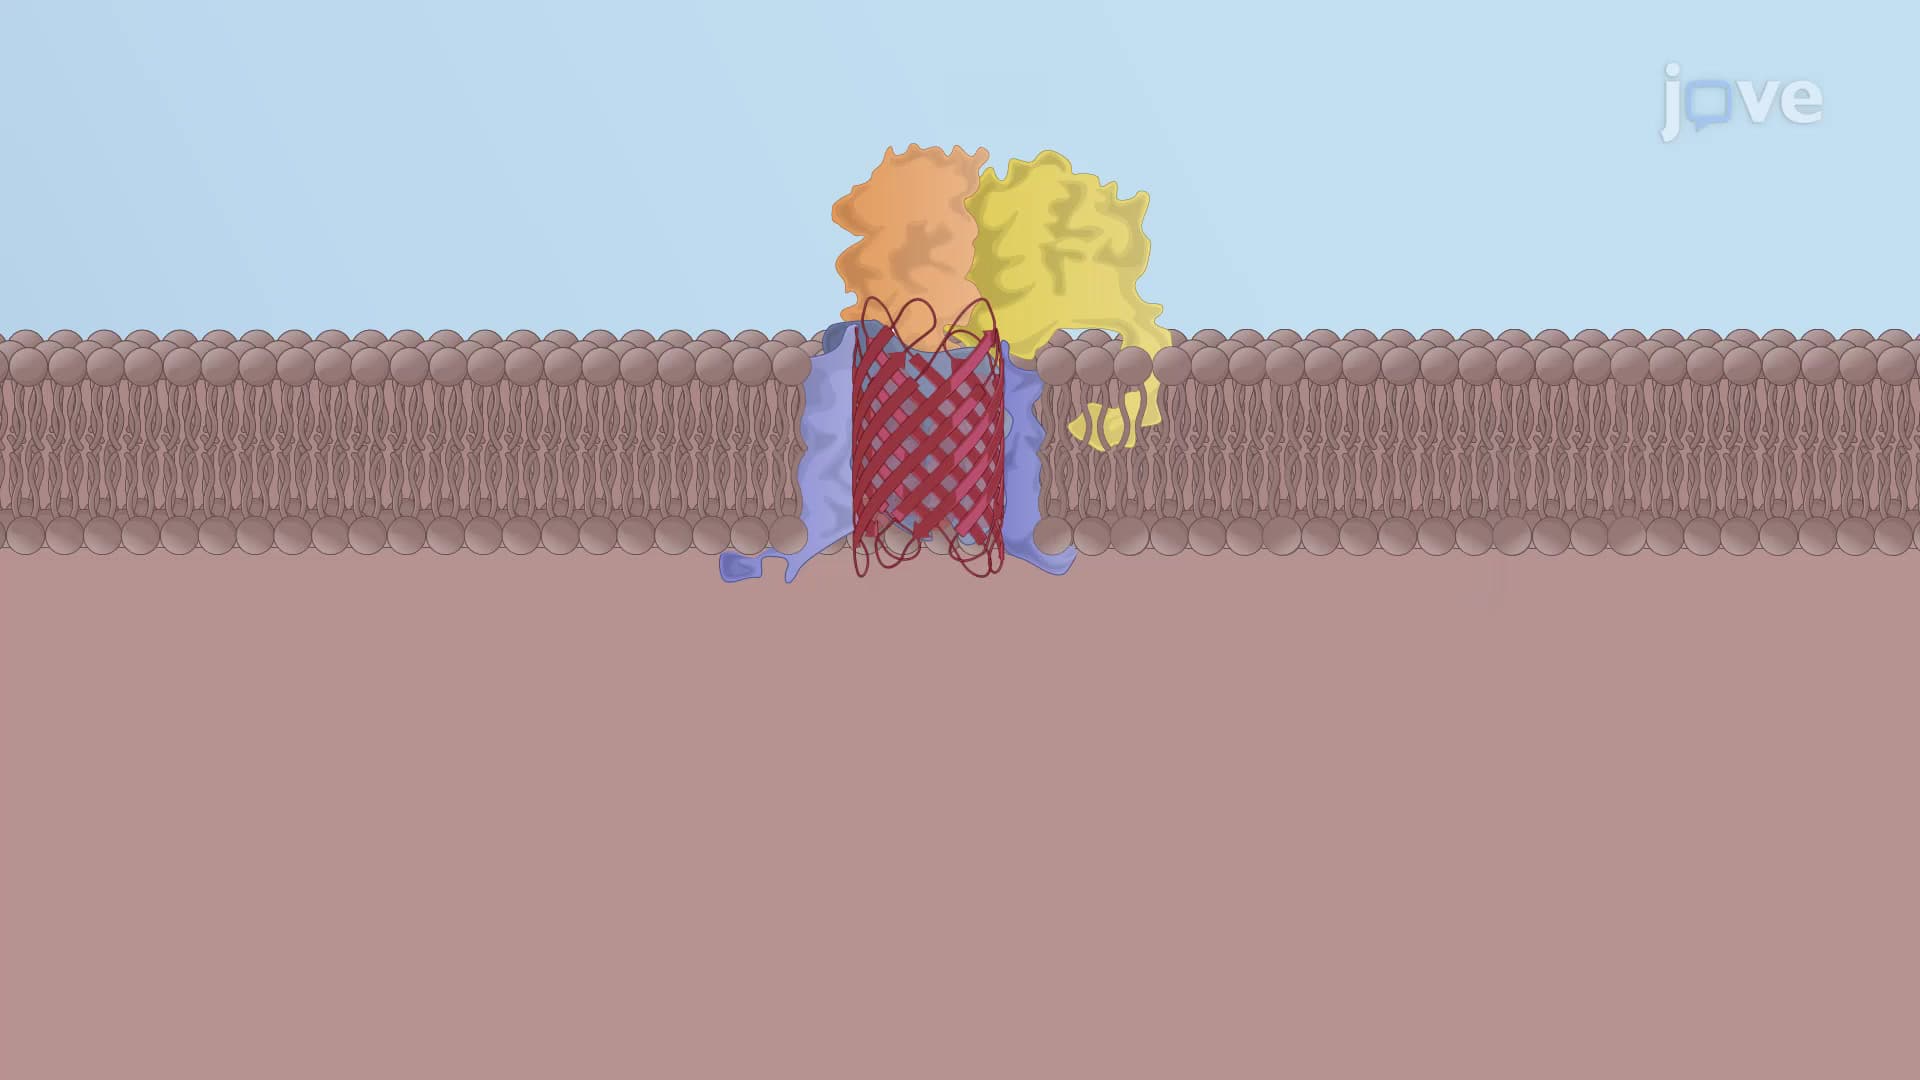
Porin Insertion in the Outer Mitochondrial Membrane
Three models describe the assembly of porins by the SAM complex and their insertion into the outer membrane. Model 1 suggests that porins are assembled outside the SAM channel as the...
 01:39
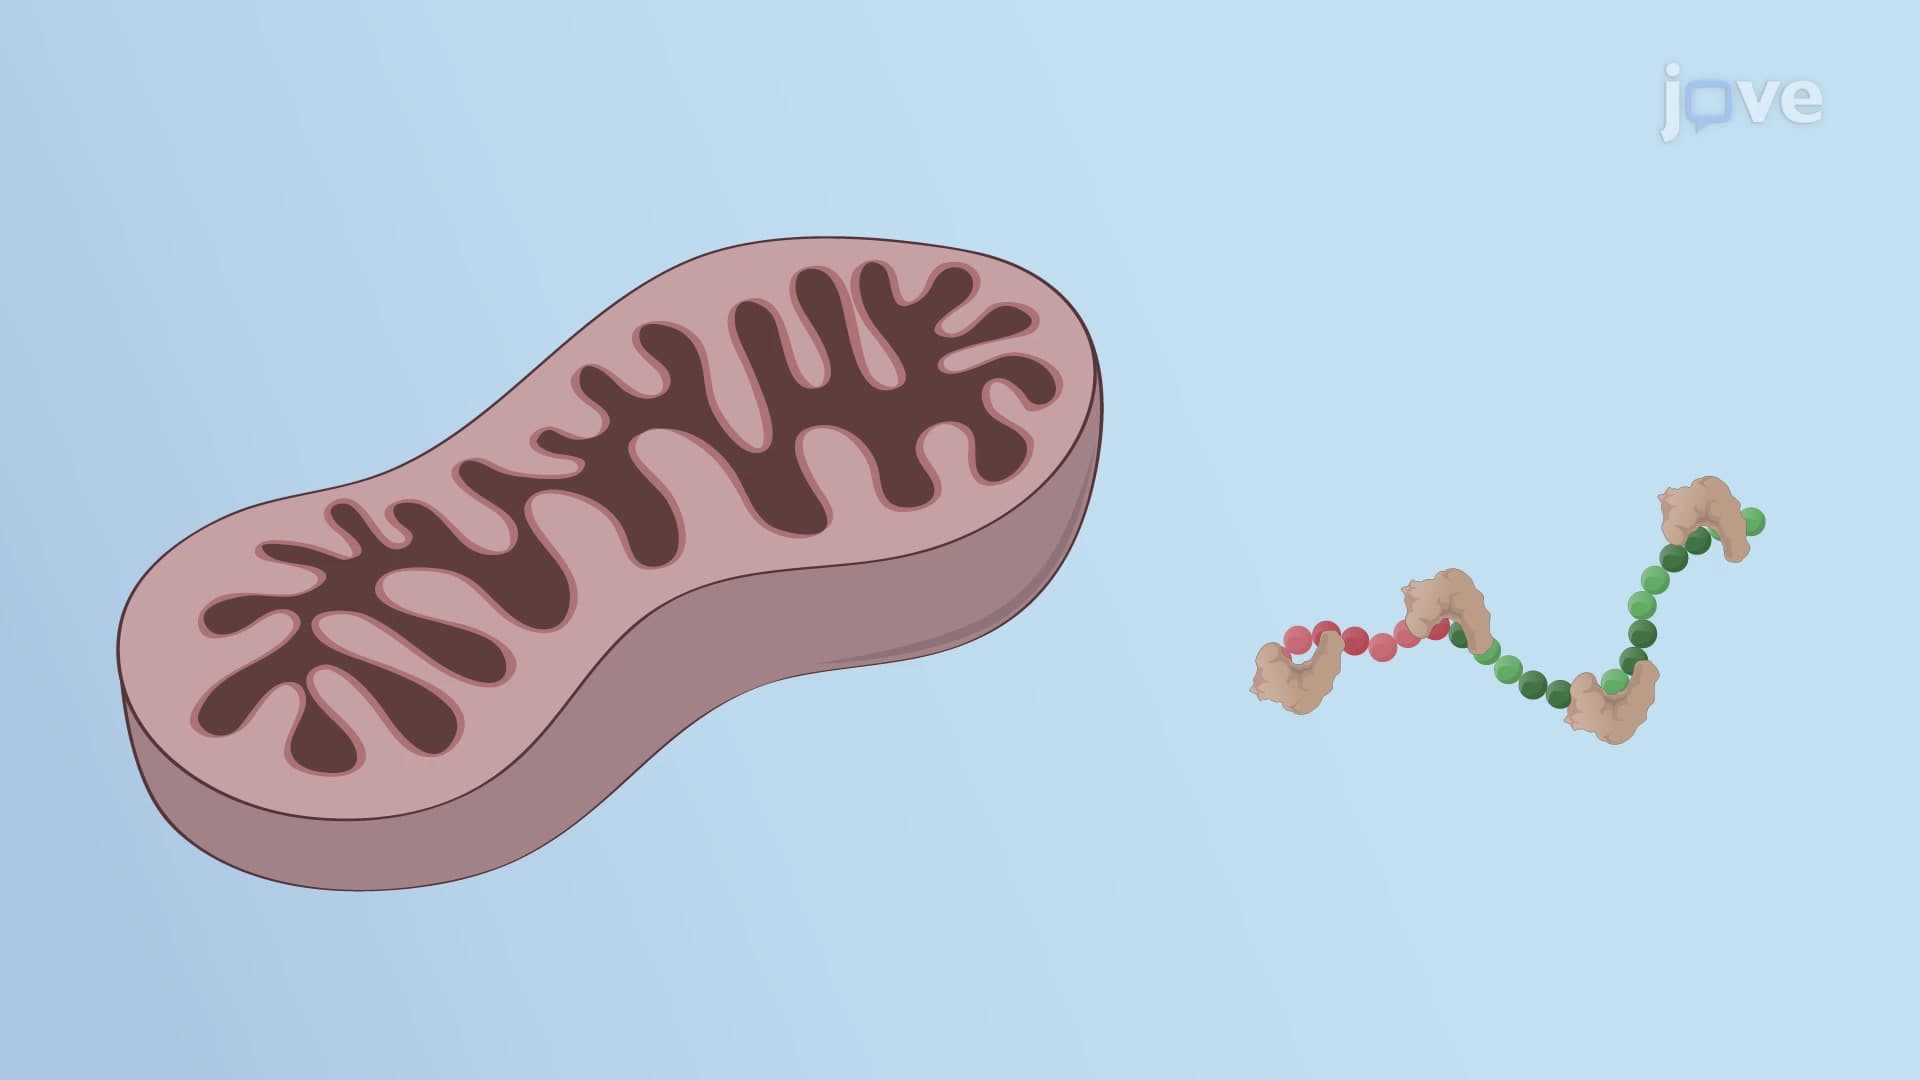
Mitochondrial Protein Sorting
Most of these mitochondrial proteins are encoded by the nucleus and imported to the mitochondria as unfolded or loosely folded precursors. Mitochondrial precursors...
 01:45
Vesicular Tubular Clusters
With the help of motor proteins such...