Related Experiment Video
Updated: Feb 14, 2026

In Vitro Analysis of E3 Ubiquitin Ligase Function
Published on: May 14, 2021
The SKP1-Cullin-F-box E3 ligase βTrCP and CDK2 cooperate to control STIL abundance and centriole number
Christian Arquint1, Fabien Cubizolles1, Agathe Morand1
1Biozentrum, University of Basel, Klingelbergstrasse 50/70, 4056 Basel, Switzerland.

Abstract:
Deregulation of centriole duplication has been implicated in cancer and primary microcephaly. Accordingly, it is important to understand how key centriole duplication factors are regulated. E3 ubiquitin ligases have been implicated in controlling the levels of several duplication factors, including PLK4, STIL and SAS-6, but the precise mechanisms ensuring centriole homeostasis remain to be fully understood. Here, we have combined proteomics approaches with the use of MLN4924, a generic inhibitor of SCF E3 ubiquitin ligases, to monitor changes in the cellular abundance of centriole duplication factors. We identified human STIL as a novel substrate of SCF-βTrCP. The binding of βTrCP depends on a DSG motif within STIL, and serine 395 within this motif is phosphorylated in vivo SCF-βTrCP-mediated degradation of STIL occurs throughout interphase and mutations in the DSG motif causes massive centrosome amplification, attesting to the physiological importance of the pathway. We also uncover a connection between this new pathway and CDK2, whose role in centriole biogenesis remains poorly understood. We show that CDK2 activity protects STIL against SCF-βTrCP-mediated degradation, indicating that CDK2 and SCF-βTrCP cooperate via STIL to control centriole biogenesis.
Insights
Scientists discovered a new pathway regulating centriole duplication by identifying STIL as a target of SCF-βTrCP. This finding is crucial for understanding cell division and diseases like cancer and microcephaly.
Area of Science:
- Cell Biology
- Molecular Biology
- Biochemistry
Background:
- Centriole duplication is essential for cell division and its deregulation is linked to cancer and microcephaly.
- E3 ubiquitin ligases are known to regulate key centriole duplication factors, but precise mechanisms for maintaining centriole homeostasis are unclear.
Purpose of the Study:
- To investigate the regulation of centriole duplication factors.
- To identify novel substrates and mechanisms of SCF E3 ubiquitin ligases in centriole biogenesis.
Main Methods:
- Proteomics approaches were used to identify changes in centriole duplication factors.
- MLN4924, an inhibitor of SCF E3 ubiquitin ligases, was employed to study degradation pathways.
- Investigated the interaction between STIL, SCF-βTrCP, and CDK2.
Main Results:
- Human STIL was identified as a novel substrate of SCF-βTrCP, regulated by a DSG motif phosphorylated in vivo.
- SCF-βTrCP-mediated degradation of STIL occurs during interphase, and mutations in the DSG motif lead to centrosome amplification.
- CDK2 activity was found to protect STIL from SCF-βTrCP-mediated degradation, revealing a cooperative mechanism.
Conclusions:
- A new regulatory pathway involving SCF-βTrCP-mediated degradation of STIL controls centriole duplication.
- This pathway, in cooperation with CDK2, is critical for maintaining centriole homeostasis.
- The findings provide insights into the molecular mechanisms underlying centriole biogenesis and its link to diseases.
Related Concept Videos
 01:58
Cooperative Allosteric Transitions
01:58Cooperative Allosteric Transitions
01:58Cooperative Allosteric Transitions
 02:13
Cooperative Binding of Transcription Regulators
02:13Cooperative Binding of Transcription Regulators
 01:13
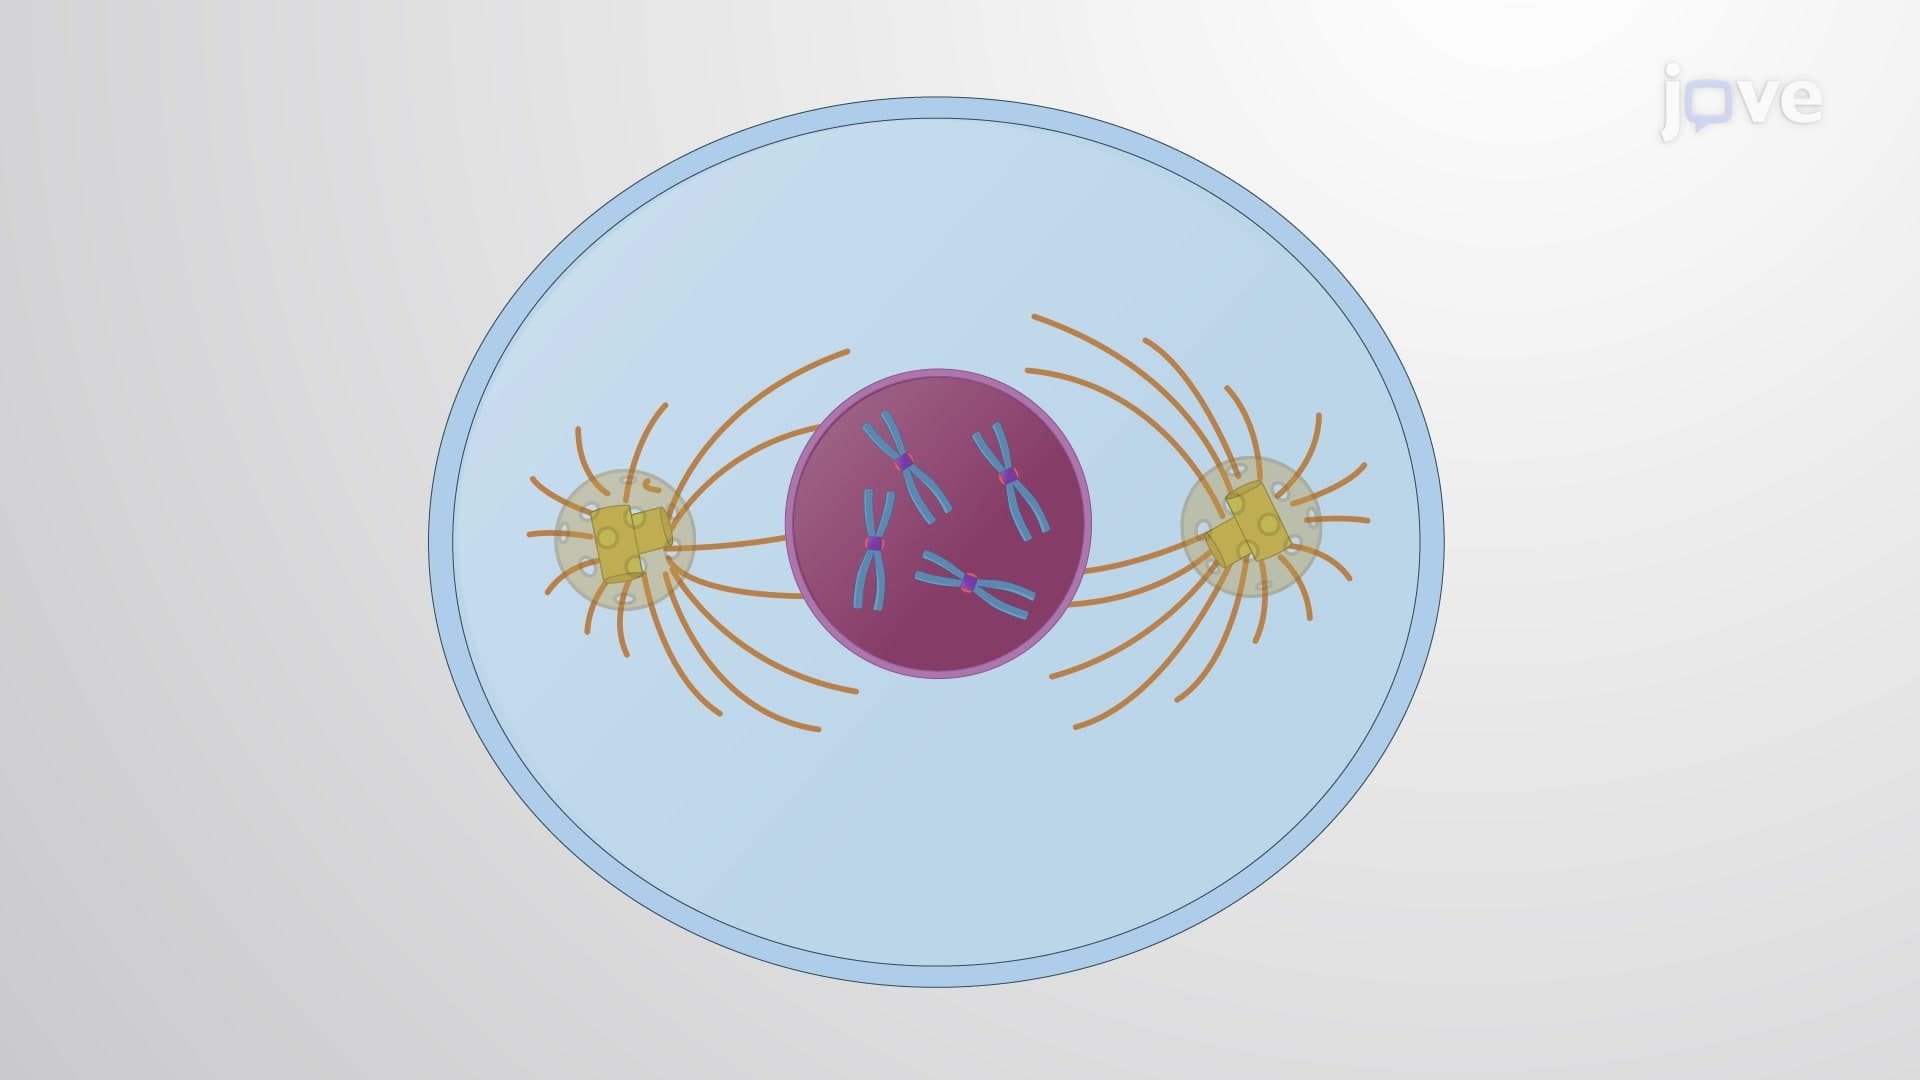
Centrioles and Centrosomes
Near the end of the prophase, also called late prophase or...