Related Experiment Video
Updated: Oct 23, 2026
A Protein Preparation Method for the High-throughput Identification of Proteins Interacting with a Nuclear Cofactor Using LC-MS/MS Analysis
Published on: January 24, 2017
On the relationship status for Arf and NPM1 - it's complicated
Diana M Mitrea1, Richard W Kriwacki1,2
1Department of Structural Biology, St. Jude Children's Research Hospital, Memphis, TN, USA.

Abstract:
Arf levels are tightly regulated in cells and correlate with the level of ribosome biogenesis and proliferative status of cells. Through multivalent interactions with NPM1 - a regulator of ribosome biogenesis, and Mdm2 - a regulator of cellular fate, Arf integrates within the nucleolar matrix, altering its structure, dynamics and function and therefore modulates the cell cycle.
Insights
Cellular levels of Arf protein are linked to ribosome production and cell growth. Arf interacts with NPM1 and Mdm2 within the nucleolus, changing its structure and function to control the cell cycle.
Area of Science:
- Cell Biology
- Molecular Biology
- Cancer Research
Background:
- Arf protein levels are critical indicators of cellular ribosome biogenesis and proliferation.
- The nucleolus is a key site for ribosome synthesis and plays a role in cell cycle regulation.
- NPM1 and Mdm2 are crucial regulators involved in ribosome biogenesis and cellular fate, respectively.
Purpose of the Study:
- To investigate the role of Arf in integrating ribosome biogenesis and cell cycle control.
- To elucidate the mechanism by which Arf interacts with NPM1 and Mdm2 within the nucleolus.
- To understand how Arf modulates nucleolar structure, dynamics, and function.
Main Methods:
- Analysis of Arf protein levels in correlation with ribosome biogenesis markers.
- Investigating the multivalent interactions of Arf with NPM1 and Mdm2 using biochemical assays.
- Studying the structural and dynamic changes within the nucleolar matrix upon Arf integration.
Main Results:
- Arf levels directly correlate with ribosome biogenesis and cellular proliferative status.
- Arf forms multivalent interactions with NPM1 and Mdm2, integrating into the nucleolar matrix.
- This integration alters the nucleolar matrix's structure, dynamics, and function.
Conclusions:
- Arf acts as a central integrator of ribosome biogenesis and cell cycle control.
- Arf's interaction with NPM1 and Mdm2 in the nucleolus is essential for modulating cell cycle progression.
- Understanding Arf's role in nucleolar function provides insights into cellular growth regulation and potential therapeutic targets.
Related Concept Videos
 01:14
Generation of Straight or Branched Actin Filaments
Arp2/3 Complex
Arp2/3 complex is a seven-subunit complex consisting of two proteins similar to actin- Arp2 and Arp3, and five other subunits that help keep Arp2 and Arp3 inactive. When required, the complex is...
 01:13
¹H NMR: Complex Splitting
Splitting diagrams or splitting tree diagrams are routinely used to depict such complex couplings. While drawing splitting diagrams, the splitting with the larger coupling constant is usually applied first.
 01:30
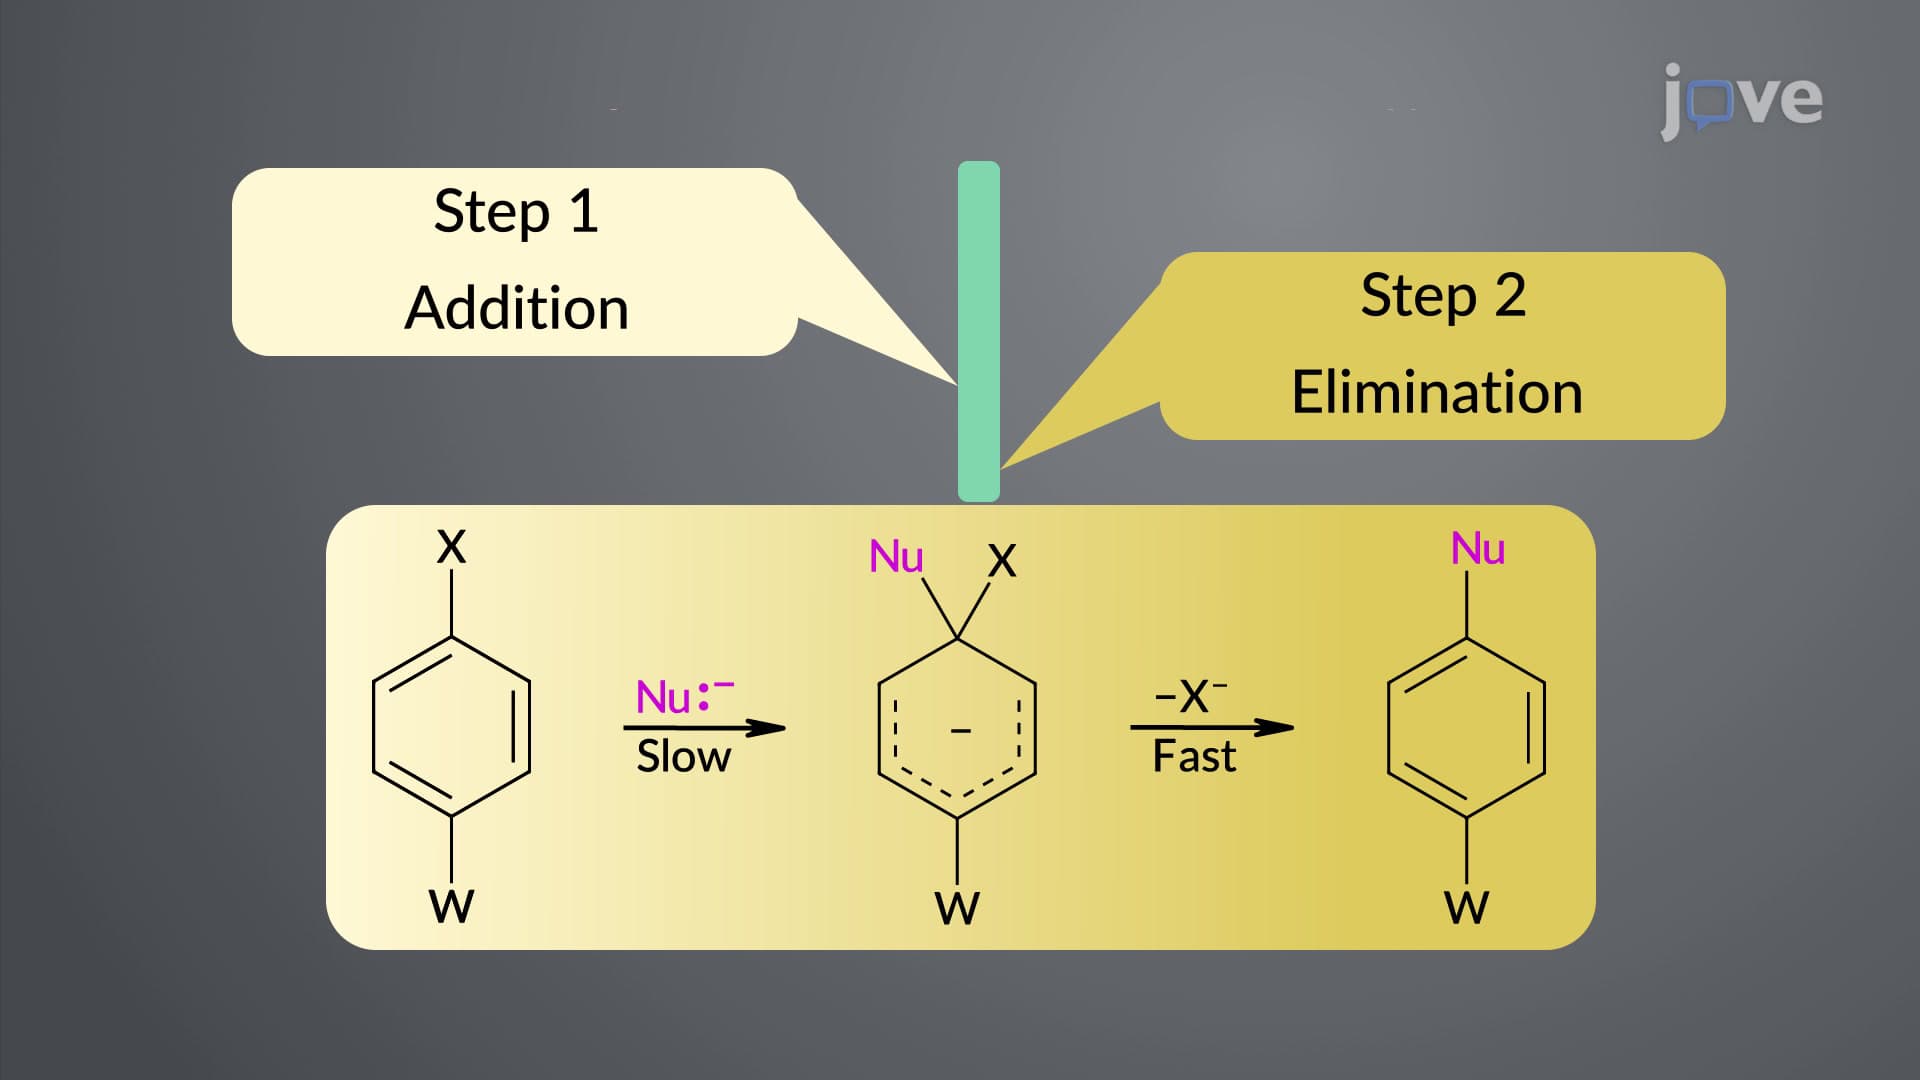
Nucleophilic Aromatic Substitution: Addition–Elimination (SNAr)
The reaction begins with an attack of the nucleophile on the carbon that holds the leaving group. This results in the delocalization of the π electrons over the ring carbons. The resonance interaction between the...
 01:13
¹H NMR Signal Multiplicity: Splitting Patterns
 01:10
Interpreting ¹H NMR Signal Splitting: The (n + 1) Rule
 01:09
¹H NMR: Pople Notation
A proton...