Related Experiment Video
Updated: Feb 3, 2026

Genotyping Single Nucleotide Polymorphisms in the Mitochondrial Genome by Pyrosequencing
Published on: February 10, 2023
The mitochondrial inner membrane protein MPV17 prevents uracil accumulation in mitochondrial DNA
Judith R Alonzo1, Chantel Venkataraman2, Martha S Field2
1From the Graduate Field of Biochemistry, Molecular, and Cellular Biology and.

Abstract:
Mitochondrial inner membrane protein MPV17 is a protein of unknown function that is associated with mitochondrial DNA (mtDNA)-depletion syndrome (MDS). MPV17 loss-of-function has been reported to result in tissue-specific nucleotide pool imbalances, which can occur in states of perturbed folate-mediated one-carbon metabolism (FOCM), but MPV17 has not been directly linked to FOCM. FOCM is a metabolic network that provides one-carbon units for the de novo synthesis of purine and thymidylate nucleotides (e.g. dTMP) for both nuclear DNA (nuDNA) and mtDNA replication. In this study, we investigated the impact of reduced MPV17 expression on markers of impaired FOCM in HeLa cells. Depressed MPV17 expression reduced mitochondrial folate levels by 43% and increased uracil levels, a marker of impaired dTMP synthesis, in mtDNA by 3-fold. The capacity of mitochondrial de novo and salvage pathway dTMP biosynthesis was unchanged by the reduced MPV17 expression, but the elevated levels of uracil in mtDNA suggested that other sources of mitochondrial dTMP are compromised in MPV17-deficient cells. These results indicate that MPV17 provides a third dTMP source, potentially by serving as a transporter that transfers dTMP from the cytosol to mitochondria to sustain mtDNA synthesis. We propose that MPV17 loss-of-function and related hepatocerebral MDS are linked to impaired FOCM in mitochondria by providing insufficient access to cytosolic dTMP pools and by severely reducing mitochondrial folate pools.
Insights
Mitochondrial protein MPV17 deficiency impairs folate metabolism and thymidylate synthesis, crucial for mitochondrial DNA replication. This suggests MPV17 is vital for transferring thymidylate precursors to mitochondria, impacting mitochondrial DNA-depletion syndrome.
Area of Science:
- Biochemistry
- Molecular Biology
- Cell Biology
Background:
- Mitochondrial inner membrane protein MPV17 is linked to mitochondrial DNA (mtDNA)-depletion syndrome (MDS).
- MPV17 loss-of-function causes nucleotide pool imbalances, potentially involving folate-mediated one-carbon metabolism (FOCM).
- FOCM provides essential one-carbon units for nucleotide synthesis required for nuclear and mtDNA replication.
Purpose of the Study:
- To investigate the impact of reduced MPV17 expression on markers of impaired FOCM in HeLa cells.
- To determine if MPV17 deficiency affects mitochondrial folate levels and thymidylate synthesis.
Main Methods:
- Reduced MPV17 expression in HeLa cells.
- Quantification of mitochondrial folate levels.
- Measurement of uracil and thymidylate levels in mtDNA.
- Assessment of mitochondrial de novo and salvage pathway dTMP biosynthesis capacity.
Main Results:
- Reduced MPV17 expression decreased mitochondrial folate by 43%.
- Uracil levels in mtDNA increased 3-fold, indicating impaired thymidylate synthesis.
- Mitochondrial de novo and salvage dTMP biosynthesis capacity remained unchanged.
- Elevated uracil suggests compromised mitochondrial dTMP sources in MPV17-deficient cells.
Conclusions:
- MPV17 may act as a transporter for cytosolic thymidylate precursors to mitochondria, supporting mtDNA synthesis.
- MPV17 loss-of-function in hepatocerebral MDS could stem from impaired mitochondrial FOCM due to reduced cytosolic thymidylate access and depleted mitochondrial folate pools.
Related Concept Videos
 01:34
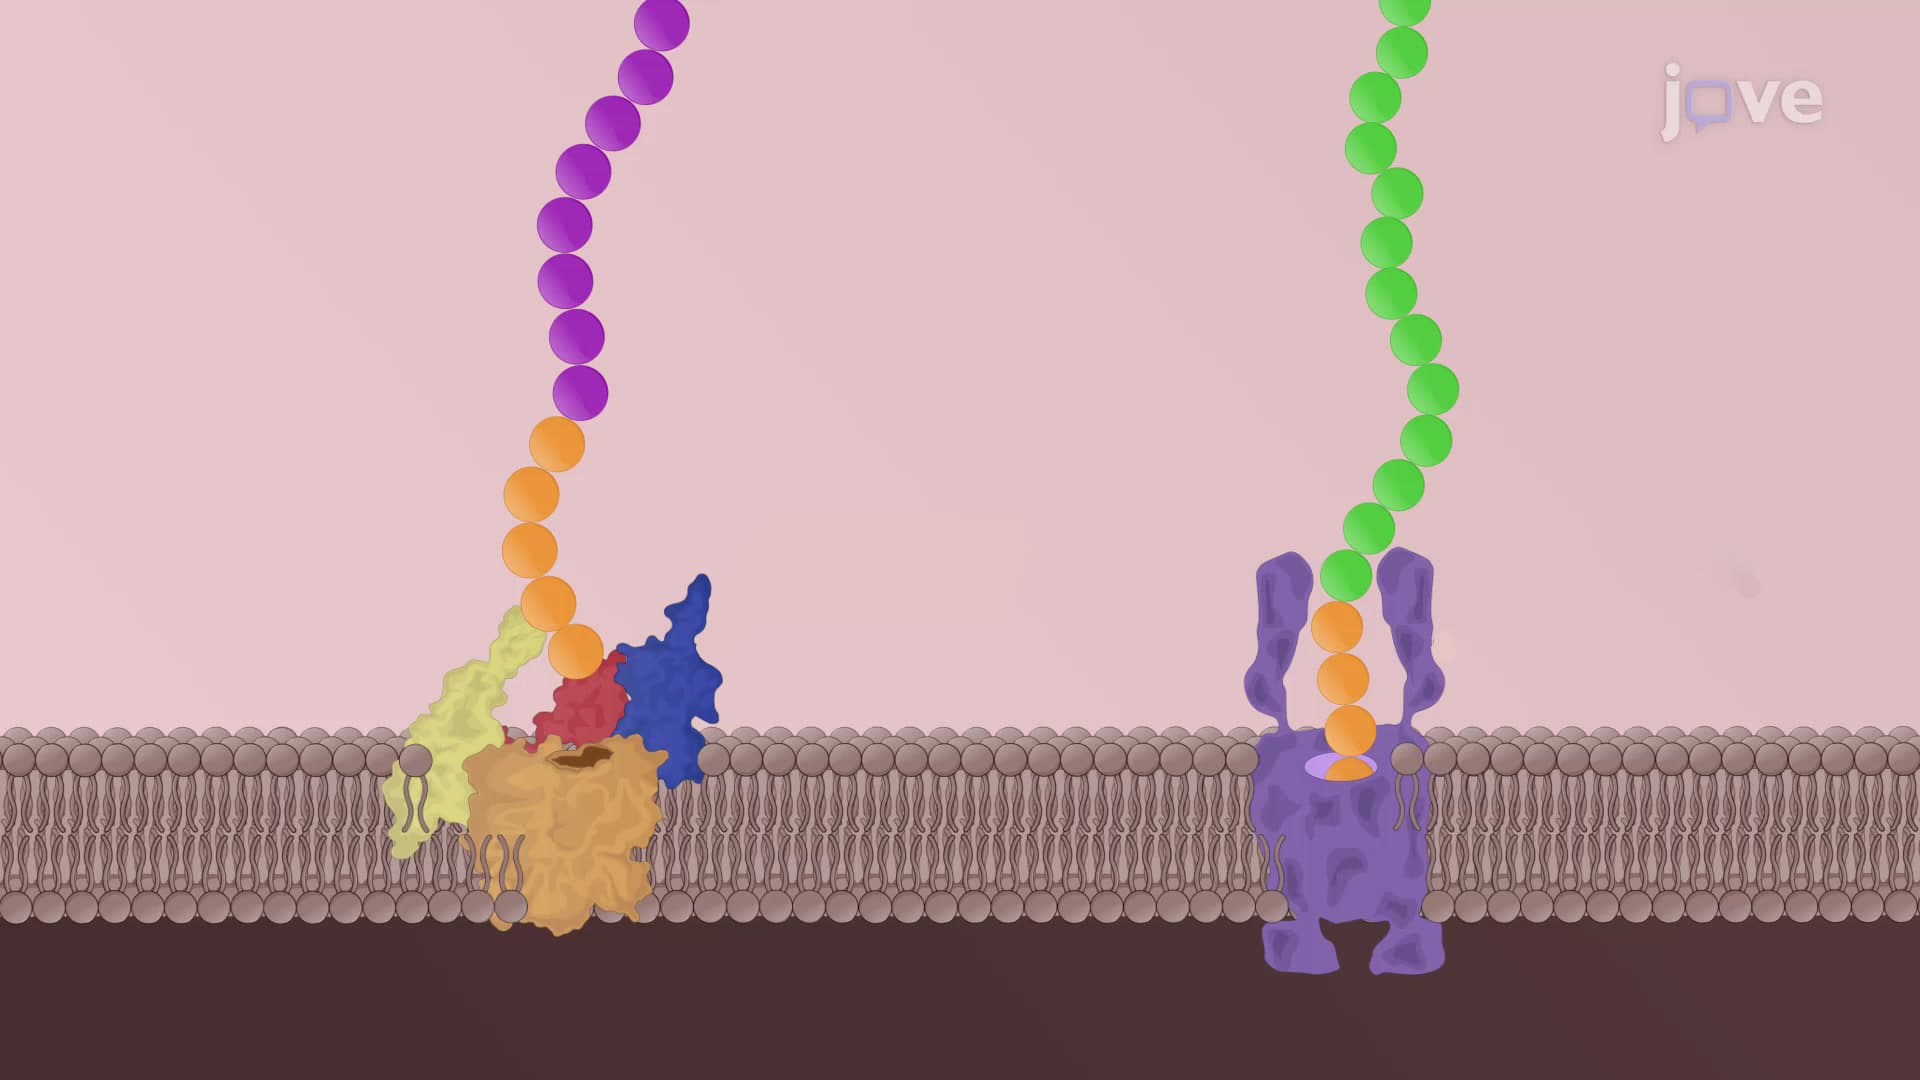
Protein Transport into the Inner Mitochondrial Membrane
Transport of mitochondrial precursors across the TIM23 channel is driven by...
 02:59
Animal Mitochondrial Genetics
 01:28
The Inner Mitochondrial Membrane
 02:19
Export of Mitochondrial and Chloroplast Genes
 01:45
Mitochondrial Membranes
 02:16
Comparing Mitochondrial, Chloroplast, and Prokaryotic Genomes