Related Experiment Video
Updated: Feb 1, 2026
Assessment of the Cytotoxic and Immunomodulatory Effects of Substances in Human Precision-cut Lung Slices
Published on: May 9, 2018
Enhancing tetrandrine cytotoxicity in human lung carcinoma A549 cells by suppressing mitochondrial ATP production
Louis W C Chow1,2,3, Ka-Shun Cheng4, Fai Leong5
1State Key Laboratory of Quality Research in Chinese Medicines, Macau University of Science and Technology, Macau, China.

Abstract:
ATP depletion induced by inhibiting glycolysis or mitochondrial ATP production has been demonstrated to cause cancer cell death. Whether ATP depletion can enhance the efficacy and potency of anti-cancer effects of herbal compounds is so far unknown. We examined the enhancing effect of ATP depletion on anti-cancer actions of tetrandrine (TET) in human lung carcinoma A549 cells. A 24-h incubation of A549 cells with tetrandrine caused a concentration-dependent cytotoxic effect (LC50 = 66.1 μM). Co-incubation with 20 mM 2-deoxyglucose (2-DG, glycolysis inhibitor) caused only a very slight enhancement of tetrandrine cytotoxicity. By contrast, inhibiting mitochondrial ATP production with oligomycin (10 μM, ATP synthase inhibitor) and FCCP (30 μM, uncoupling agent) (thus, oligo-FCCP) on its own caused only slight cell cytotoxicity but strongly potentiated tetrandrine cytotoxicity (tetrandrine LC50 = 15.6 μM). The stronger enhancing effect of oligo-FCCP than 2-DG on TET toxicity did not result from more severe overall ATP depletion, since both treatments caused a similar ATP level suppression. Neither oligo-FCCP nor 2-DG synergized with tetrandrine in decreasing mitochondrial membrane potential. TET on its own triggered reactive oxygen species (ROS) production, and oligo-FCCP, but not 2-DG, potentiated TET in causing ROS production. Taken together, our results suggest that inhibiting ATP production from mitochondria, but not from glycolysis, appears to be a very effective means in augmenting TET-triggered ROS production and hence toxicity in A549 cells.
Insights
Inhibiting mitochondrial ATP production, but not glycolysis, significantly enhances the anti-cancer effects of tetrandrine (TET) in lung cancer cells. This approach boosts TET-induced reactive oxygen species (ROS) production and cell death.
Area of Science:
- Biochemistry
- Cell Biology
- Pharmacology
Background:
- ATP depletion is a known inducer of cancer cell death.
- The potential of ATP depletion to enhance the efficacy of herbal anti-cancer compounds remains unexplored.
Purpose of the Study:
- To investigate whether inhibiting ATP production can enhance the anti-cancer effects of tetrandrine (TET).
- To compare the effects of inhibiting glycolysis versus mitochondrial ATP production on TET's anti-cancer activity.
Main Methods:
- Human lung carcinoma A549 cells were treated with tetrandrine (TET).
- Cells were co-treated with glycolysis inhibitor 2-deoxyglucose (2-DG) or mitochondrial inhibitors oligomycin and FCCP (oligo-FCCP).
- Cytotoxicity, ATP levels, mitochondrial membrane potential, and reactive oxygen species (ROS) production were assessed.
Main Results:
- Tetrandrine (TET) exhibited concentration-dependent cytotoxicity against A549 cells.
- Inhibiting mitochondrial ATP production with oligo-FCCP significantly potentiated TET's cytotoxicity more than inhibiting glycolysis with 2-DG.
- Both treatments similarly reduced overall ATP levels but only oligo-FCCP enhanced TET-induced ROS production.
Conclusions:
- Mitochondrial ATP production inhibition is a more effective strategy than glycolysis inhibition for potentiating TET's anti-cancer effects in lung cancer cells.
- Enhanced ROS production by mitochondria appears to be the key mechanism underlying the potentiation of TET toxicity.
Related Concept Videos
 01:31
ATP Yield
The ETC is embedded in the inner mitochondrial membrane and is comprised of four main protein complexes and an ATP synthase. NADH and FADH2 pass electrons to these complexes, which pump protons into the intermembrane space. This distribution of...
 01:23
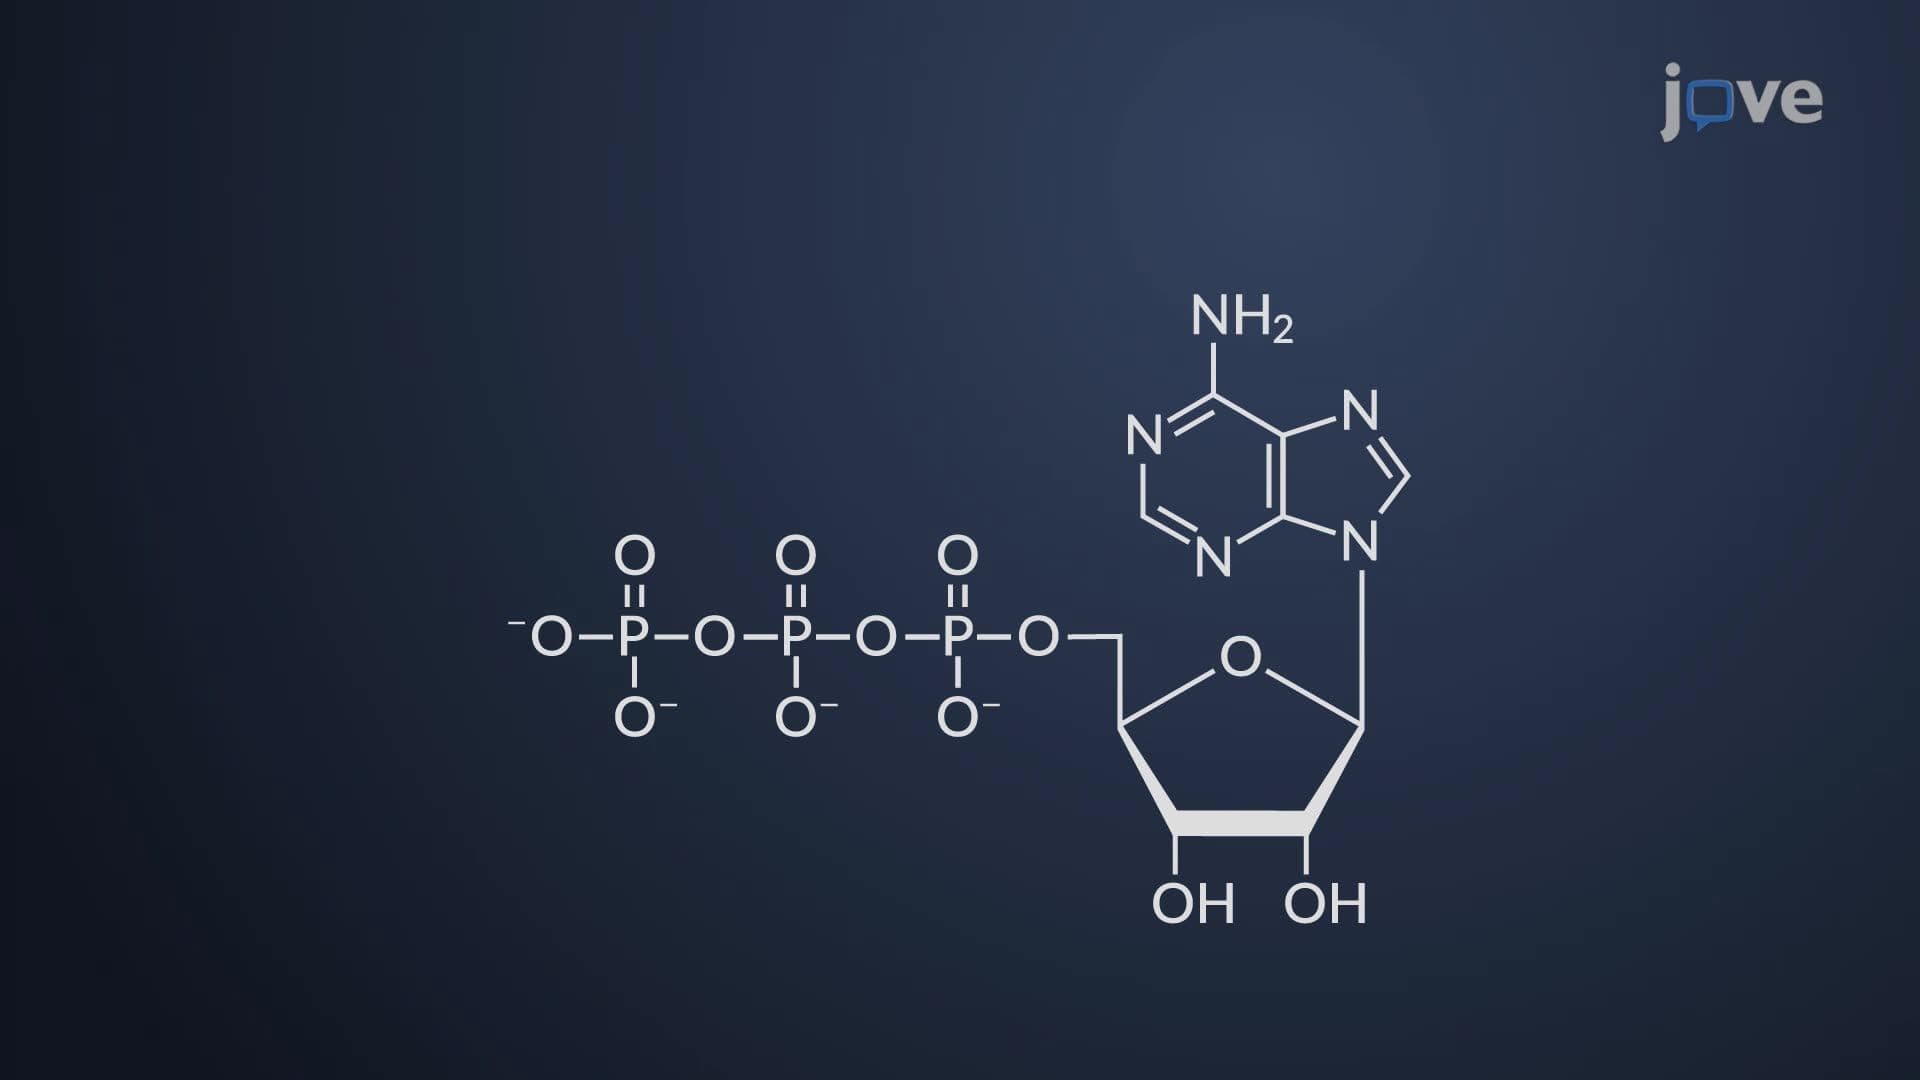
ATP and Energy Production
 02:59
Animal Mitochondrial Genetics
 01:08
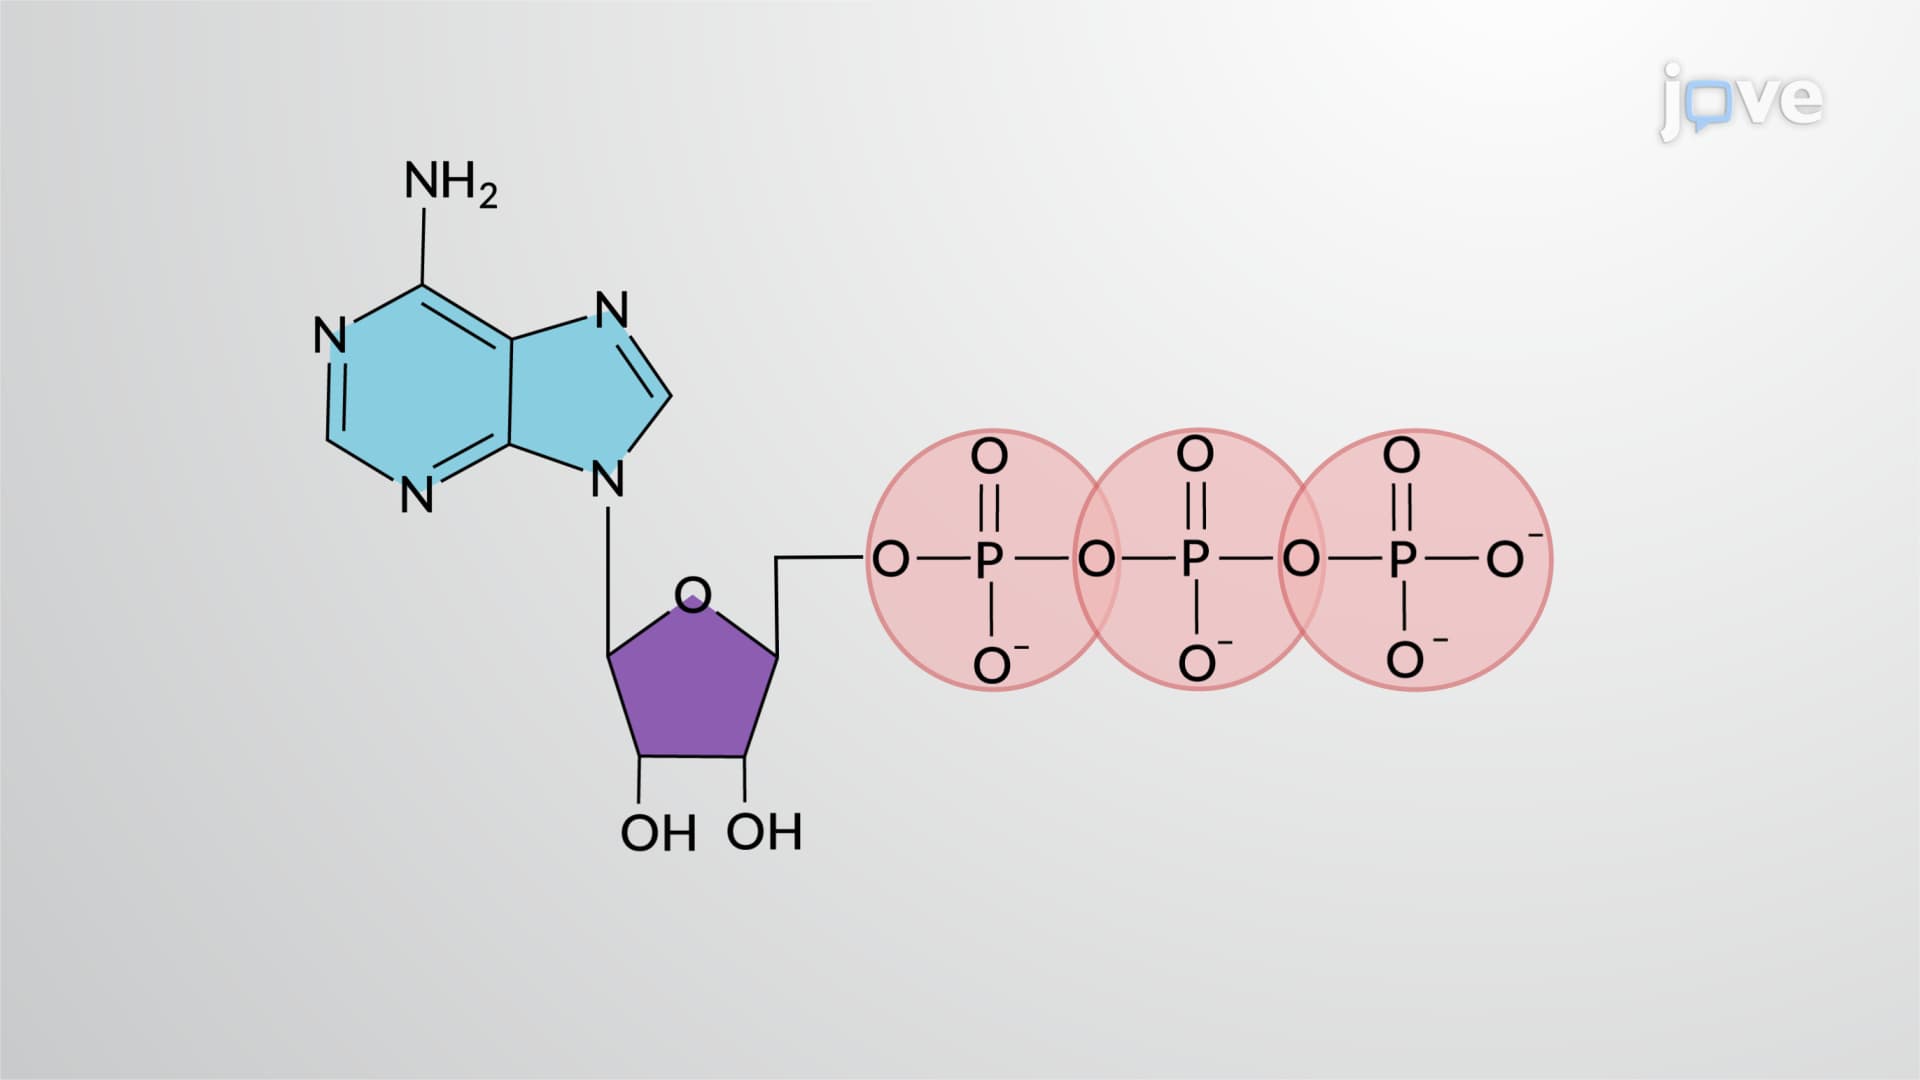
Hydrolysis of ATP
If one phosphate group is removed, a molecule of ADP—adenosine diphosphate—remains, along with inorganic phosphate. ADP can be further hydrolyzed to AMP—adenosine...
 02:16
Comparing Mitochondrial, Chloroplast, and Prokaryotic Genomes
 02:19
Export of Mitochondrial and Chloroplast Genes