Related Experiment Video
Updated: Jan 26, 2026
An Optimized Rhizobox Protocol to Visualize Root Growth and Responsiveness to Localized Nutrients
Published on: October 22, 2018
Phytoplankton growth and stoichiometric responses to warming, nutrient addition and grazing depend on lake
Marika A Schulhof1,2, Jonathan B Shurin1, Steven A J Declerck2
1Division of Biological Sciences, Section of Ecology, Behavior & Evolution, University of California San Diego, La Jolla, California.

Abstract:
Global change involves shifts in multiple environmental factors that act in concert to shape ecological systems in ways that depend on local biotic and abiotic conditions. Little is known about the effects of combined global change stressors on phytoplankton communities, and particularly how these are mediated by distinct community properties such as productivity, grazing pressure and size distribution. Here, we tested for the effects of warming and eutrophication on phytoplankton net growth rate and C:N:P stoichiometry in two phytoplankton cell size fractions (<30 µm and >30 µm) in the presence and absence of grazing in microcosm experiments. Because effects may also depend on lake productivity, we used phytoplankton communities from three Dutch lakes spanning a trophic gradient. We measured the response of each community to multifactorial combinations of temperature, nutrient, and grazing treatments and found that nutrients elevated net growth rates and reduced carbon:nutrient ratios of all three phytoplankton communities. Warming effects on growth and stoichiometry depended on nutrient supply and lake productivity, with enhanced growth in the most productive community dominated by cyanobacteria, and strongest stoichiometric responses in the most oligotrophic community at ambient nutrient levels. Grazing effects were also most evident in the most oligotrophic community, with reduced net growth rates and phytoplankton C:P stoichiometry that suggests consumer-driven nutrient recycling. Our experiments indicate that stoichiometric responses to warming and interactions with nutrient addition and grazing are not universal but depend on lake productivity and cell size distribution.
More Related Videos
 08:15
Author Spotlight: Unveiling Plankton Response to Climate Change Through Time-Series Data and Artistic Expression
Published on: July 28, 2023
 09:13
Hydroponics: A Versatile System to Study Nutrient Allocation and Plant Responses to Nutrient Availability and Exposure to Toxic Elements
Published on: July 13, 2016
Related Concept Videos
 01:22
Cell Size
Surface Area
Cells can take in nutrients and water via diffusion through the plasma membrane itself or through specific channels in the membrane. The area of the membrane surrounding...
 02:36
Meristems and Plant Growth
 01:27
Conjugate Addition (1,4-Addition) vs Direct Addition (1,2-Addition)
Conjugate addition results in a thermodynamically stable product. The reaction retains the stronger C=O bond at the expense of the weaker C=C π bond. The process is slow as the β carbon is less electrophilic than the carbonyl carbon.
Direct addition products are...
 02:10
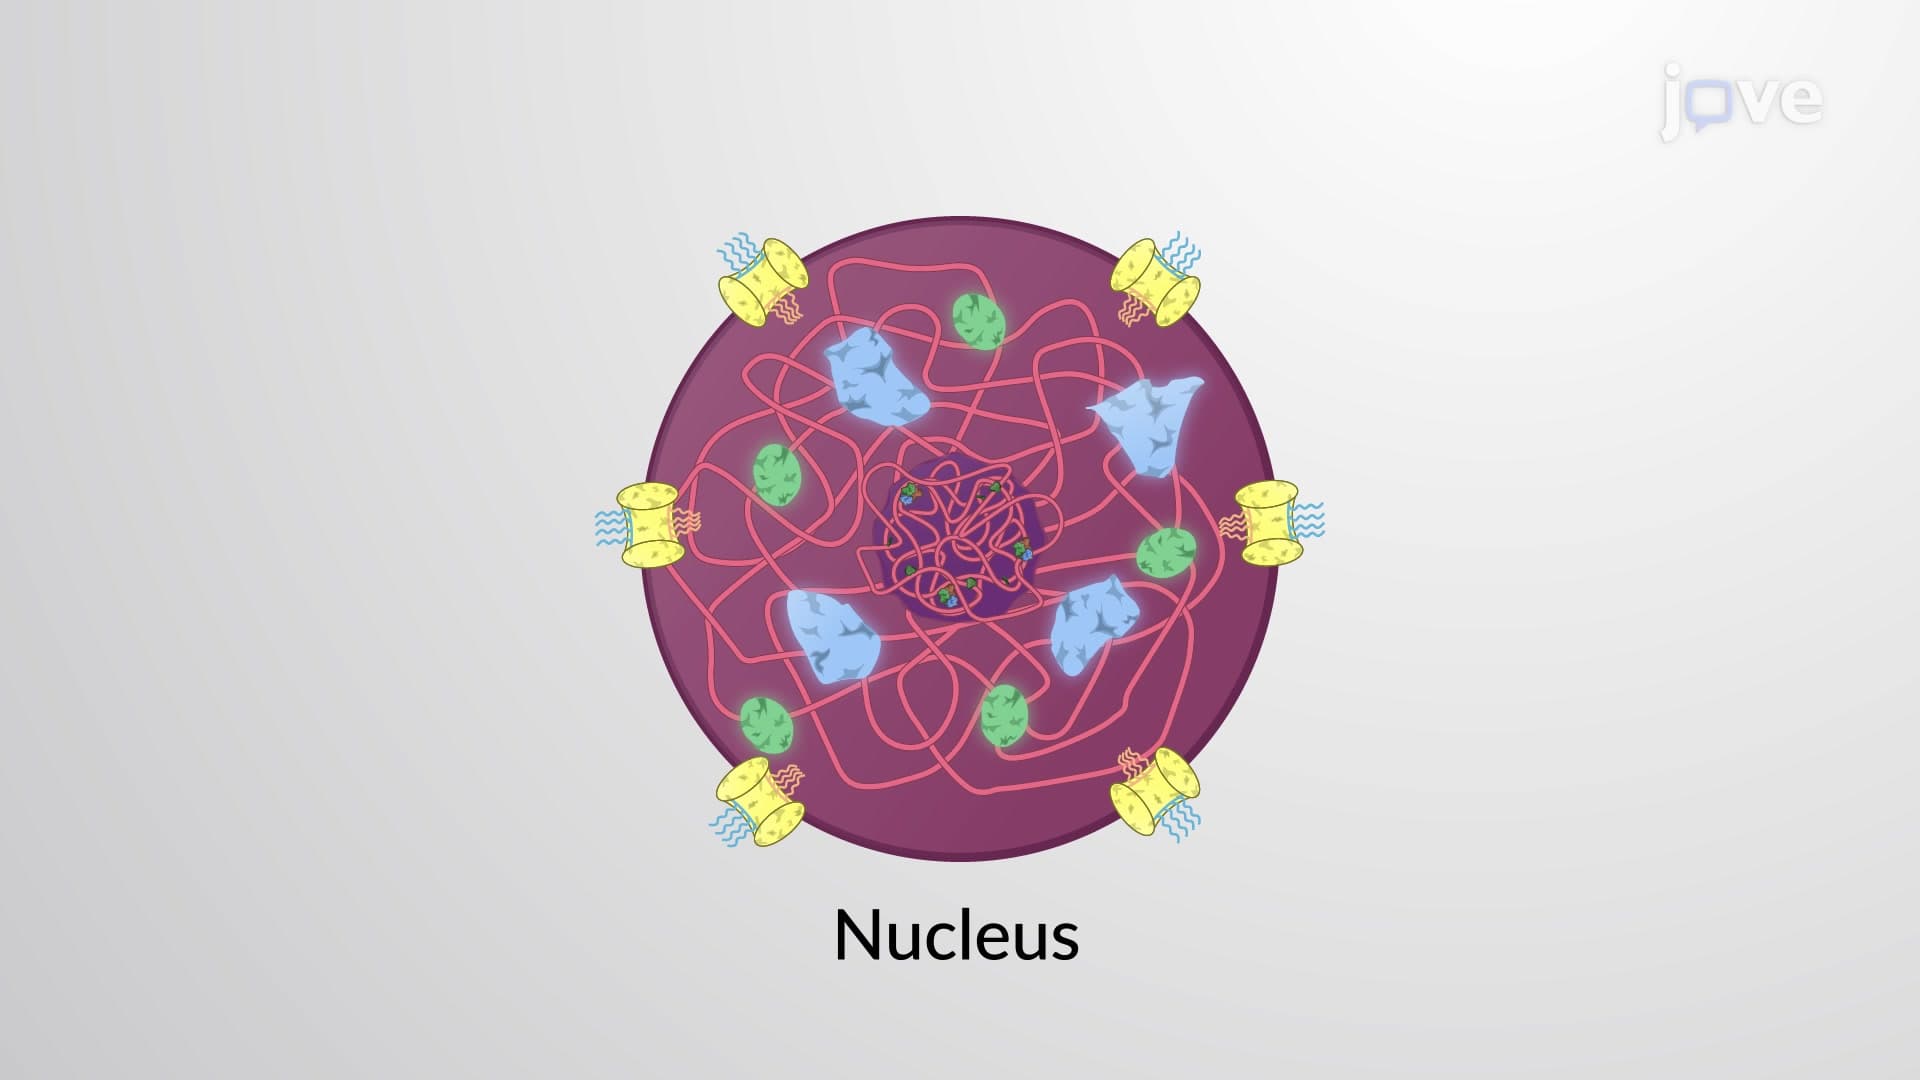
Additional Subnuclear Structures
The nucleus contains many membrane-less subnuclear organelles or nuclear bodies, such as nucleoli, Cajal bodies, speckles,...
 01:19
Absorption of Nutrients
Enterocytes, which are specialized polar epithelial cells, line the mucosa of the small intestinal walls. These cells...
 01:08
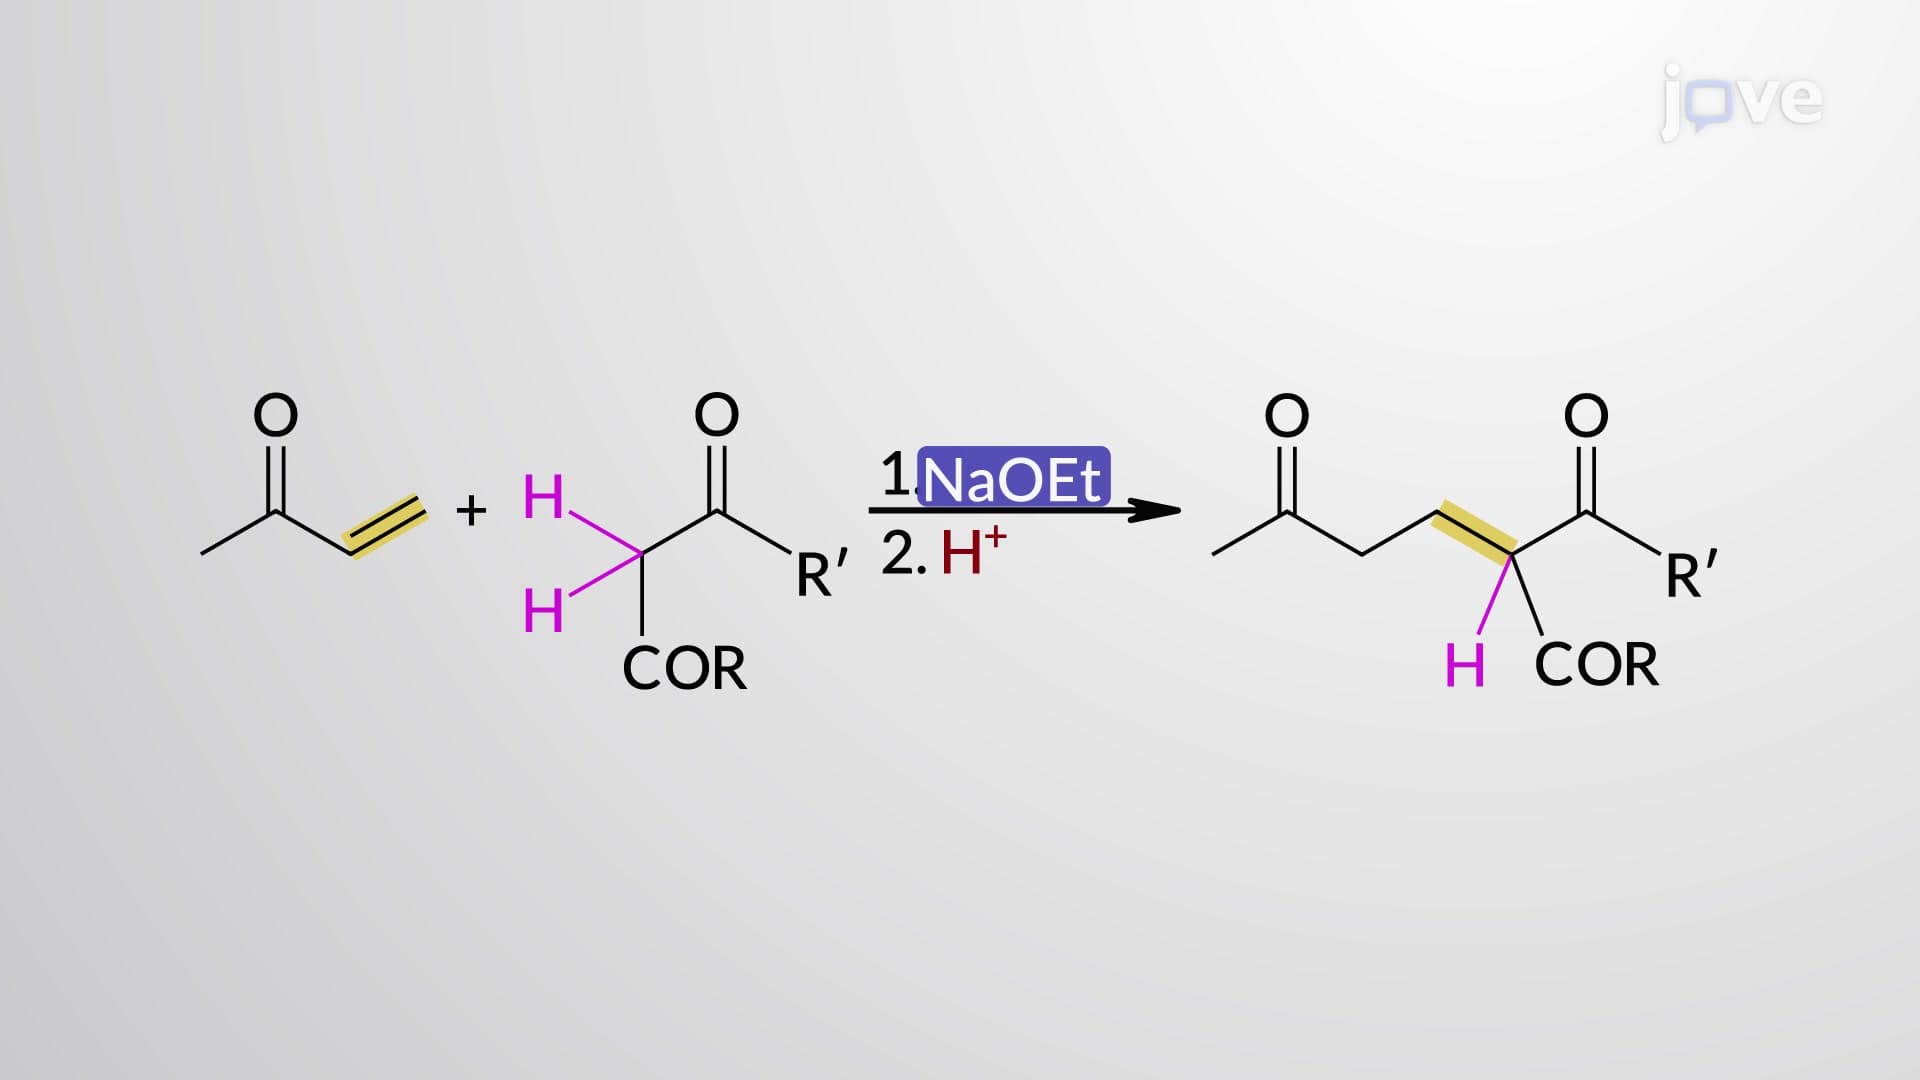
Conjugate Addition of Enolates: Michael Addition