Related Experiment Video
Updated: Jan 6, 2026
In Vitro Analysis of E3 Ubiquitin Ligase Function
Published on: May 14, 2021
A tri-ionic anchor mechanism drives Ube2N-specific recruitment and K63-chain ubiquitination in TRIM ligases
Leo Kiss1, Jingwei Zeng1, Claire F Dickson1,2
1Medical Research Council Laboratory of Molecular Biology, Cambridge, UK.

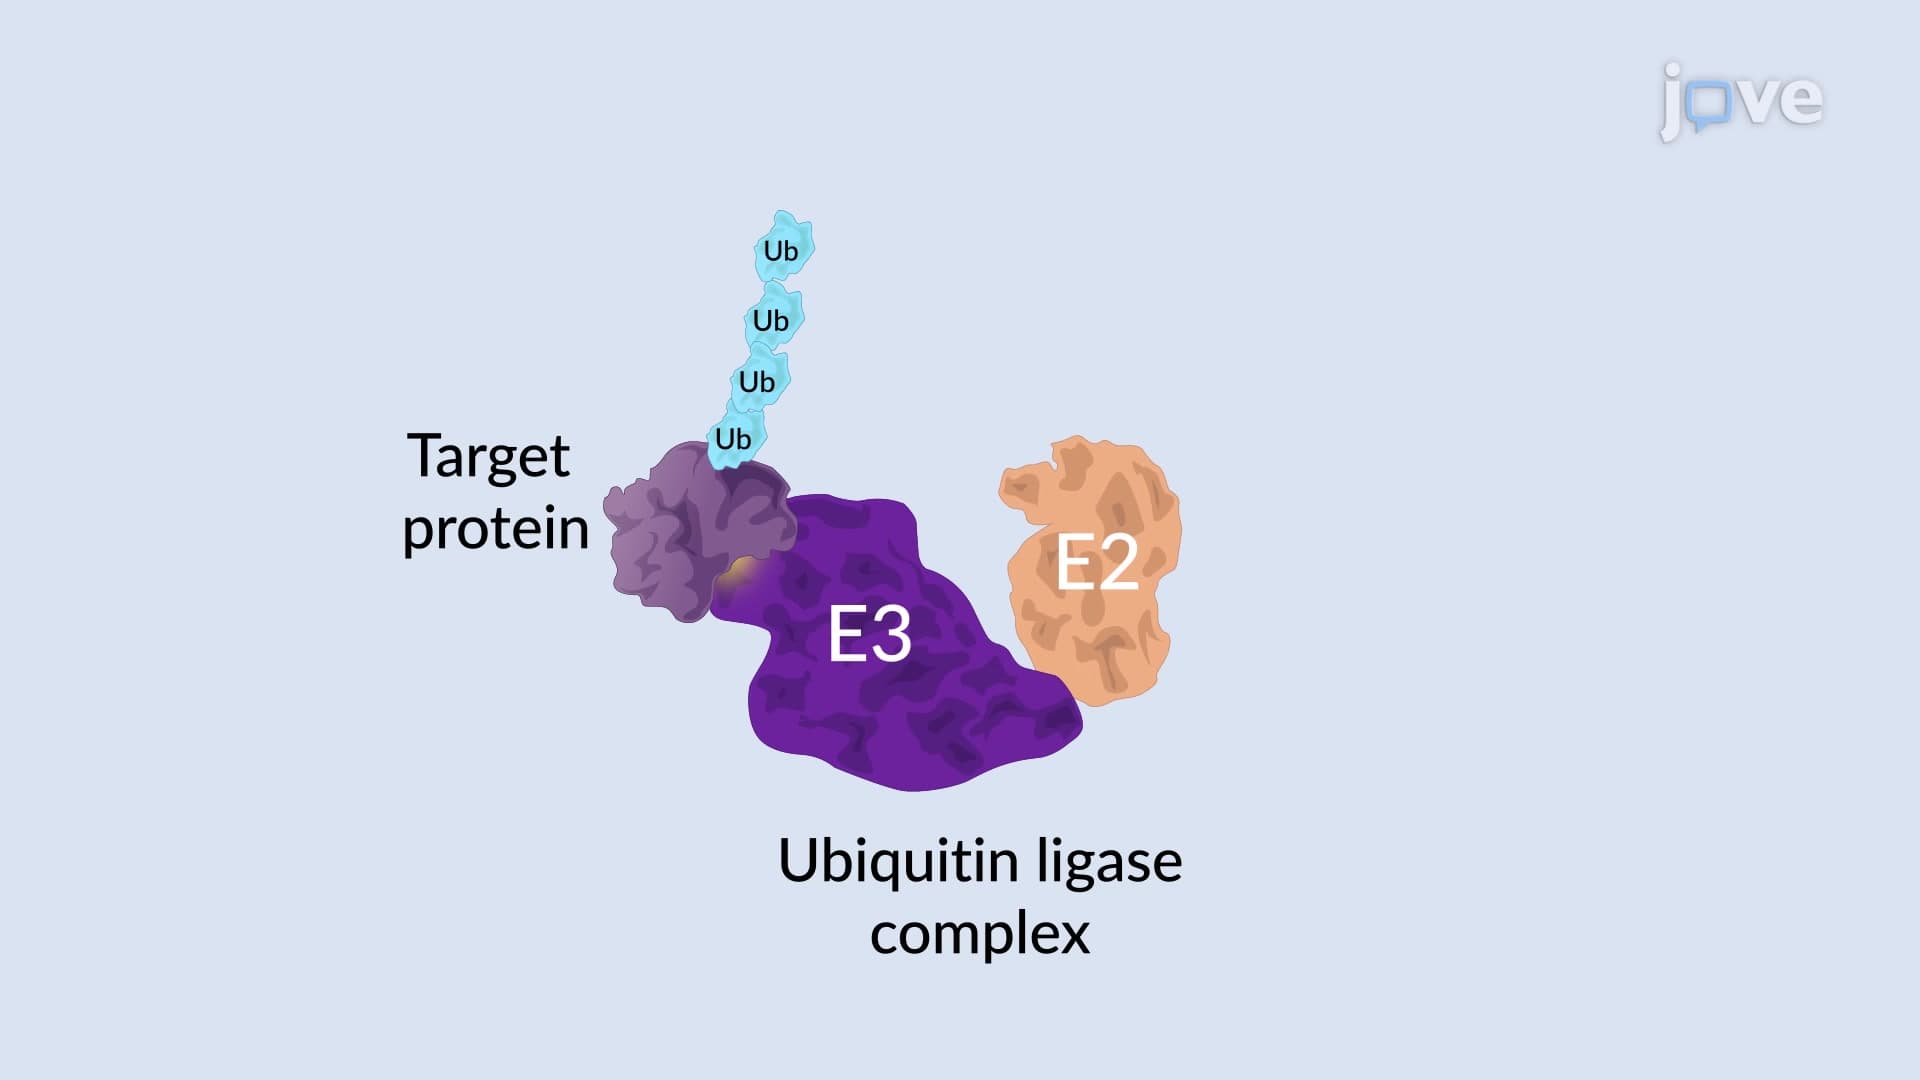
The cytosolic antibody receptor TRIM21 possesses unique ubiquitination activity that drives broad-spectrum anti-pathogen targeting and underpins the protein depletion technology Trim-Away. This activity is dependent on formation of self-anchored, K63-linked ubiquitin chains by the heterodimeric E2 enzyme Ube2N/Ube2V2. Here we reveal how TRIM21 facilitates ubiquitin transfer and differentiates this E2 from other closely related enzymes. A tri-ionic motif provides optimally distributed anchor points that allow TRIM21 to wrap an Ube2N~Ub complex around its RING domain, locking the closed conformation and promoting ubiquitin discharge. Mutation of these anchor points inhibits ubiquitination with Ube2N/Ube2V2, viral neutralization and immune signalling. We show that the same mechanism is employed by the anti-HIV restriction factor TRIM5 and identify spatially conserved ionic anchor points in other Ube2N-recruiting RING E3s. The tri-ionic motif is exclusively required for Ube2N but not Ube2D1 activity and provides a generic E2-specific catalysis mechanism for RING E3s.
The cytosolic antibody receptor TRIM21 possesses unique ubiquitination activity that drives broad-spectrum anti-pathogen targeting and underpins the protein depletion technology Trim-Away. This activity is dependent on formation of self-anchored, K63-linked ubiquitin chains by the heterodimeric E2 enzyme Ube2N/Ube2V2. Here we reveal how TRIM21 facilitates ubiquitin transfer and differentiates this E2 from other closely related enzymes. A tri-ionic motif provides optimally distributed anchor points that allow TRIM21 to wrap an Ube2N~Ub complex around its RING domain, locking the closed conformation and promoting ubiquitin discharge. Mutation of these anchor points inhibits ubiquitination with Ube2N/Ube2V2, viral neutralization and immune signalling. We show that the same mechanism is employed by the anti-HIV restriction factor TRIM5 and identify spatially conserved ionic anchor points in other Ube2N-recruiting RING E3s. The tri-ionic motif is exclusively required for Ube2N but not Ube2D1 activity and provides a generic E2-specific catalysis mechanism for RING E3s.
Related Concept Videos
 02:04
Covalently Linked Protein Regulators
These groups modify specific amino acids in a protein....
 02:58
Regulated Protein Degradation
Protein degradation plays two important roles in the cells. It helps to protect cells from misfolded or damaged proteins before they lead to a...
 01:32
Lipids as Anchors
The carboxy-terminal of most of the prenylated proteins, such as Ras proteins, contains...
 01:57
Protein Complexes with Interchangeable Parts
The SCF ubiquitin ligase is a protein complex of five individual proteins. This complex attaches ubiquitin to other target proteins to mark them for degradation. In order...
 01:45
Tail-anchoring of Proteins in the ER Membrane
 01:38
Intralumenal Vesicles and Multivesicular Bodies