Related Experiment Video
Updated: Dec 25, 2025

Single-Molecule FRET Imaging for Observing the Conformational Dynamics of Dynamin-Like GTPase Atlastin
Published on: January 24, 2025
Transmembrane protein rotaxanes reveal kinetic traps in the refolding of translocated substrates
Jianfei Feng1, Pablo Martin-Baniandres1, Michael J Booth1
1Department of Chemistry, University of Oxford, 12 Mansfield Road, Oxford, OX1 3TA, UK.

Abstract:
Understanding protein folding under conditions similar to those found in vivo remains challenging. Folding occurs mainly vectorially as a polypeptide emerges from the ribosome or from a membrane translocon. Protein folding during membrane translocation is particularly difficult to study. Here, we describe a single-molecule method to characterize the folded state of individual proteins after membrane translocation, by monitoring the ionic current passing through the pore. We tag both N and C termini of a model protein, thioredoxin, with biotinylated oligonucleotides. Under an electric potential, one of the oligonucleotides is pulled through a α-hemolysin nanopore driving the unfolding and translocation of the protein. We trap the protein in the nanopore as a rotaxane-like complex using streptavidin stoppers. The protein is subjected to cycles of unfolding-translocation-refolding switching the voltage polarity. We find that the refolding pathway after translocation is slower than in bulk solution due to the existence of kinetic traps.
Related Concept Videos
 01:37
Energy to Drive Translocation
Generally, polypeptides are unfolded by two distinct...
 01:19
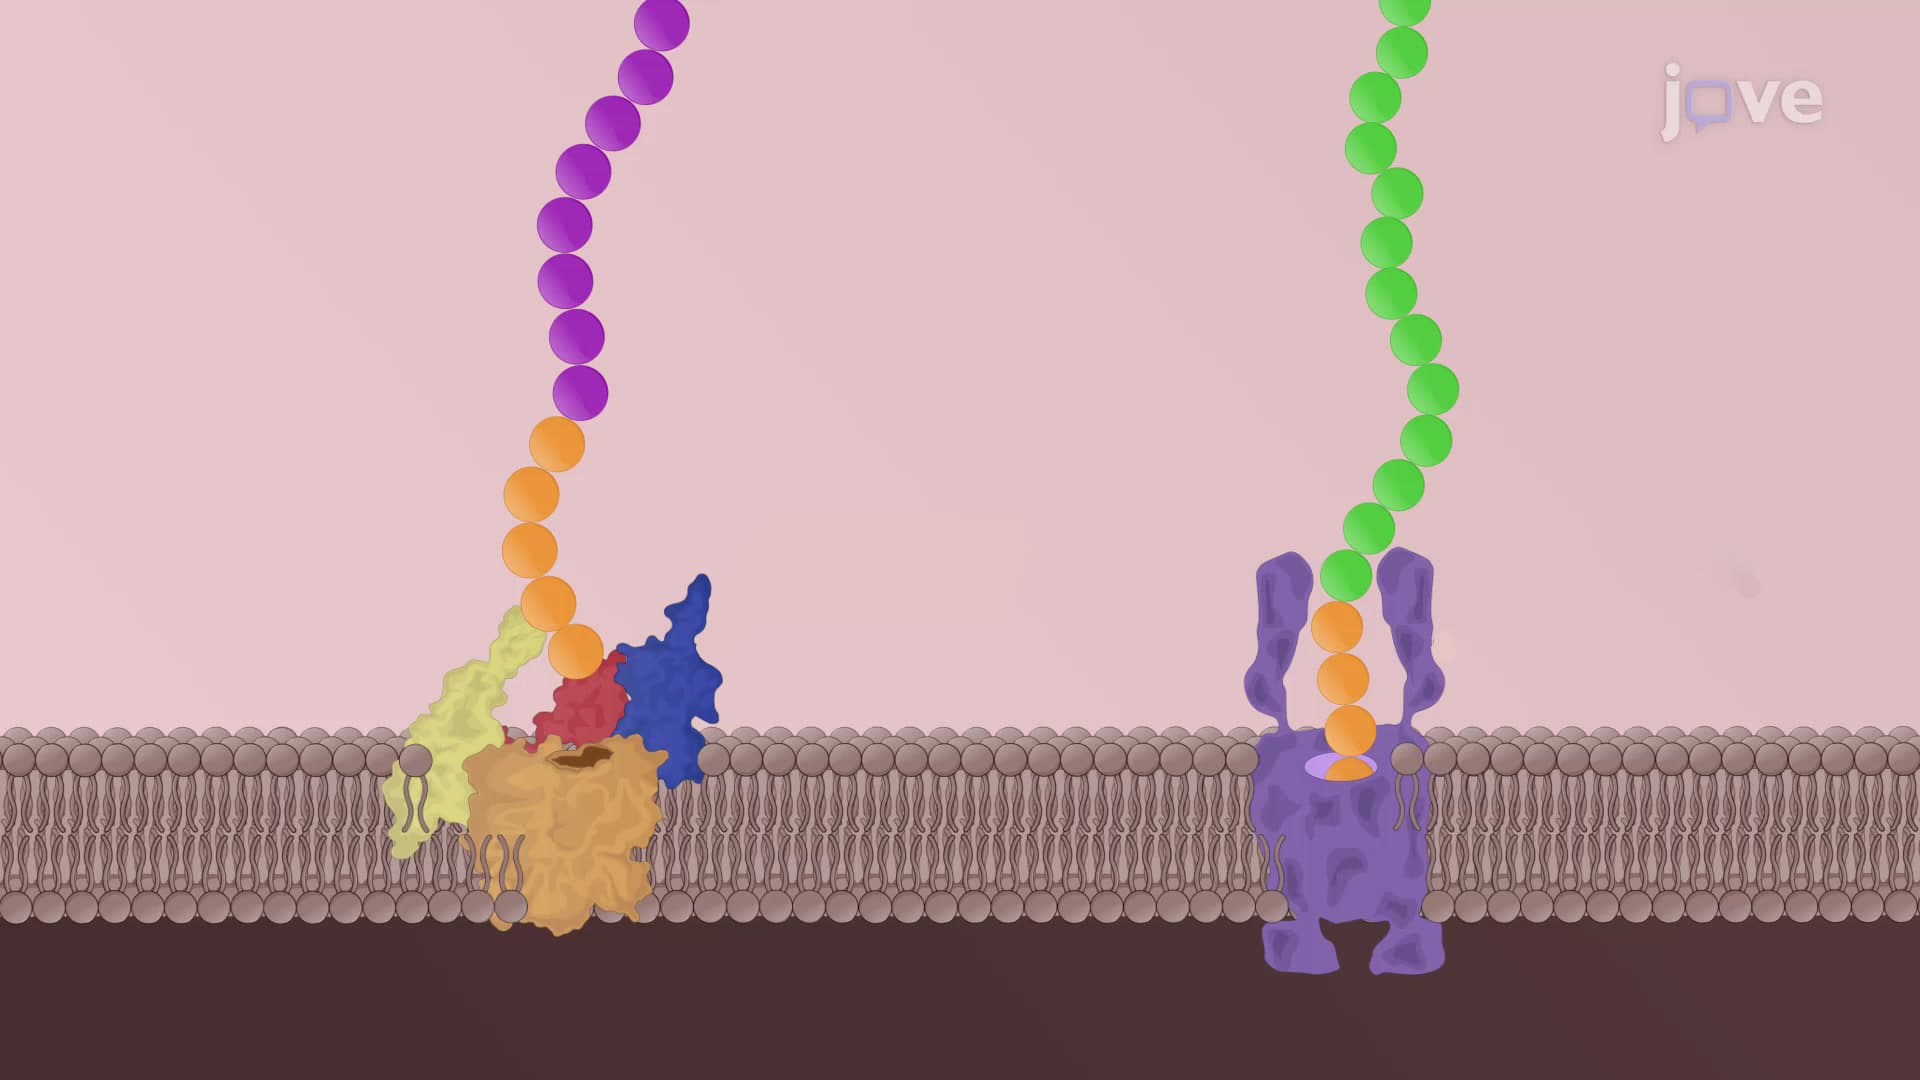
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:20
Cotranslational Protein Translocation
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
 03:00
Molecular Chaperones and Protein Folding
The...
 01:32
Export of Misfolded Proteins out of the ER
 01:34
Protein Transport into the Inner Mitochondrial Membrane
Transport of mitochondrial precursors across the TIM23 channel is driven by...