Related Experiment Video
Updated: Nov 17, 2025

Detecting and Characterizing Protein Self-Assembly In Vivo by Flow Cytometry
Published on: July 17, 2019
FAM134B-RHD Protein Clustering Drives Spontaneous Budding of Asymmetric Membranes
Marc Siggel1, Ramachandra M Bhaskara1,2,3, Melanie K Moesser1
1Department of Theoretical Biophysics, Max Planck Institute of Biophysics, Max-von-Laue Str. 3, 60438 Frankfurt am Main, Germany.

Abstract:
Living cells constantly remodel the shape of their lipid membranes. In the endoplasmic reticulum (ER), the reticulon homology domain (RHD) of the reticulophagy regulator 1 (RETR1/FAM134B) forms dense autophagic puncta that are associated with membrane removal by ER-phagy. In molecular dynamics (MD) simulations, we find that FAM134B-RHD spontaneously forms clusters, driven in part by curvature-mediated attractions. At a critical size, as in a nucleation process, the FAM134B-RHD clusters induce the formation of membrane buds. The kinetics of budding depends sensitively on protein concentration and bilayer asymmetry. Our MD simulations shed light on the role of FAM134B-RHD in ER-phagy and show that membrane asymmetry can be used to modulate the kinetic barrier for membrane remodeling.
Related Concept Videos
 01:45
Vesicular Tubular Clusters
With the help of motor proteins such...
 01:25
Rab Cascades
 01:32
Pinching-off of Coated Vesicles
 01:14
Rab Proteins
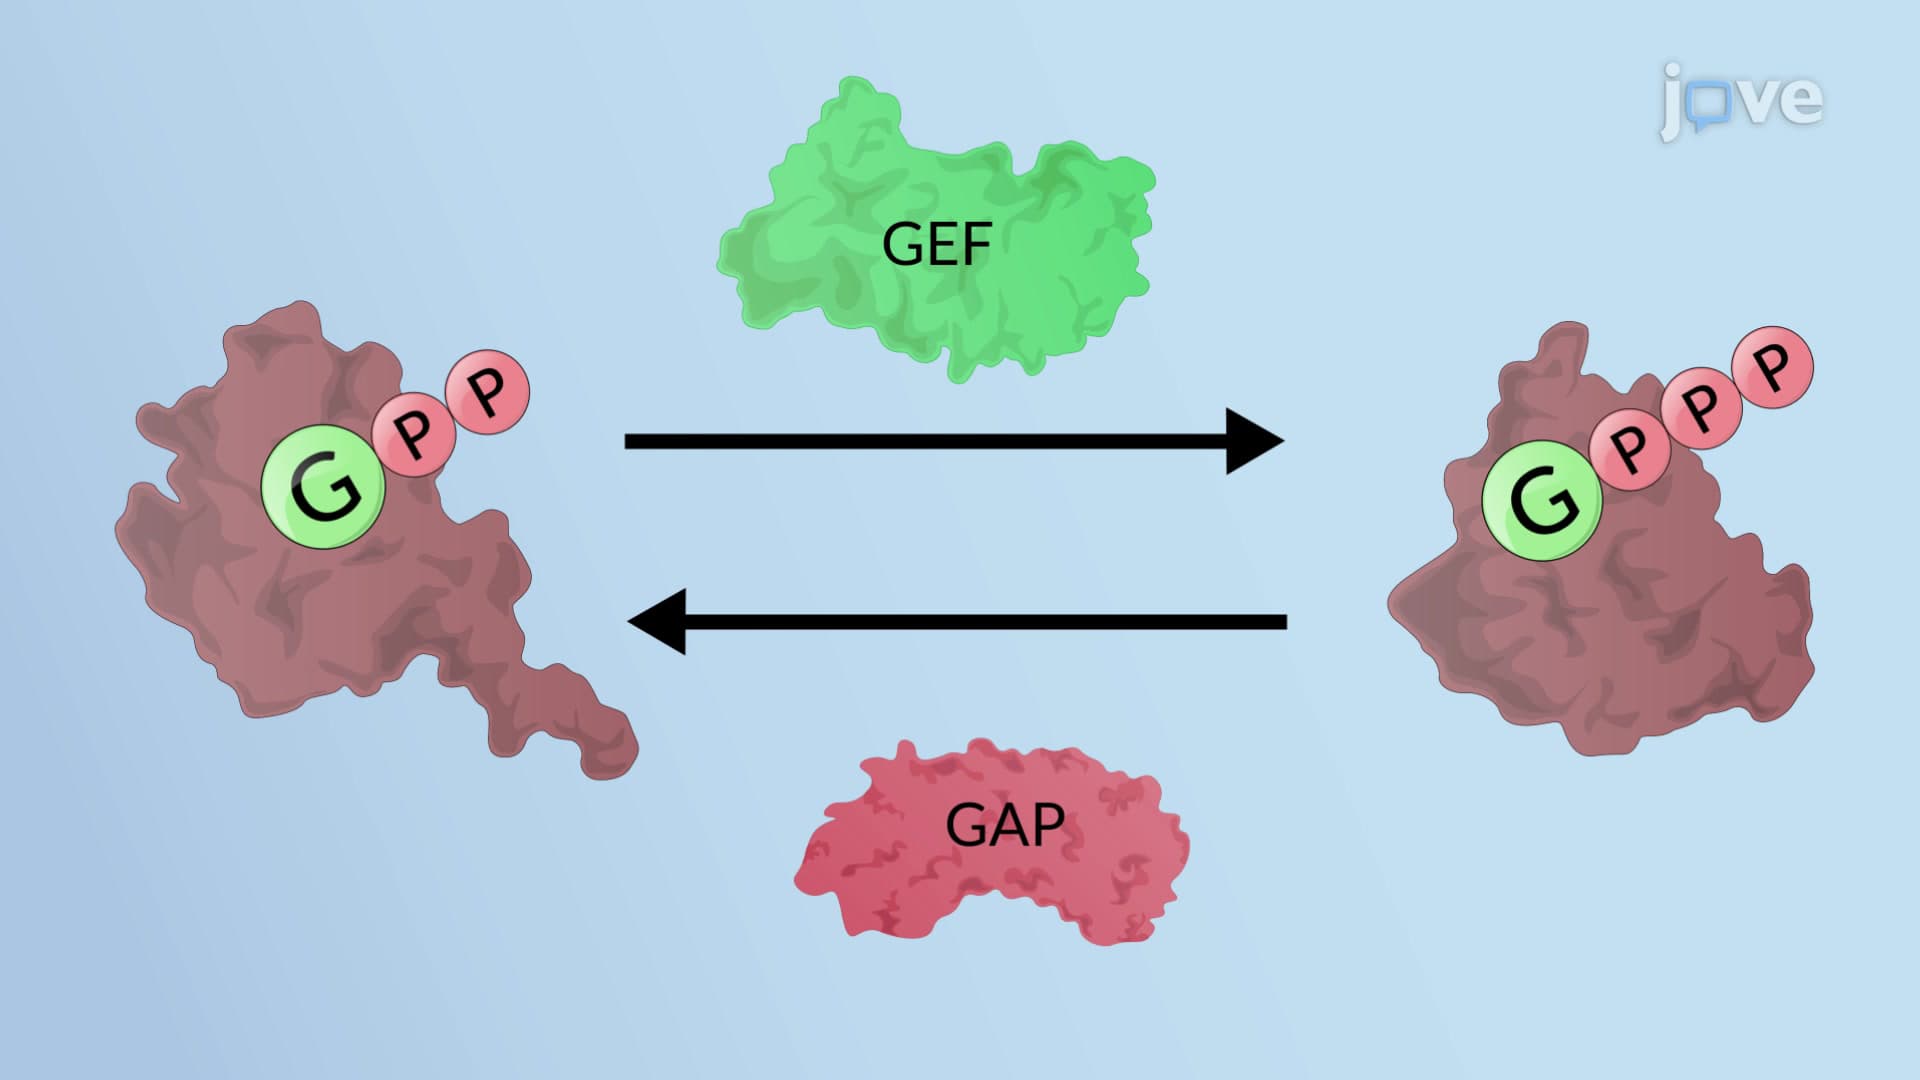
Rab proteins switch between a cytosolic, GDP-bound inactive state and a membrane-anchored, GTP-bound active state. By themselves, Rabs show slow rates of GDP/GTP exchange and GTP hydrolysis. Thus, Rab proteins are considered...
 00:59
Mechanisms of Membrane Domain Formation
Another mechanism for membrane domain formation involves membrane proteins interacting with...
 01:39
Mechanism of Filopodia Formation
Their main function is to guide migrating cells during normal tissue morphogenesis or cancer metastasis by recognizing and making initial contacts with the extracellular matrix. However, they can also act as stationary cell anchors or help to establish communication...