Related Experiment Video
Updated: Nov 12, 2025
Chemical Dimerization-Induced Protein Condensates on Telomeres
Published on: April 12, 2021
N-terminal Domain of TDP43 Enhances Liquid-Liquid Phase Separation of Globular Proteins
G Campbell Carter1, Chia-Heng Hsiung1, Leman Simpson2
1Department of Chemistry, The Pennsylvania State University, University Park, PA 16802, United States; Department of Biochemistry and Molecular Biology, The Pennsylvania State University, University Park, PA 16802, United States.

Liquid-liquid phase separation (LLPS) of proteins is involved in a growing number of cellular processes. Most proteins with LLPS harbor intrinsically disordered regions (IDR), which serve as a guideline to search for cellular proteins that potentially phase separate. Herein, we reveal that oligomerization lowers the barriers for LLPS and could act as a general mechanism to enhance LLPS of proteins domains independent of IDR. Using TDP43 as a model system, we found that deleting its IDR resulted in LLPS that was dependent on the oligomerization of the N-terminal domain (NTD). Replacing TDP43's NTD with other oligomerization domains enhanced the LLPS proportionately to the state of oligomerization. In addition to TDP43, fusing NTD to other globular proteins without known LLPS behavior also drove their phase separation in a manner dependent on oligomerization. Finally, we demonstrate that heterooligomers composed of NTD-fused proteins can be driven into droplets through NTD interactions. Our results potentiate a new paradigm for using oligomerization domains as a signature to systematically identify cellular proteins with LLPS behavior, thus broadening the scope of this exciting research field.
Liquid-liquid phase separation (LLPS) of proteins is involved in a growing number of cellular processes. Most proteins with LLPS harbor intrinsically disordered regions (IDR), which serve as a guideline to search for cellular proteins that potentially phase separate. Herein, we reveal that oligomerization lowers the barriers for LLPS and could act as a general mechanism to enhance LLPS of proteins domains independent of IDR. Using TDP43 as a model system, we found that deleting its IDR resulted in LLPS that was dependent on the oligomerization of the N-terminal domain (NTD). Replacing TDP43's NTD with other oligomerization domains enhanced the LLPS proportionately to the state of oligomerization. In addition to TDP43, fusing NTD to other globular proteins without known LLPS behavior also drove their phase separation in a manner dependent on oligomerization. Finally, we demonstrate that heterooligomers composed of NTD-fused proteins can be driven into droplets through NTD interactions. Our results potentiate a new paradigm for using oligomerization domains as a signature to systematically identify cellular proteins with LLPS behavior, thus broadening the scope of this exciting research field.
Related Concept Videos
 01:45
Tail-anchoring of Proteins in the ER Membrane
 00:59
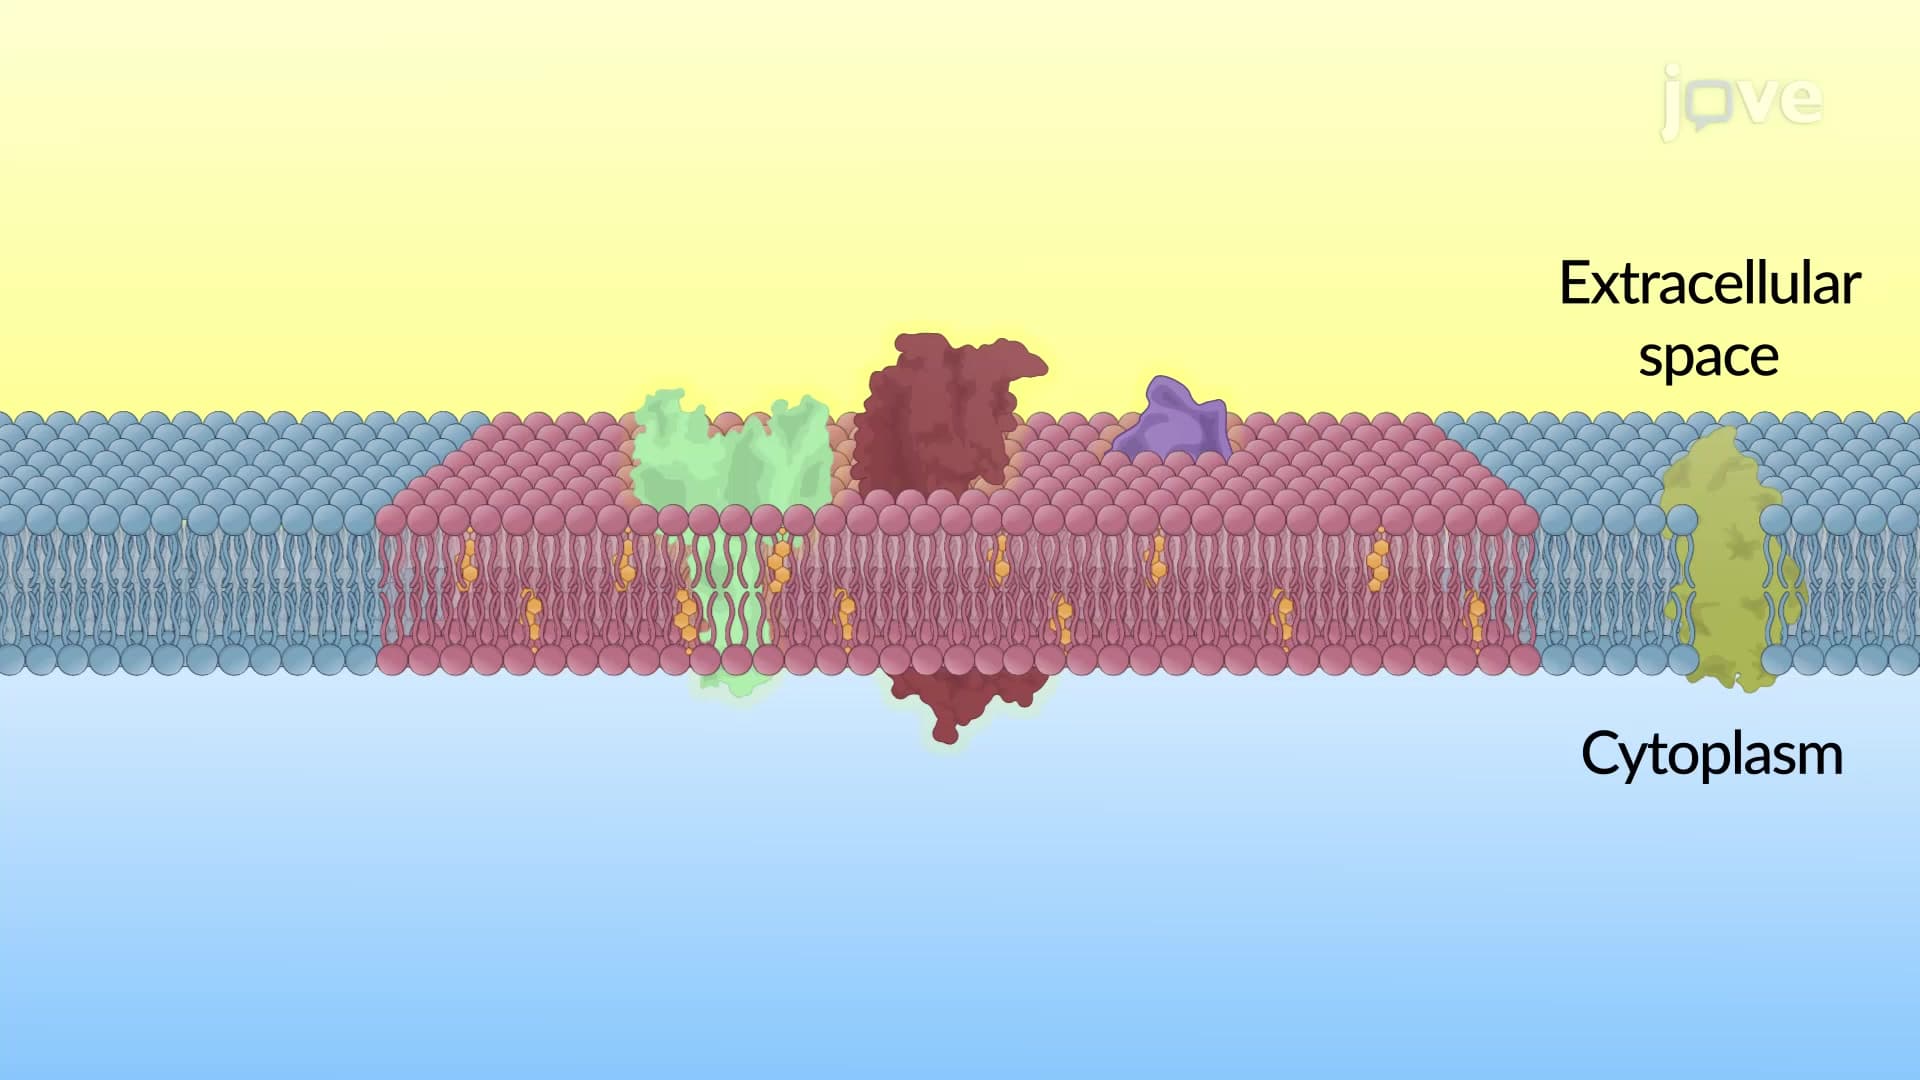
Mechanisms of Membrane Domain Formation
Another mechanism for membrane domain formation involves membrane proteins interacting with...
 01:26
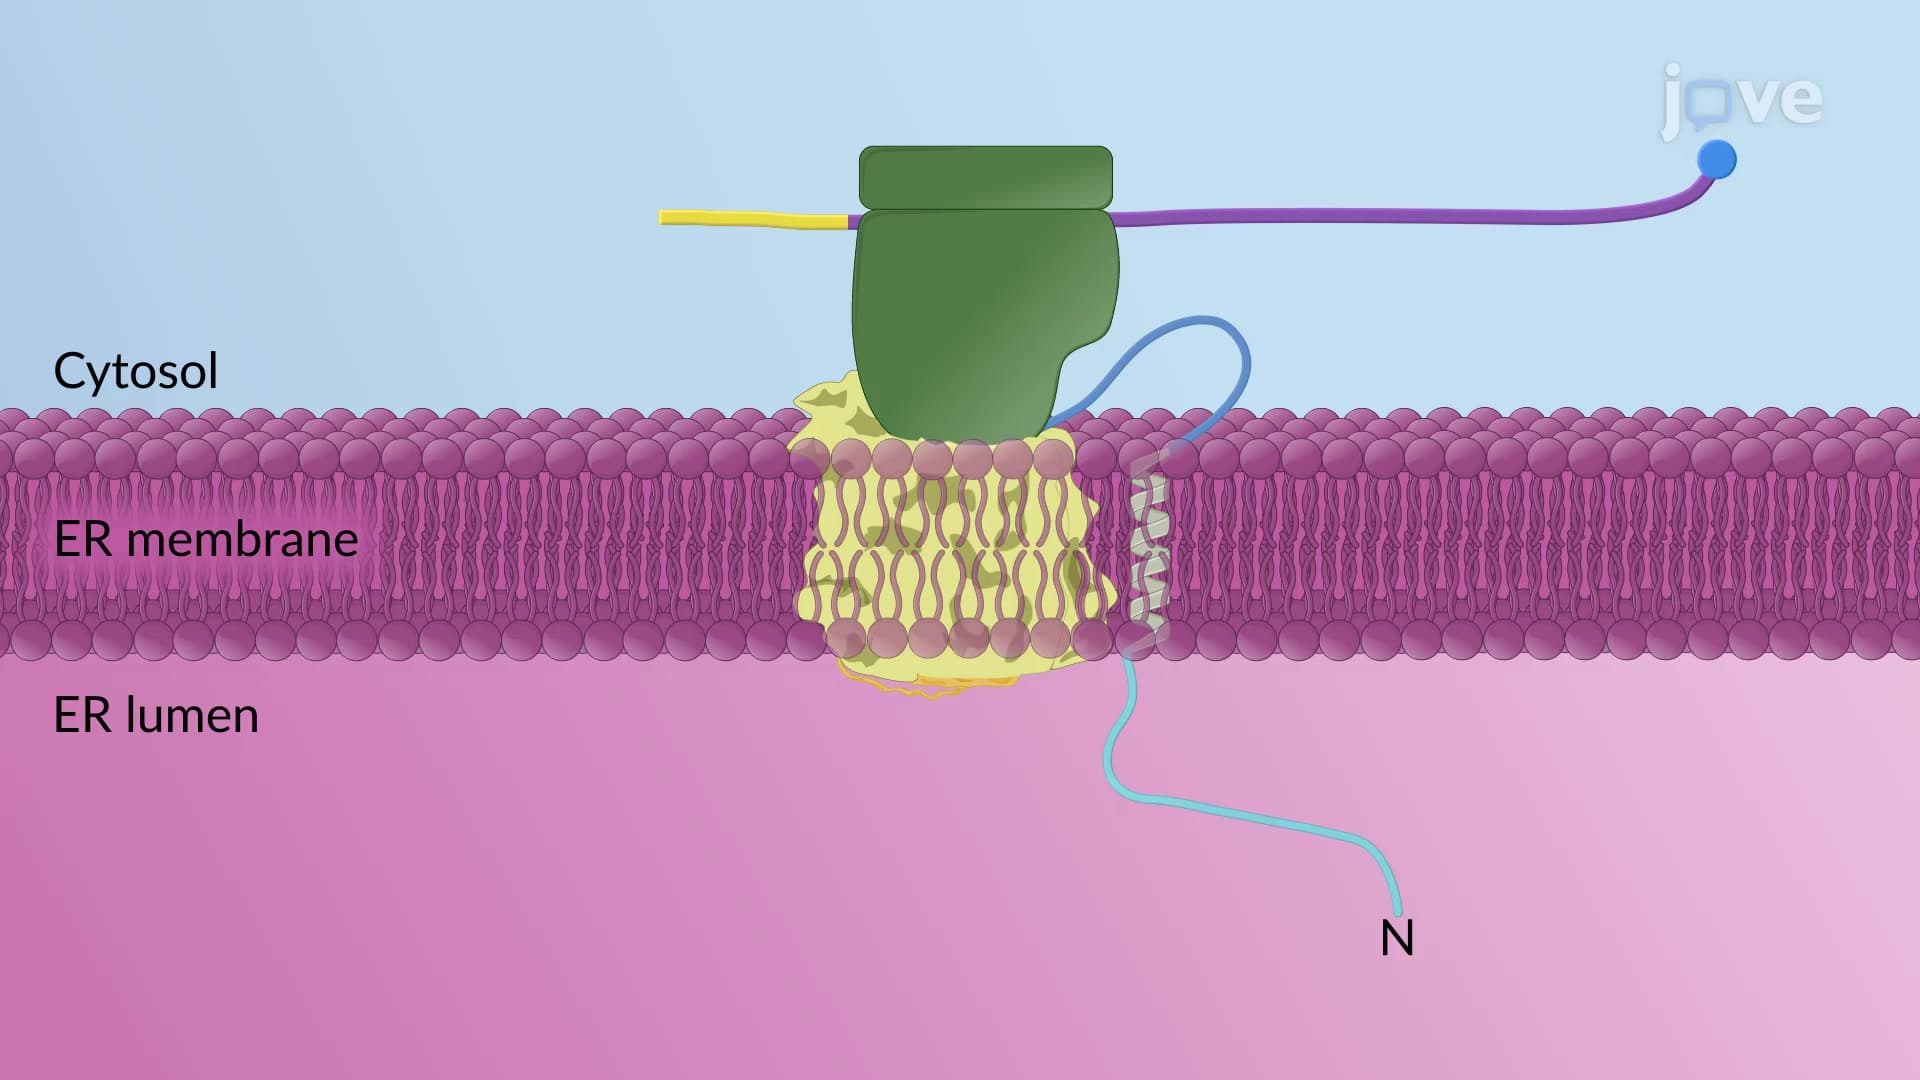
Insertion of Single-pass Transmembrane Proteins in the RER
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
 01:18
Membrane Domains
Protein Domains
The membrane comprises a group of distinct proteins responsible for carrying out a cell's specific function. For example, the plasma membrane of the human sperm, or a single germ cell, contains a unique set of proteins in the...
 02:18
Intrinsically Disordered Proteins