Related Experiment Video
Updated: Oct 28, 2025

Spontaneous Formation and Rearrangement of Artificial Lipid Nanotube Networks as a Bottom-Up Model for Endoplasmic Reticulum
Published on: January 22, 2019
Unraveling How Multivalency Triggers Shape Deformation of Sub-100 nm Lipid Vesicles
Hyeonjin Park1,2, Tun Naw Sut1,2, Bo Kyeong Yoon1
1School of Chemical Engineering, Sungkyunkwan University, Suwon 16419, Republic of Korea.

Abstract:
Multivalent ligand-receptor interactions are critical to the function of membrane-enveloped biological and biomimetic nanoparticles, yet resulting nanoparticle shape changes are rarely investigated. Using the localized surface plasmon resonance (LSPR) sensing technique, we tracked the attachment of biotinylated, sub-100 nm lipid vesicles to a streptavidin-functionalized supported lipid bilayer (SLB) and developed an analytical model to extract quantitative details about the vesicle-SLB contact region. The experimental results were supported by theoretical analyses of biotin-streptavidin complex formation and corresponding structural and energetic aspects of vesicle deformation. Our findings reveal how varying the surface densities of streptavidin receptors in the SLB and biotin ligands in the vesicles affects the extent of nanometer-scale vesicle deformation. We also identify conditions, i.e., a critical ligand density, at which appreciable vesicle deformation began, which provides insight into how the membrane bending energy partially counterposes the multivalent binding interaction energy. These findings are generalizable to various multivalent ligand-receptor systems.
More Related Videos
Related Concept Videos
 01:32
Pinching-off of Coated Vesicles
 00:59
Mechanisms of Membrane Domain Formation
Another mechanism for membrane domain formation involves membrane proteins interacting with...
 01:15
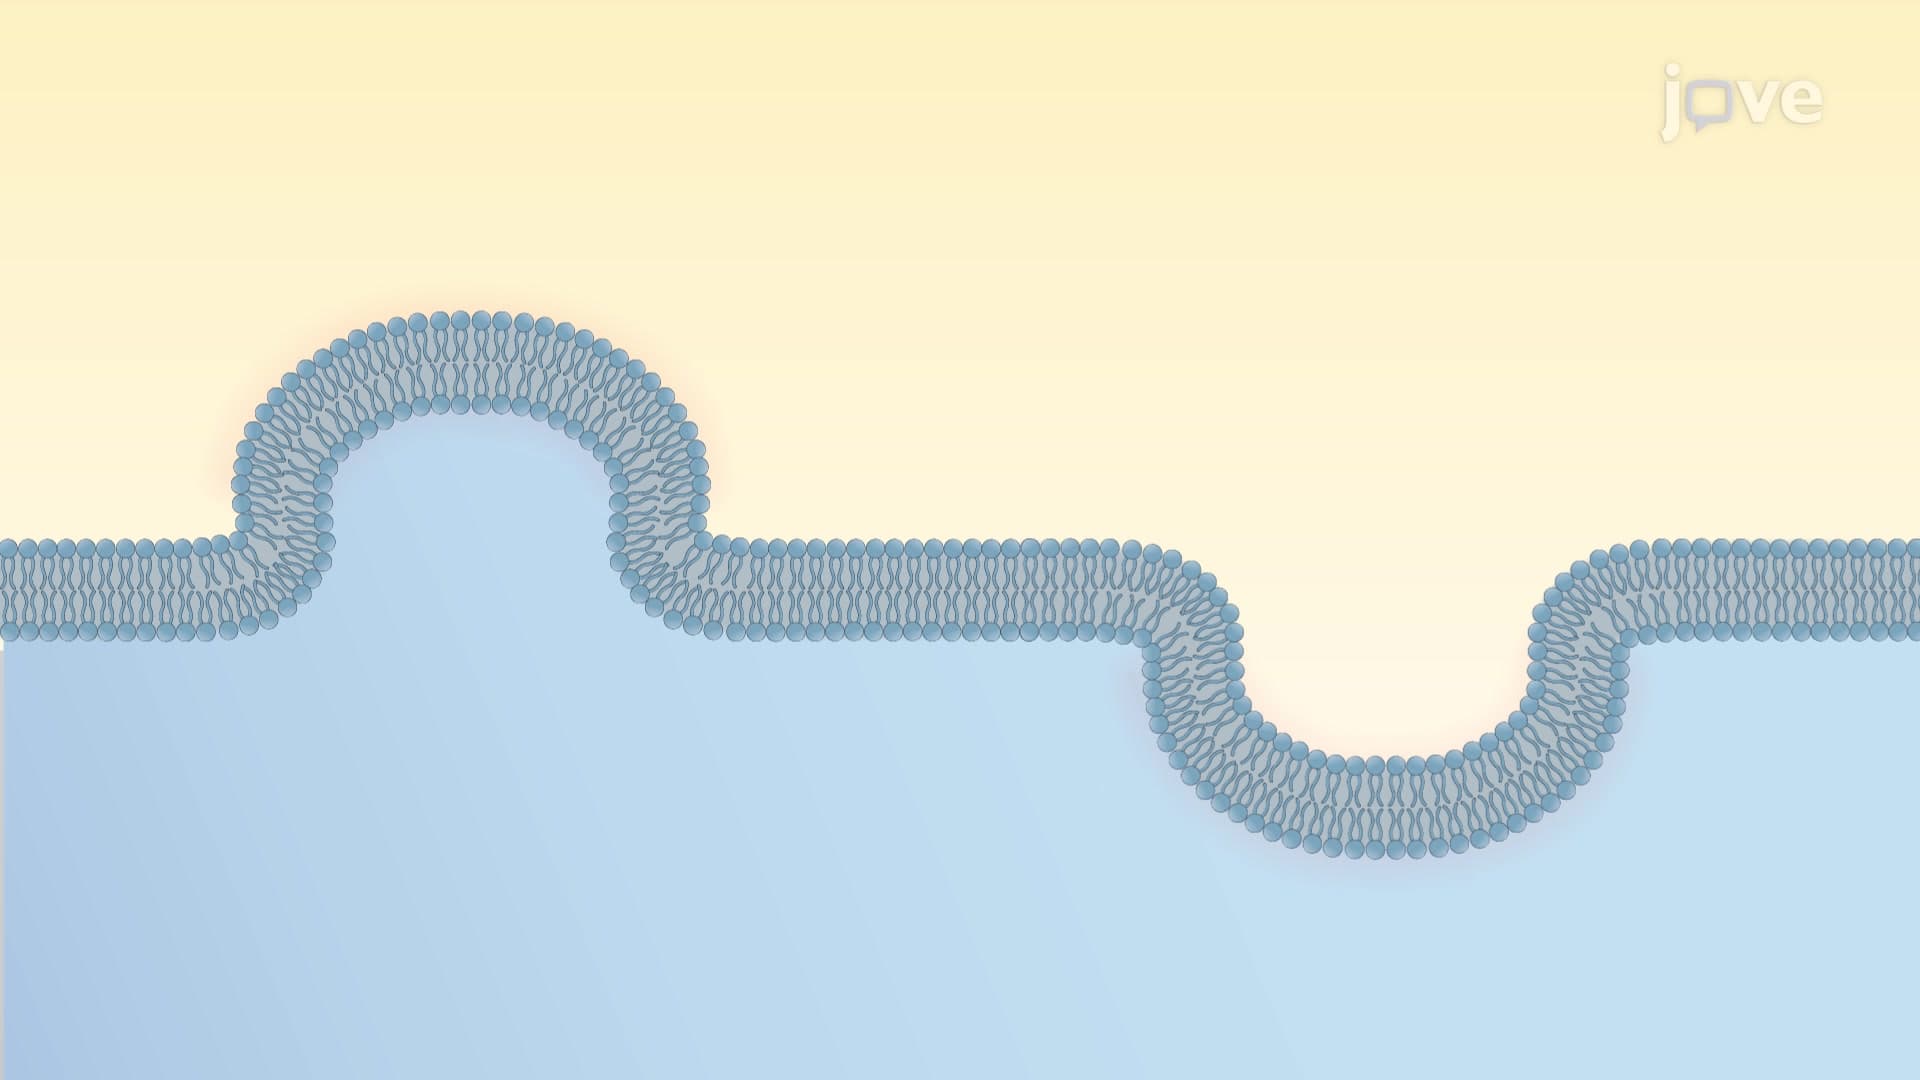
Mechanisms of Membrane-bending
Membrane bending can happen due to intrinsic changes in lipid composition or extrinsic association with different proteins. The proteins involved...
 01:43
SNAREs and Membrane Fusion
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
 01:12
Clathrin Coated Vesicles
 01:26
Fusion of Secretory Vesicles with the Plasma Membrane
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...