Related Experiment Video
Updated: Oct 20, 2025

Functional Complementation Analysis FCA: A Laboratory Exercise Designed and Implemented to Supplement the Teaching of Biochemical Pathways
Published on: June 24, 2016
Revisiting AMPylation through the lens of Fic enzymes
1Department of Biochemistry and Signal Transduction, University Medical Center Hamburg-Eppendorf (UKE), Martinistr. 52, 20246, Hamburg, Germany; Present address: Department of Molecular Biology, University of Texas Southwestern Medical Center, Dallas, TX, USA.

Abstract:
AMPylation, a post-translational modification (PTM) first discovered in the late 1960s, is catalyzed by adenosine monophosphate (AMP)-transferring enzymes. The observation that filamentation-induced-by-cyclic-AMP (fic) enzymes are associated with this unique PTM revealed that AMPylation plays a major role in hijacking of host signaling by pathogenic bacteria during infection. Studies over the past decade showed that AMPylation is conserved across all kingdoms of life and, outside their role in infection, also modulates cellular functions. Many aspects of AMPylation are yet to be uncovered. In this review we present the advancement in research on AMPylation and Fic enzymes as well as other distinct classes of enzymes that catalyze AMPylation.
More Related Videos
 05:33
Author Spotlight: Characterizing Novel Enzymes from Extremophiles and Common Pathogens to Understand DNA Repair and Replication
Published on: July 5, 2024
 10:21
Expression, Purification, Crystallization, and Enzyme Assays of Fumarylacetoacetate Hydrolase Domain-Containing Proteins
Published on: June 20, 2019
Related Concept Videos
 01:39
Mechanism of Filopodia Formation
Their main function is to guide migrating cells during normal tissue morphogenesis or cancer metastasis by recognizing and making initial contacts with the extracellular matrix. However, they can also act as stationary cell anchors or help to establish communication...
 01:22
Amplifying Signals via Enzymatic Cascade
 01:32
Pinching-off of Coated Vesicles
 01:27
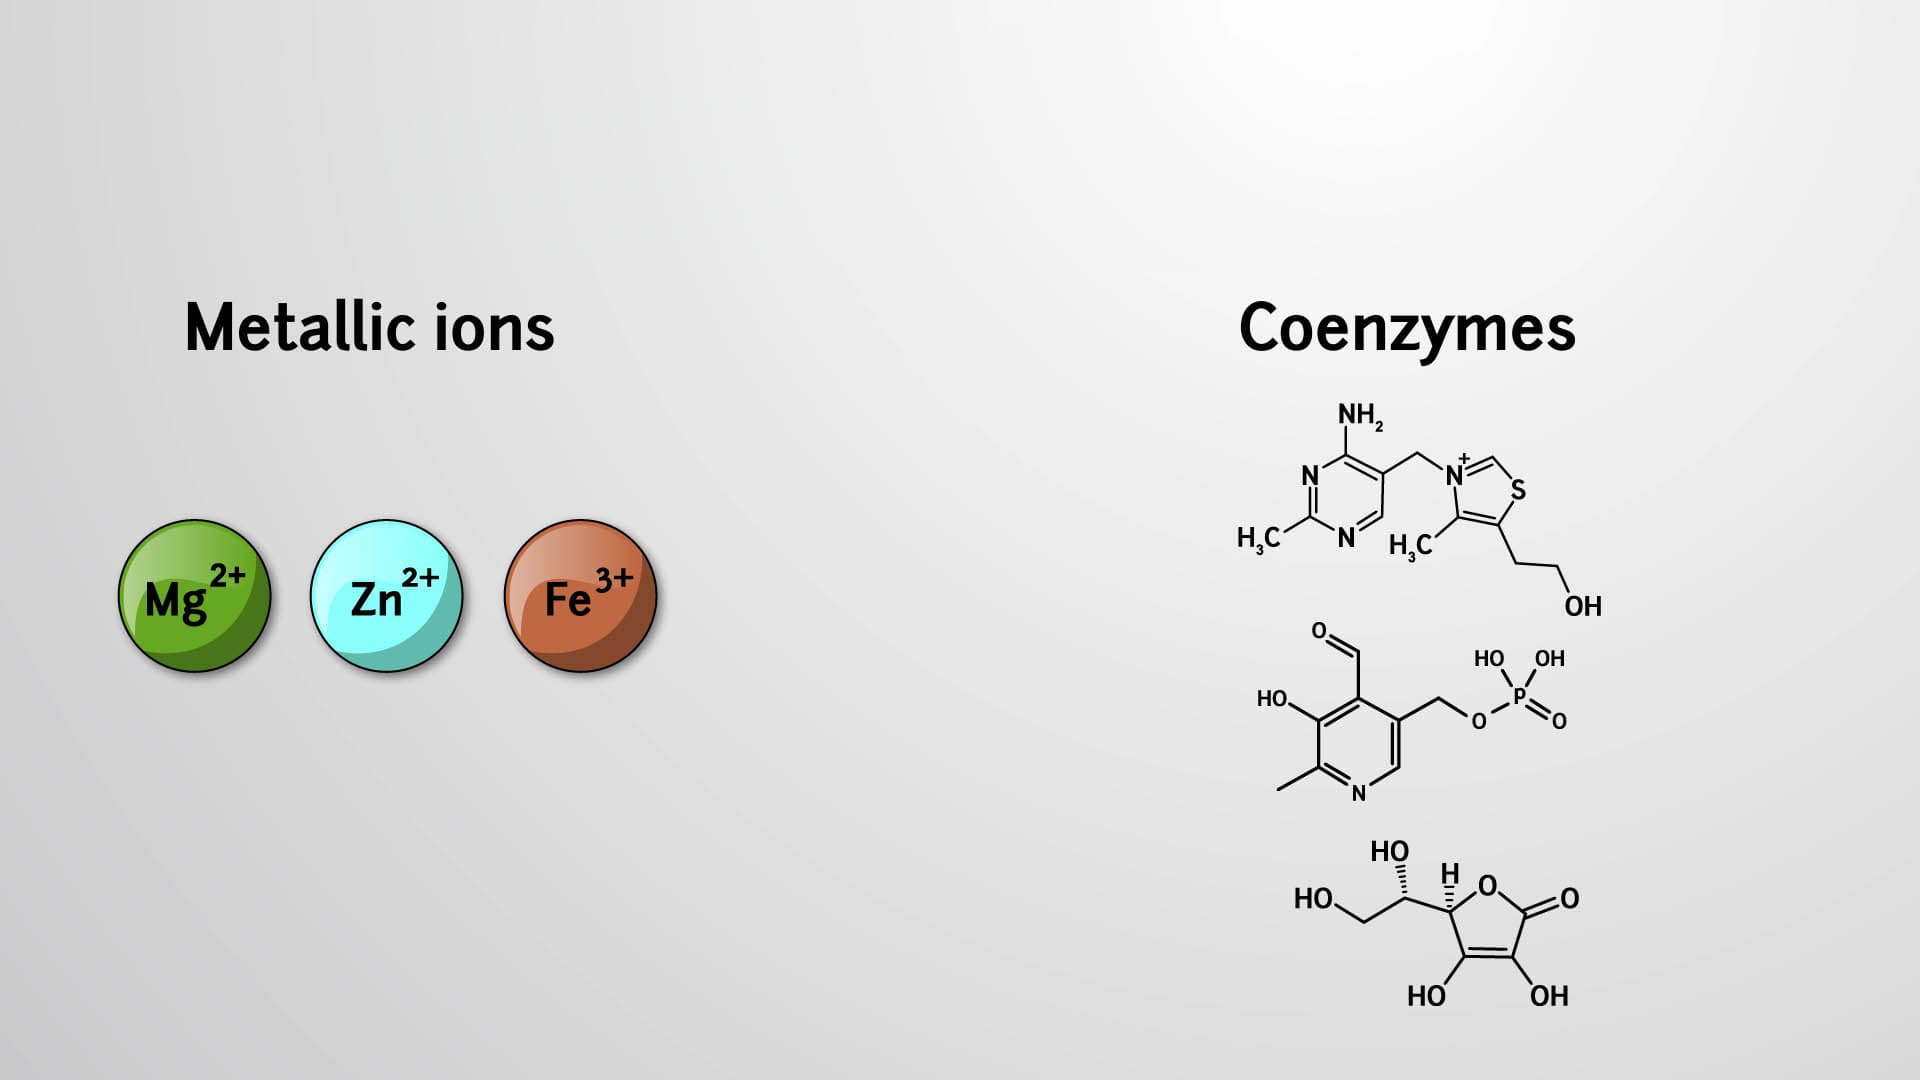
Cofactors and Coenzymes
 01:14
Generation of Straight or Branched Actin Filaments
Arp2/3 Complex
Arp2/3 complex is a seven-subunit complex consisting of two proteins similar to actin- Arp2 and Arp3, and five other subunits that help keep Arp2 and Arp3 inactive. When required, the complex is...
 01:42
Actin Polymerization
The nucleation phase involves forming a stable nucleus consisting of three actin monomers to form a new actin filament. Actin-binding proteins such as formins and Arp2/3 complex help filament growth post-nucleation. The Formins form straight...