Related Experiment Video
Updated: Oct 14, 2025
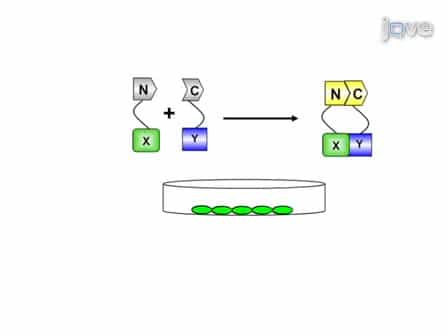

Bimolecular Fluorescence Complementation
Published on: April 15, 2011
Ift88, but not Kif3a, is required for establishment of the periciliary membrane compartment
Fruzsina Kotsis1, Heike Janusch1, Yujie Li1
1Department of Medicine IV - Nephrology and Primary Care, Faculty of Medicine and Medical Center - University of Freiburg, Freiburg, Germany.

Abstract:
The primary cilium is a sensory organelle at the cell surface with integral functions in cell signaling. It contains a microtubular axoneme that is rooted in the basal body (BB) and serves as a scaffold for the movement of intraflagellar transport (IFT) particles by Kinesin-2 along the cilium. Ift88, a member of the anterograde moving IFT-B1 complex, as well as the Kinesin-2 subunit Kif3a are required for cilia formation. To facilitate signaling, the cilium restricts the access of molecules to its membrane ("ciliary gate"). This is thought to be mediated by cytoskeletal barriers ("subciliary domains") originating from the BB subdistal/distal appendages, the periciliary membrane compartment (PCMC) as well as the transition fibers and zone (TF/TZ). The PCMC is a poorly characterized membrane domain surrounding the ciliary base with exclusion of certain apical membrane proteins. Here we describe that Ift88, but not Kinesin-2, is required for the establishment of the PCMC in MDCK cells. Likewise, in C. elegans mutants of the Ift88 ortholog osm-5 fail to establish the PCMC, while Kinesin-2 deficient osm-3 mutants form PCMCs normally. Furthermore, disruption of IFT-B1 into two subcomplexes, while disrupting ciliogenesis, does not interfere with PCMC formation. Our findings suggest that cilia are not a prerequisite for the formation of the PCMC, and that separate machineries with partially overlapping functions are required for the establishment of each.
Related Concept Videos
 01:39
Mechanism of Filopodia Formation
Their main function is to guide migrating cells during normal tissue morphogenesis or cancer metastasis by recognizing and making initial contacts with the extracellular matrix. However, they can also act as stationary cell anchors or help to establish communication...
 01:33
Coat Assembly and GTPases
Coat assembly depends on the local availability of phosphatidylinositol phosphates or PIPs and GTP-binding proteins. Adaptor proteins, which link the coat proteins to the membrane, bind to these PIPs and play a crucial role in controlling...
 01:42
Phosphoinositides and PIPs
Different phosphoinositides are synthesized and recruited on the cytosolic face of the plasma membrane. The localization of specific phosphoinositides concentrated in separate membrane...
 01:35
Disassembly of Intermediate Filaments
Keratin proteins, found at the cell periphery near cell junctions, undergo a cycle of assembly and disassembly. In Type...
 01:45
Vesicular Tubular Clusters
With the help of motor proteins such...
 01:32
Pinching-off of Coated Vesicles