Related Experiment Video
Updated: Aug 31, 2025

Genetic Manipulation in Δku80 Strains for Functional Genomic Analysis of Toxoplasma gondii
Published on: July 12, 2013
An apical protein, Pcr2, is required for persistent movement by the human parasite Toxoplasma gondii
Jonathan Munera Lopez1, Isadonna F Tengganu1, Jun Liu2
1Biodesign Center for Mechanisms of Evolution/School of Life Sciences, Arizona State University, Tempe, Arizona, United States of America.

Abstract:
The phylum Apicomplexa includes thousands of species of unicellular parasites that cause a wide range of human and animal diseases such as malaria and toxoplasmosis. To infect, the parasite must first initiate active movement to disseminate through tissue and invade into a host cell, and then cease moving once inside. The parasite moves by gliding on a surface, propelled by an internal cortical actomyosin-based motility apparatus. One of the most effective invaders in Apicomplexa is Toxoplasma gondii, which can infect any nucleated cell and any warm-blooded animal. During invasion, the parasite first makes contact with the host cell "head-on" with the apical complex, which features an elaborate cytoskeletal apparatus and associated structures. Here we report the identification and characterization of a new component of the apical complex, Preconoidal region protein 2 (Pcr2). Pcr2 knockout parasites replicate normally, but they are severely diminished in their capacity for host tissue destruction due to significantly impaired invasion and egress, two vital steps in the lytic cycle. When stimulated for calcium-induced egress, Pcr2 knockout parasites become active, and secrete effectors to lyse the host cell. Calcium-induced secretion of the major adhesin, MIC2, also appears to be normal. However, the movement of the Pcr2 knockout parasite is spasmodic, which drastically compromises egress. In addition to faulty motility, the ability of the Pcr2 knockout parasite to assemble the moving junction is impaired. Both defects likely contribute to the poor efficiency of invasion. Interestingly, actomyosin activity, as indicated by the motion of mEmerald tagged actin chromobody, appears to be largely unperturbed by the loss of Pcr2, raising the possibility that Pcr2 may act downstream of or in parallel with the actomyosin machinery.
Related Concept Videos
 01:10
Intracellular Movement of Viruses and Bacteria
 01:20
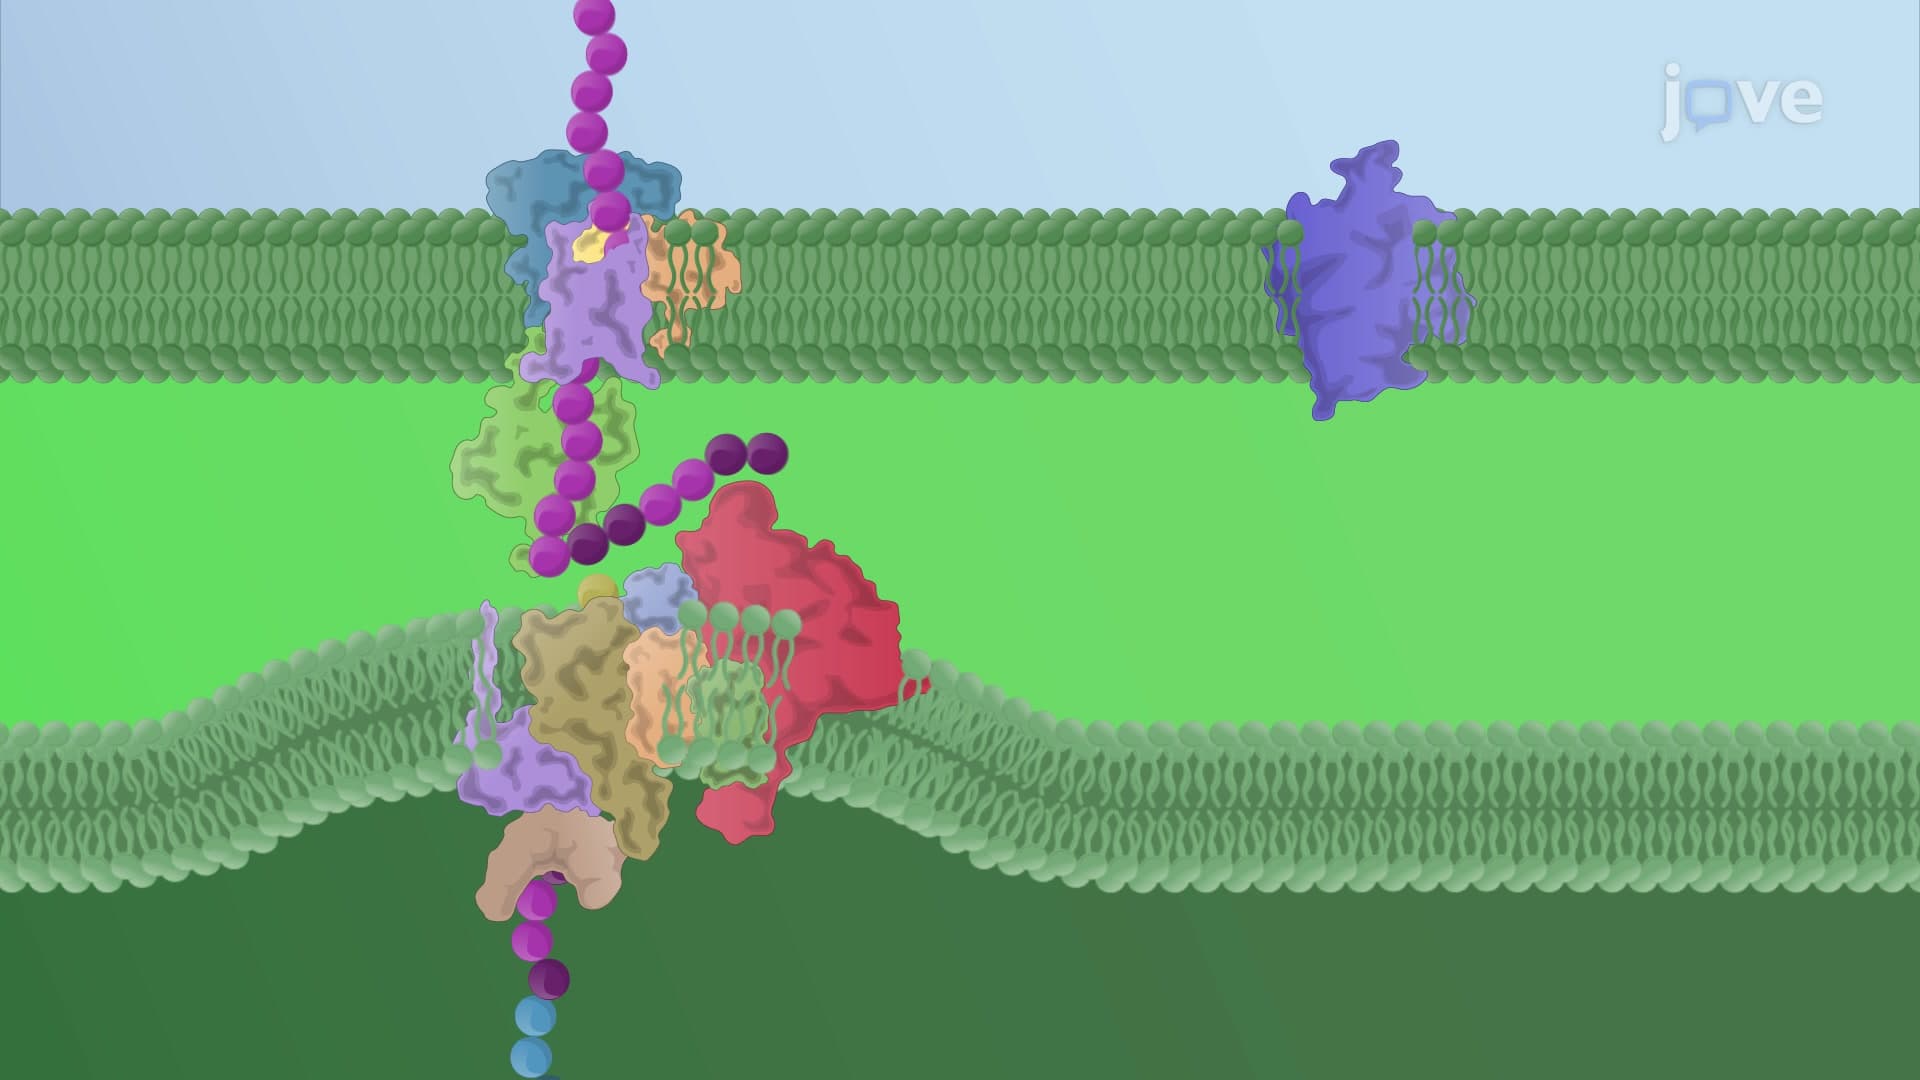
Cotranslational Protein Translocation
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
 01:11
Protein Transport to the Outer Chloroplast Membrane
Two models describe the mechanism of precursor recognition and entry across the outer membrane through the TOC complex. Model 1 suggests the newly synthesized precursor binds to the TOC receptor 159 and forms a complex.
 01:22
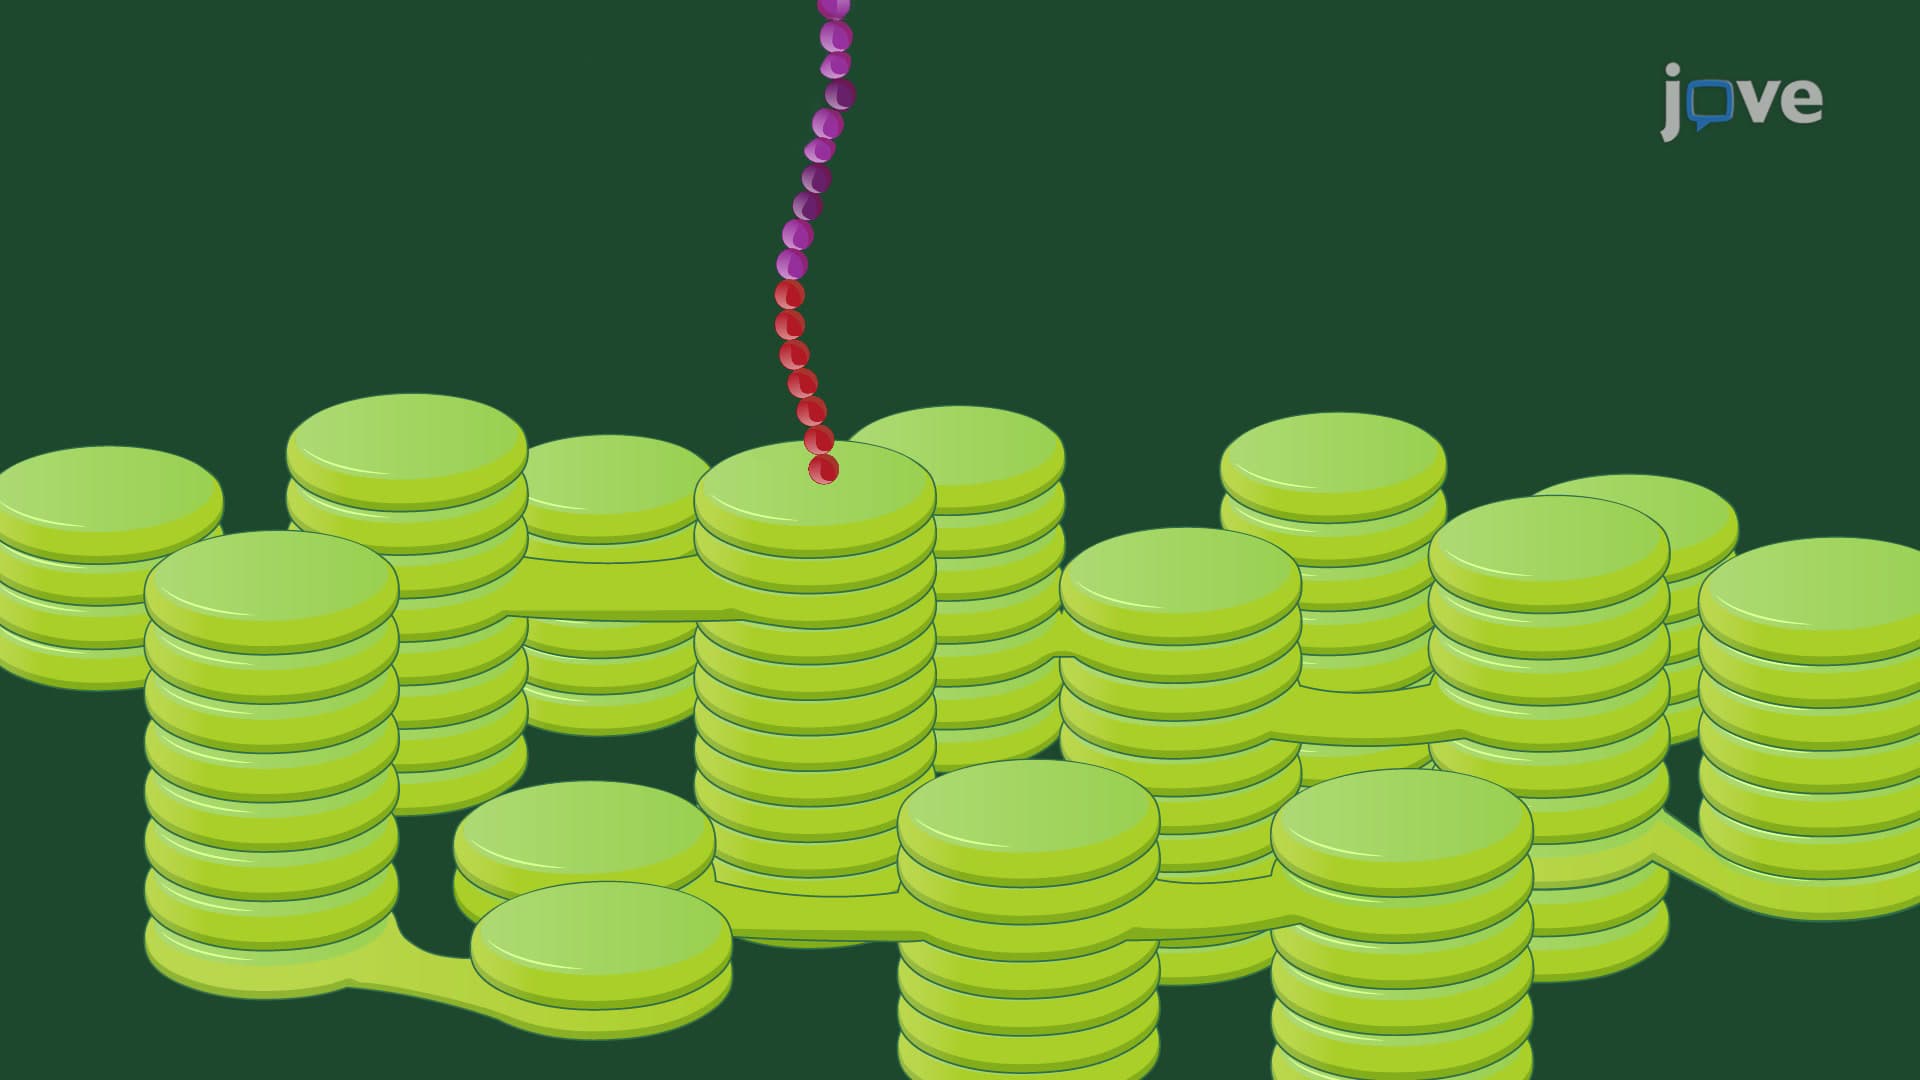
Protein Transport to the Thylakoids
 01:19
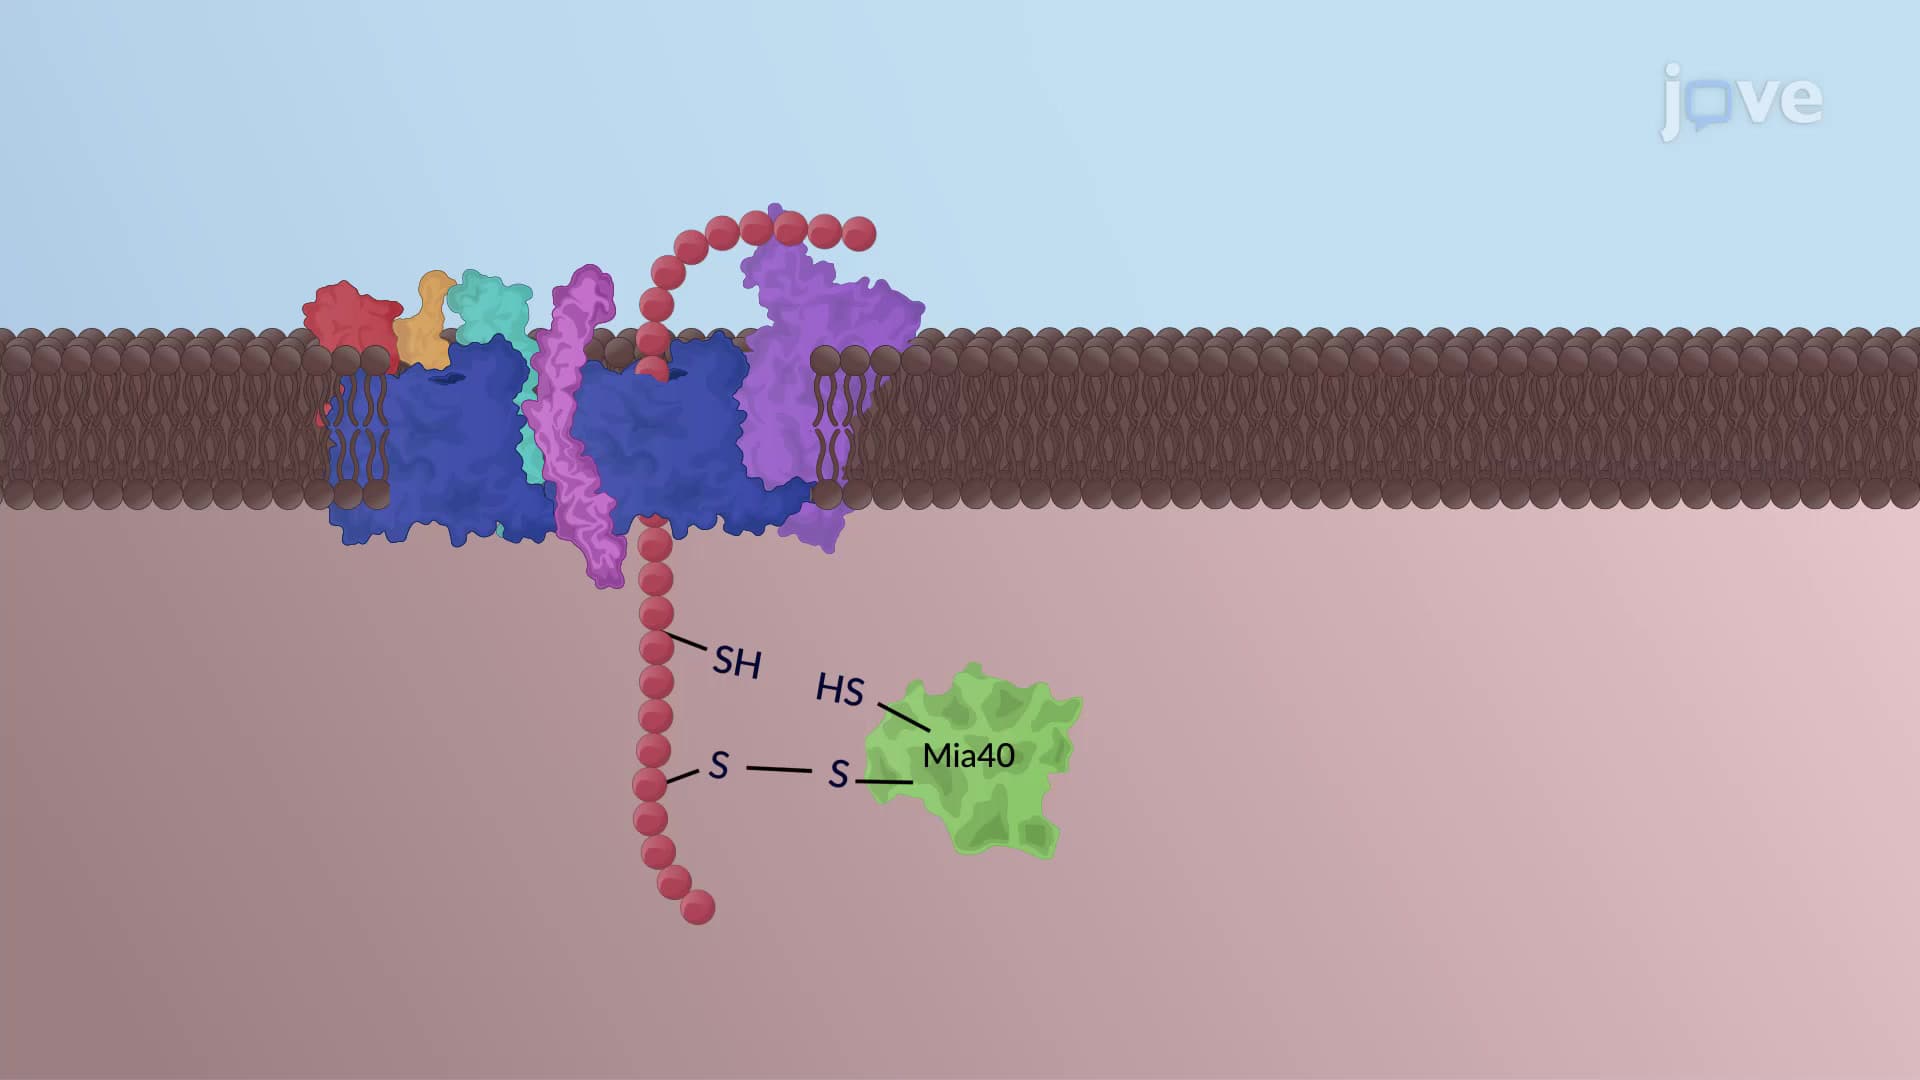
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:37
Energy to Drive Translocation
Generally, polypeptides are unfolded by two distinct...