Related Experiment Video
Updated: Aug 23, 2025

Author Spotlight: Evaluation of Protein-Condensate Dynamics in Live Human Cells
Published on: January 5, 2024
Kinetic frustration by limited bond availability controls the LAT protein condensation phase transition on membranes
Simou Sun1,2,3, Trevor GrandPre4, David T Limmer1,5,6
1Department of Chemistry, University of California, Berkeley, Berkeley, CA 94720, USA.

Abstract:
LAT is a membrane-linked scaffold protein that undergoes a phase transition to form a two-dimensional protein condensate on the membrane during T cell activation. Governed by tyrosine phosphorylation, LAT recruits various proteins that ultimately enable condensation through a percolation network of discrete and selective protein-protein interactions. Here, we describe detailed kinetic measurements of the phase transition, along with coarse-grained model simulations, that reveal that LAT condensation is kinetically frustrated by the availability of bonds to form the network. Unlike typical miscibility transitions in which compact domains may coexist at equilibrium, the LAT condensates are dynamically arrested in extended states, kinetically trapped out of equilibrium. Modeling identifies the structural basis for this kinetic arrest as the formation of spindle arrangements, favored by limited multivalent binding interactions along the flexible, intrinsically disordered LAT protein. These results reveal how local factors controlling the kinetics of LAT condensation enable formation of different, stable condensates, which may ultimately coexist within the cell.
Related Concept Videos
 01:24
Protein Diffusion in the Membrane
 01:26
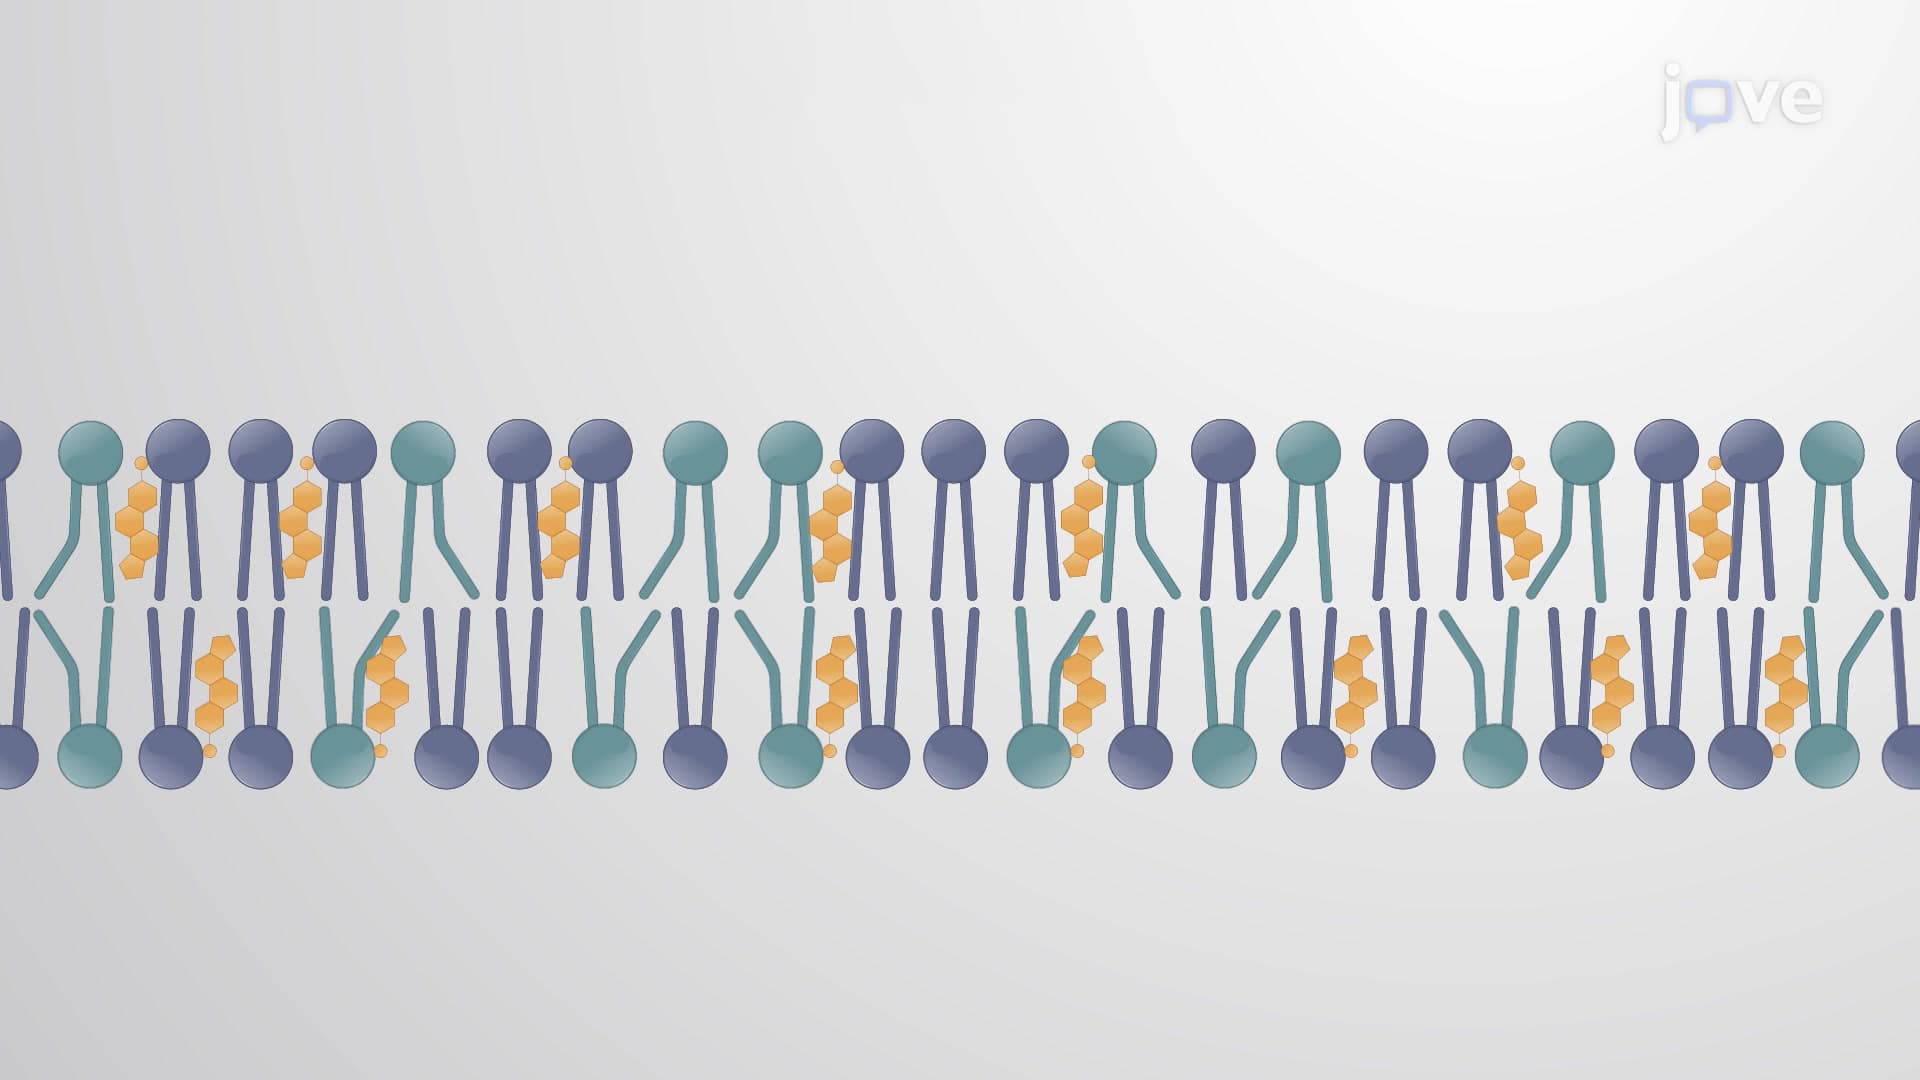
Membrane Fluidity
Mosaic nature of the membrane
The mosaic characteristic of the membrane helps the plasma membrane remain fluid. The integral proteins and lipids exist as separate but loosely-attached molecules in the membrane. The membrane is...
 01:15
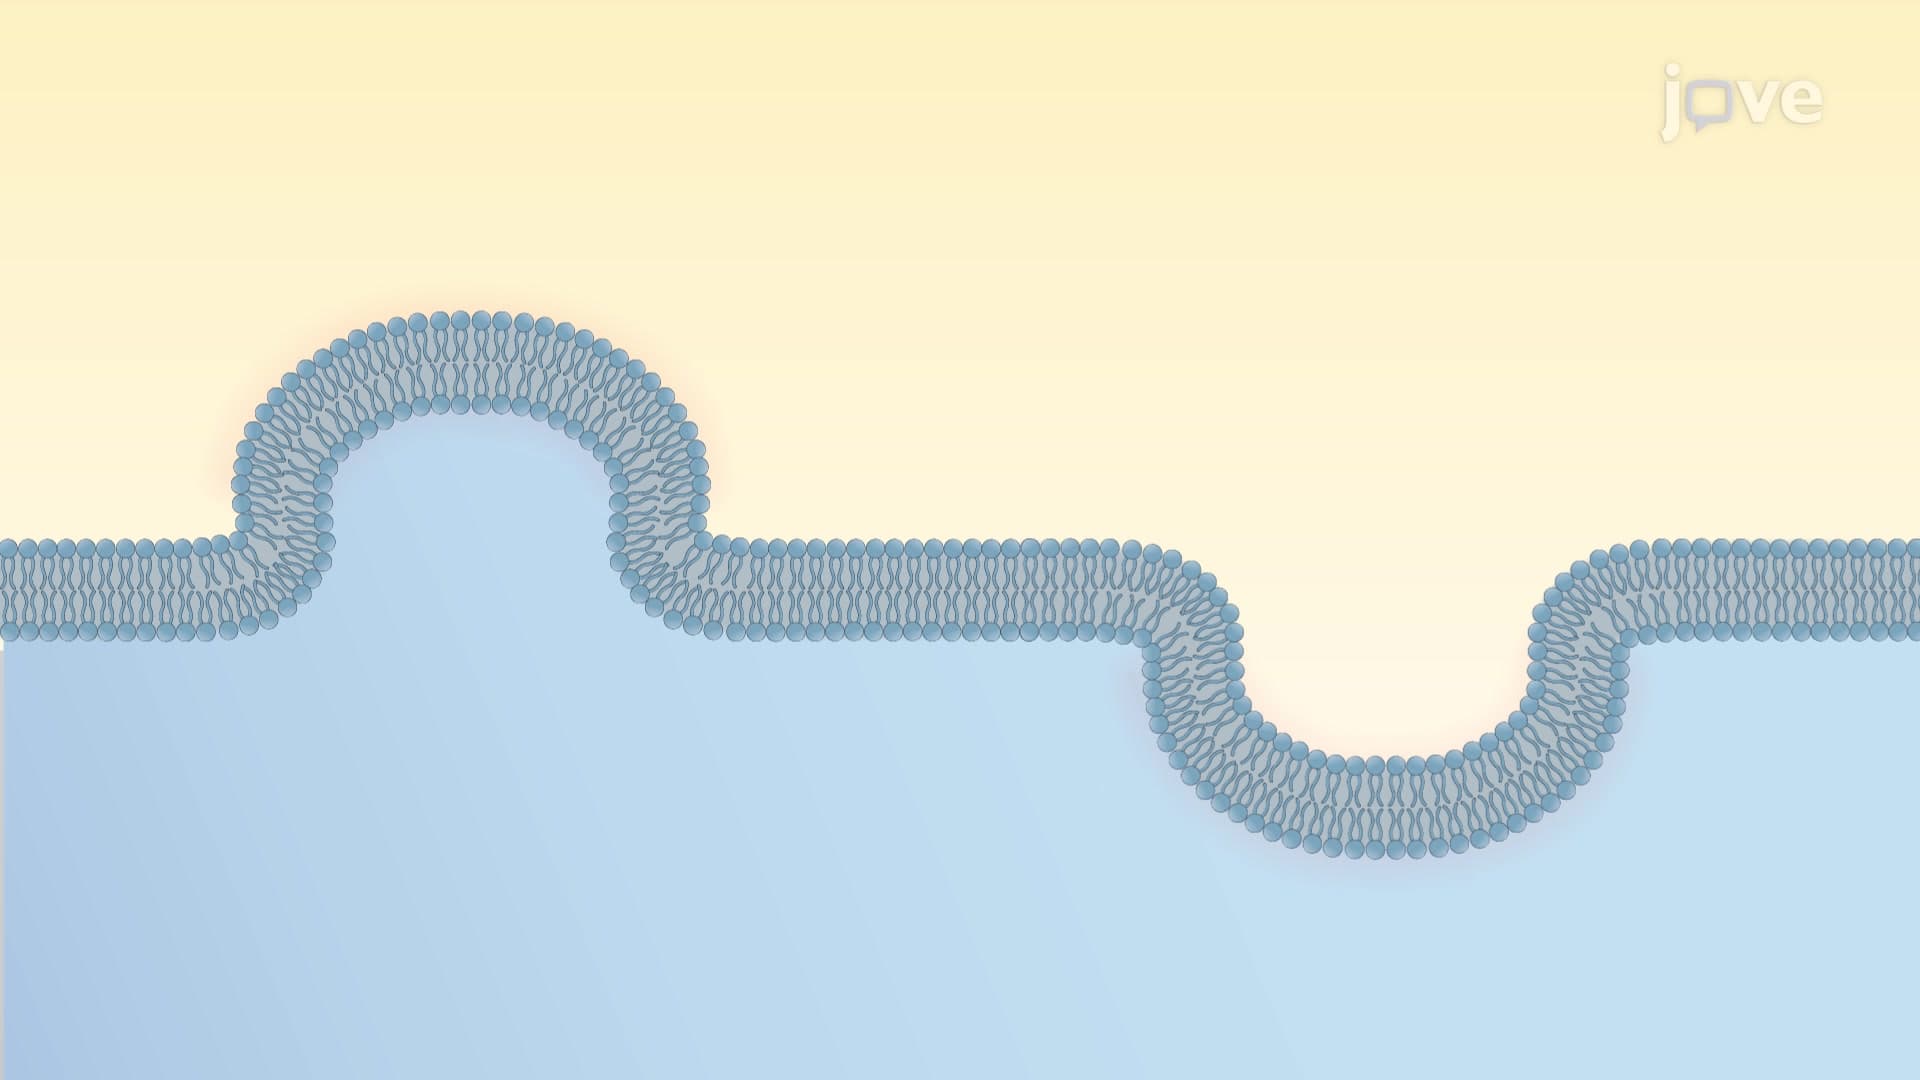
Mechanisms of Membrane-bending
Membrane bending can happen due to intrinsic changes in lipid composition or extrinsic association with different proteins. The proteins involved...
 03:00
Molecular Chaperones and Protein Folding
The...
 00:59
Mechanisms of Membrane Domain Formation
Another mechanism for membrane domain formation involves membrane proteins interacting with...
 01:37
Energy to Drive Translocation
Generally, polypeptides are unfolded by two distinct...