Related Experiment Video
Updated: Aug 16, 2025

Imaging Spatial Reorganization of a MAPK Signaling Pathway Using the Tobacco Transient Expression System
Published on: March 20, 2016
Brassinosteroid signals cooperate with katanin-mediated microtubule severing to control stamen filament elongation
Jie Wang1,2,3, Guangda Wang1,2, Weiwei Liu1,4
1State Key Laboratory of Plant Genomics, Institute of Microbiology, Chinese Academy of Sciences, Beijing, China.

Abstract:
Proper stamen filament elongation is essential for pollination and plant reproduction. Plant hormones are extensively involved in every stage of stamen development; however, the cellular mechanisms by which phytohormone signals couple with microtubule dynamics to control filament elongation remain unclear. Here, we screened a series of Arabidopsis thaliana mutants showing different microtubule defects and revealed that only those unable to sever microtubules, lue1 and ktn80.1234, displayed differential floral organ elongation with less elongated stamen filaments. Prompted by short stamen filaments and severe decrease in KTN1 and KTN80s expression in qui-2 lacking five BZR1-family transcription factors (BFTFs), we investigated the crosstalk between microtubule severing and brassinosteroid (BR) signaling. The BFTFs transcriptionally activate katanin-encoding genes, and the microtubule-severing frequency was severely reduced in qui-2. Taken together, our findings reveal how BRs can regulate cytoskeletal dynamics to coordinate the proper development of reproductive organs.
Related Concept Videos
 01:45
Destabilization of Microtubules
 01:25
Cell Signaling in Plants
 01:14
Generation of Straight or Branched Actin Filaments
Arp2/3 Complex
Arp2/3 complex is a seven-subunit complex consisting of two proteins similar to actin- Arp2 and Arp3, and five other subunits that help keep Arp2 and Arp3 inactive. When required, the complex is...
 01:19
Actin Filament Depolymerization
In F-actin, the ADF/cofilin proteins...
 02:57
Attachment of Sister Chromatids
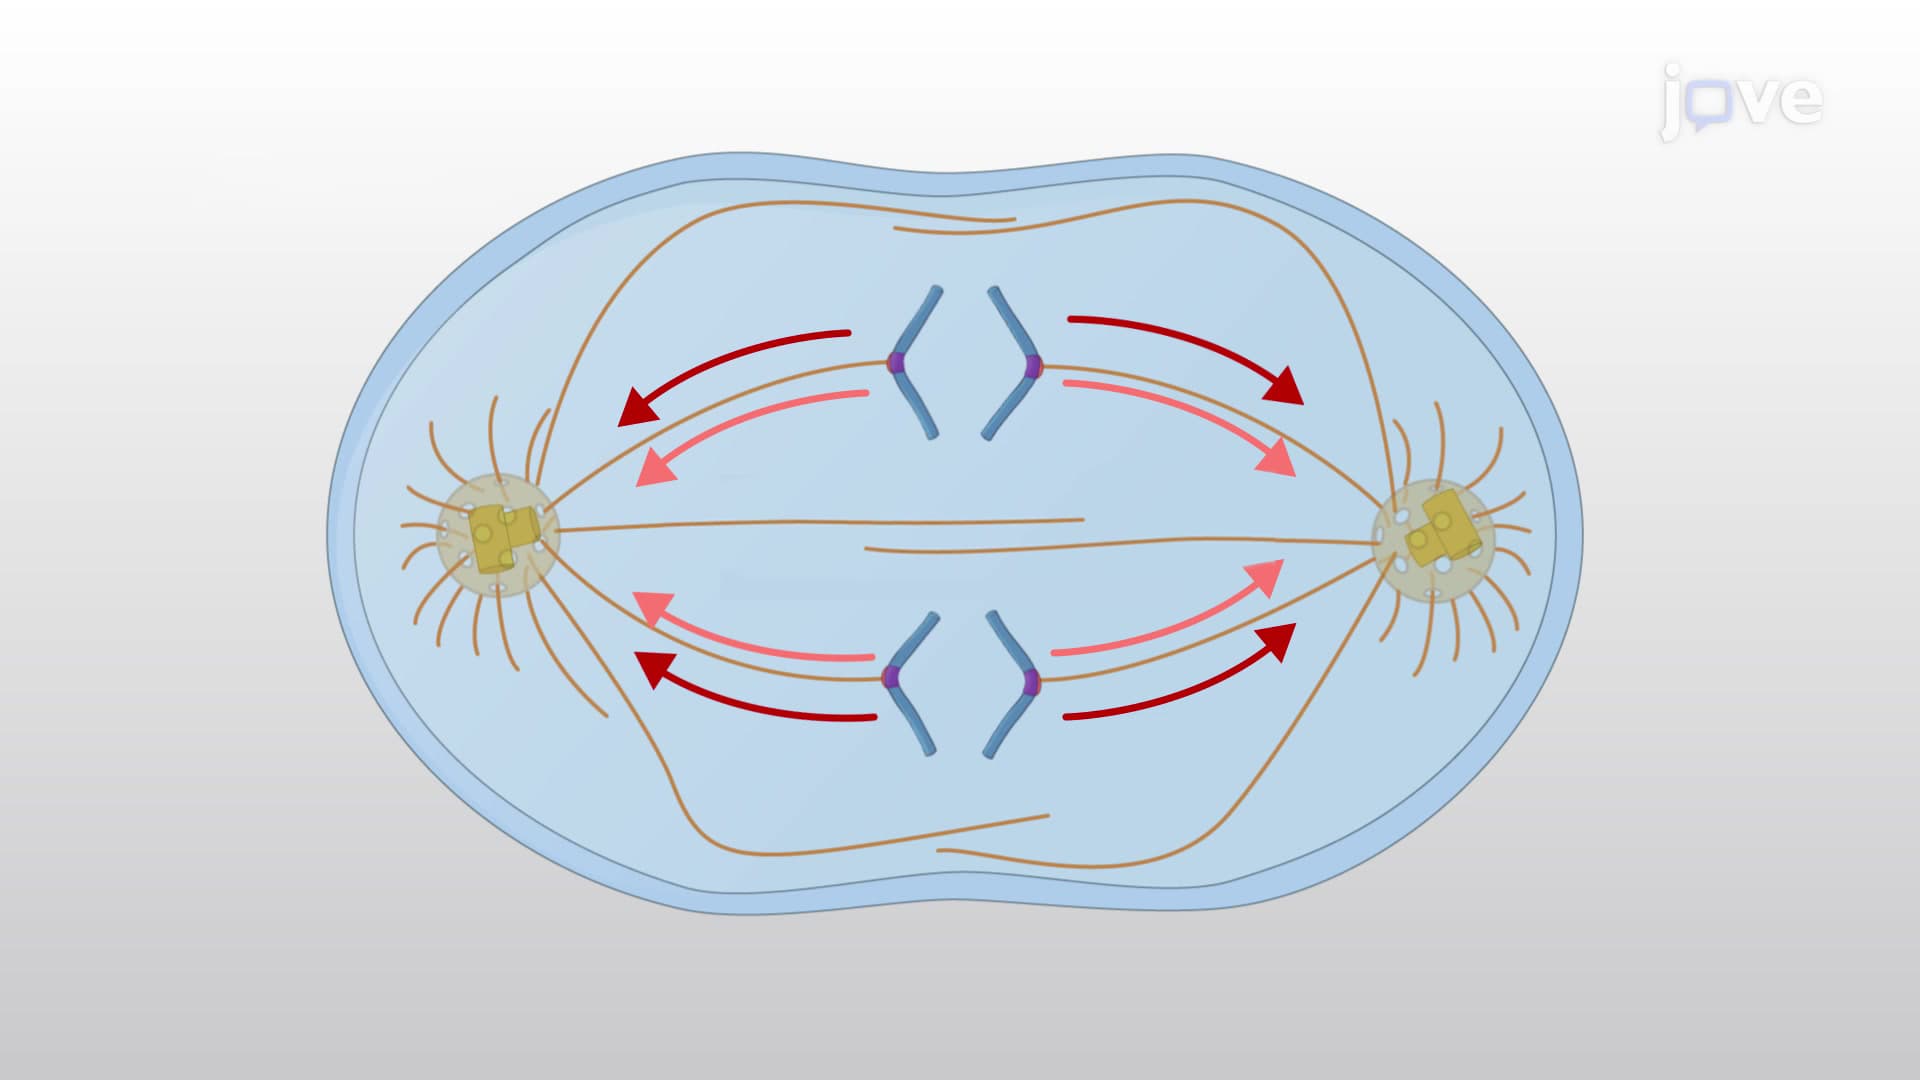 01:39
Anaphase A and B
Plus-end depolymerization releases tubulin heterodimers from the terminal region of the microtubule. As tubulin subunits are lost, the Ndc80 complexes detach...