Related Experiment Video
Updated: Jun 28, 2025
09:42

Using SecM Arrest Sequence as a Tool to Isolate Ribosome Bound Polypeptides
Published on: June 19, 2012
12.4K
Publisher Correction: The SecM arrest peptide traps a pre-peptide bond formation state of the ribosome
Felix Gersteuer1, Martino Morici1, Sara Gabrielli2
1Institute for Biochemistry and Molecular Biology, University of Hamburg, Martin-Luther-King-Platz 6, 20146, Hamburg, Germany.
Nature Communications
|April 16, 2024

Abstract
No abstract available in PubMed .
More Related Videos
Related Concept Videos
 01:34
Directing Proteins to the Rough Endoplasmic Reticulum
7.2K
The organelle-specific signaling sequences direct proteins synthesized in the cytosol to their final destination like ER, mitochondria, peroxisomes, etc. Some of the proteins directed to ER are then trafficked via vesicles to other organelles within the cell or the extracellular environment through the Golgi complex. For example, the rough ER synthesizes soluble proteins for transportation to the lysosomes or secretion out of the cell. It can also synthesize transmembrane proteins that can...
7.2K
 01:44
Termination of Translation
25.4K
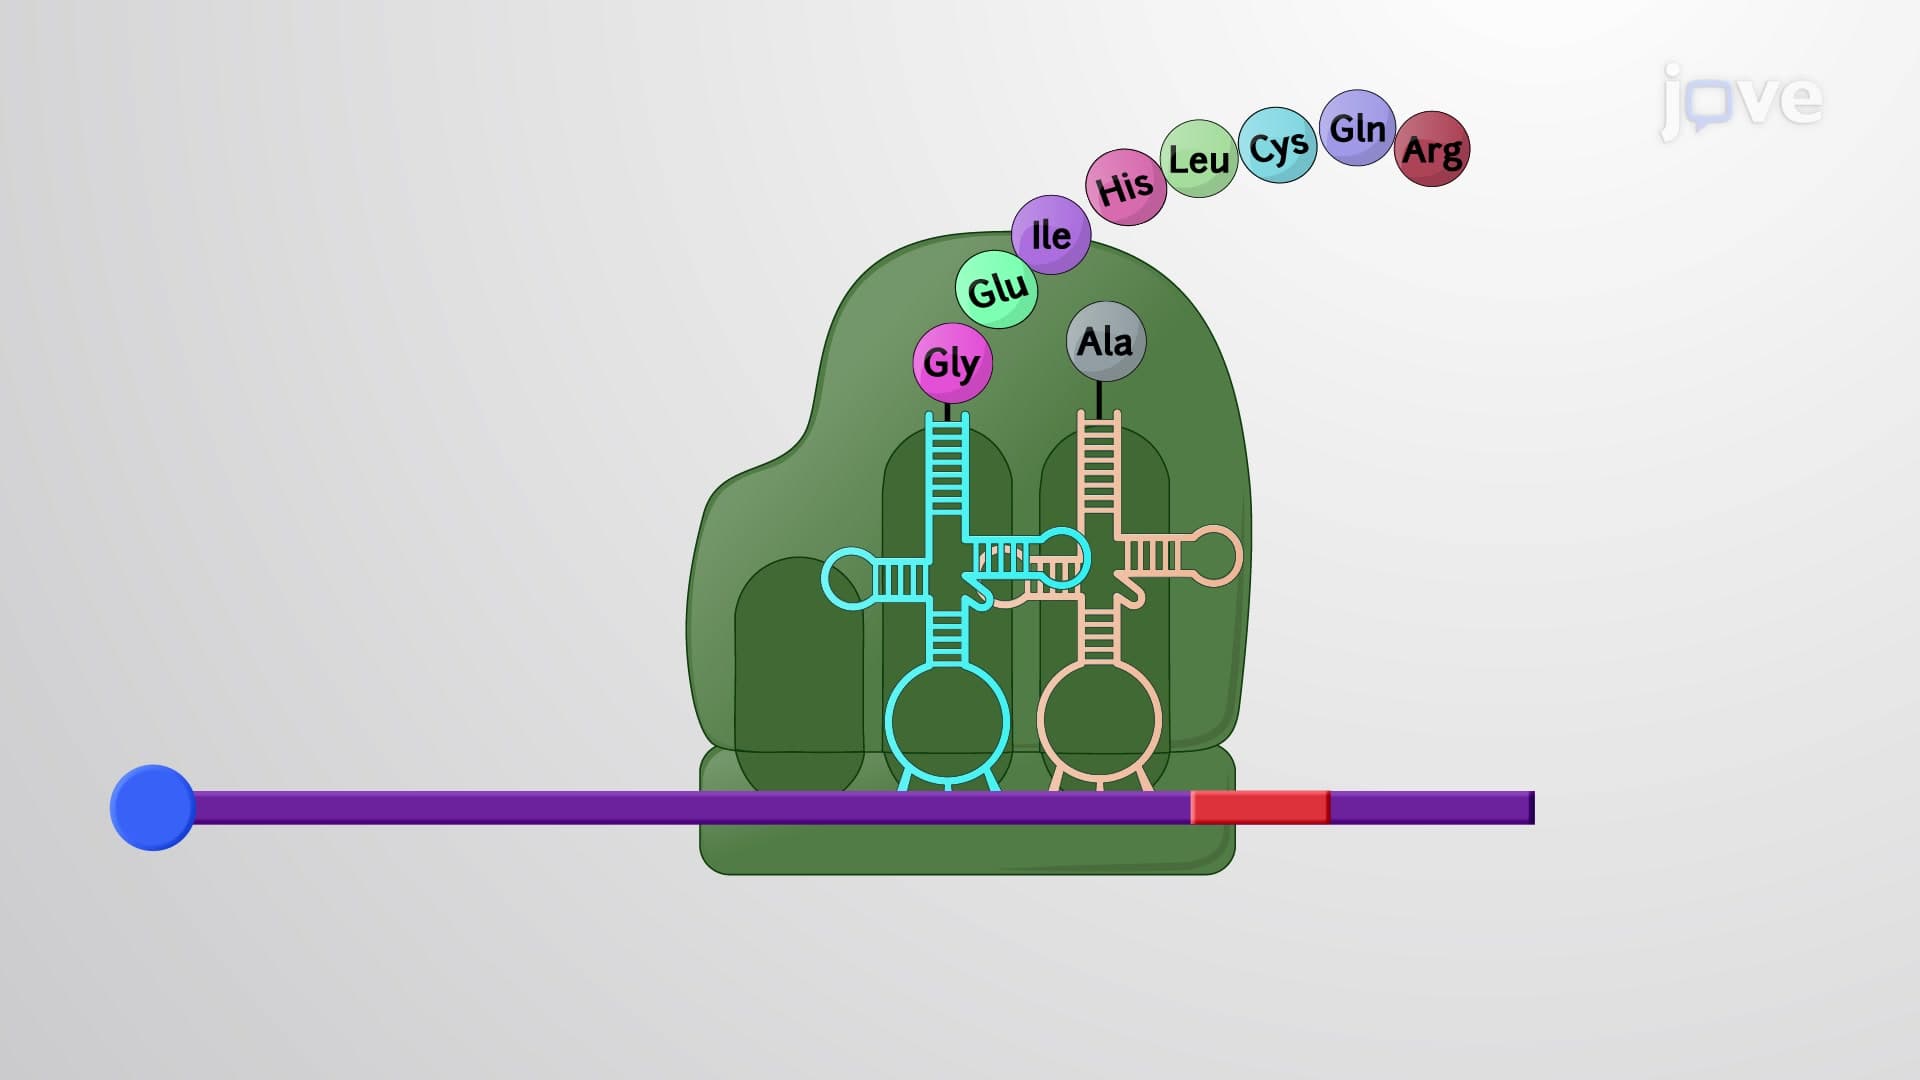
The large ribosomal subunit has several important structures essential to translation. These include the peptidyl transferase center (PTC) - which is the site where the peptide bond is formed - and a large, internal, water-filled tube through which the nascent polypeptide moves. This latter structure is called the Peptide Exit Tunnel, and it begins at the PTC and spans the body of the large ribosomal subunit. During translation, as the nascent polypeptide chain is synthesized, it passes through...
25.4K
 01:20
Cotranslational Protein Translocation
7.3K
Translocation of proteins across membranes is an ancient process that occurs even in bacteria and archaebacteria. In fact, the components of the translocation machinery are still conserved between prokaryotes and eukaryotes.
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
7.3K
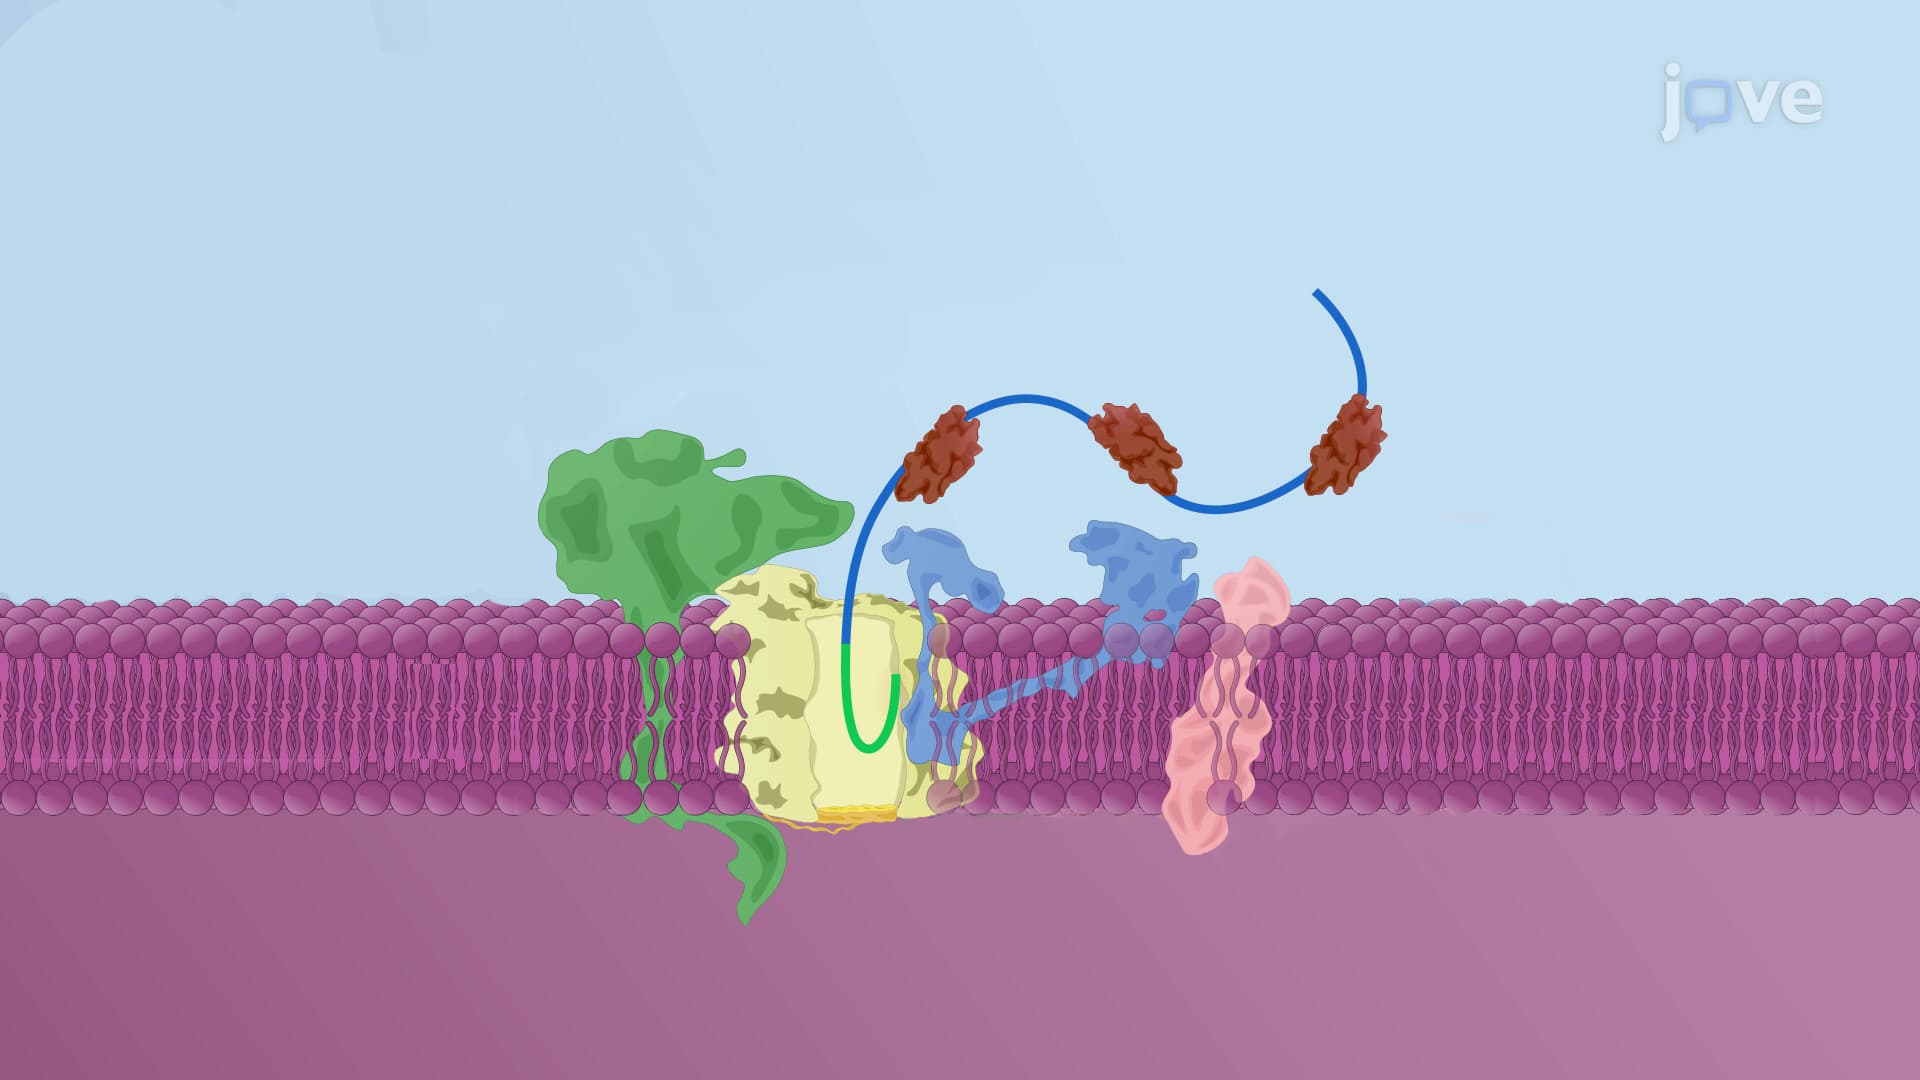 01:27
Post-translational Translocation of Proteins to the RER
5.7K
A sizable fraction of proteins destined for ER are first synthesized in the cell cytosol and then transported across the ER membrane–a process called post-translational translocation. Similar to cotranslationally translocated proteins, these proteins also use the Sec translocon complex to enter the ER lumen.
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
5.7K
 02:24
Ribosome Profiling
3.5K
Ribosome profiling or ribo-sequencing is a deep sequencing technique that produces a snapshot of active translation in a cell. It selectively sequences the mRNAs protected by ribosomes to get an insight into a cell’s translation landscape at any given point in time.
Applications of ribosome profiling
Ribosome profiling has many applications, including in vivo monitoring of translation inside a particular organ or tissue type and quantifying new protein synthesis levels.
The technique...
Applications of ribosome profiling
Ribosome profiling has many applications, including in vivo monitoring of translation inside a particular organ or tissue type and quantifying new protein synthesis levels.
The technique...
3.5K
 02:07
Improving Translational Accuracy
10.3K
Base complementarity between the three base pairs of mRNA codon and the tRNA anticodon is not a failsafe mechanism. Inaccuracies can range from a single mismatch to no correct base pairing at all. The free energy difference between the correct and nearly correct base pairs can be as small as 3 kcal/ mol. With complementarity being the only proofreading step, the estimated error frequency would be one wrong amino acid in every 100 amino acids incorporated. However, error frequencies observed in...
10.3K