Related Experiment Video
Updated: May 20, 2025

Using Scaffold Liposomes to Reconstitute Lipid-proximal Protein-protein Interactions In Vitro
Published on: January 11, 2017
Optimal functioning of the Lpt bridge depends on a ternary complex between the lipocalin YedD and the LptDE
Alexandra Gennaris1, Van Son Nguyen2, Laurie Thouvenel1
1WELBIO Department, WEL Research Institute, Avenue Pasteur, 6, 1300 Wavre, Belgium; de Duve Institute, Université catholique de Louvain (UCLouvain), Avenue Hippocrate 75, 1200 Brussels, Belgium.

Abstract:
The outer membrane is an efficient permeability barrier that protects gram-negative bacteria against external assaults, including many antibiotics. The unique permeability features of the outer membrane are due to the presence of lipopolysaccharide (LPS) molecules in its outer leaflet. LPS transport relies on the essential lipopolysaccharide transport (Lpt) pathway, which forms a bridge from the inner to the outer membrane. The LptDE translocon inserts LPS into the outer leaflet. Here, we identify the lipocalin YedD as a component of the translocon. Cryoelectron microscopy of the YedD-LptDE complex reveals that YedD binds LptD at a critical interface between its β-barrel and periplasmic β-taco domain. The YedD-LptDE complex is functionally relevant: under conditions where the connectivity of the β-taco and Lpt bridge is compromised, the absence of YedD decreases cell viability and causes LPS accumulation in the inner membrane. Our findings establish YedD as an Lpt component required for optimal LPS transport.
More Related Videos
 12:25
Isolation of Physiologically Active Thylakoids and Their Use in Energy-Dependent Protein Transport Assays
Published on: September 28, 2018
 10:59
Enrichment of Bacterial Lipoproteins and Preparation of N-terminal Lipopeptides for Structural Determination by Mass Spectrometry
Published on: May 21, 2018
Related Concept Videos
 01:28
Protein Translocation Machinery on the ER Membrane
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the...
 01:20
Cotranslational Protein Translocation
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
 01:27
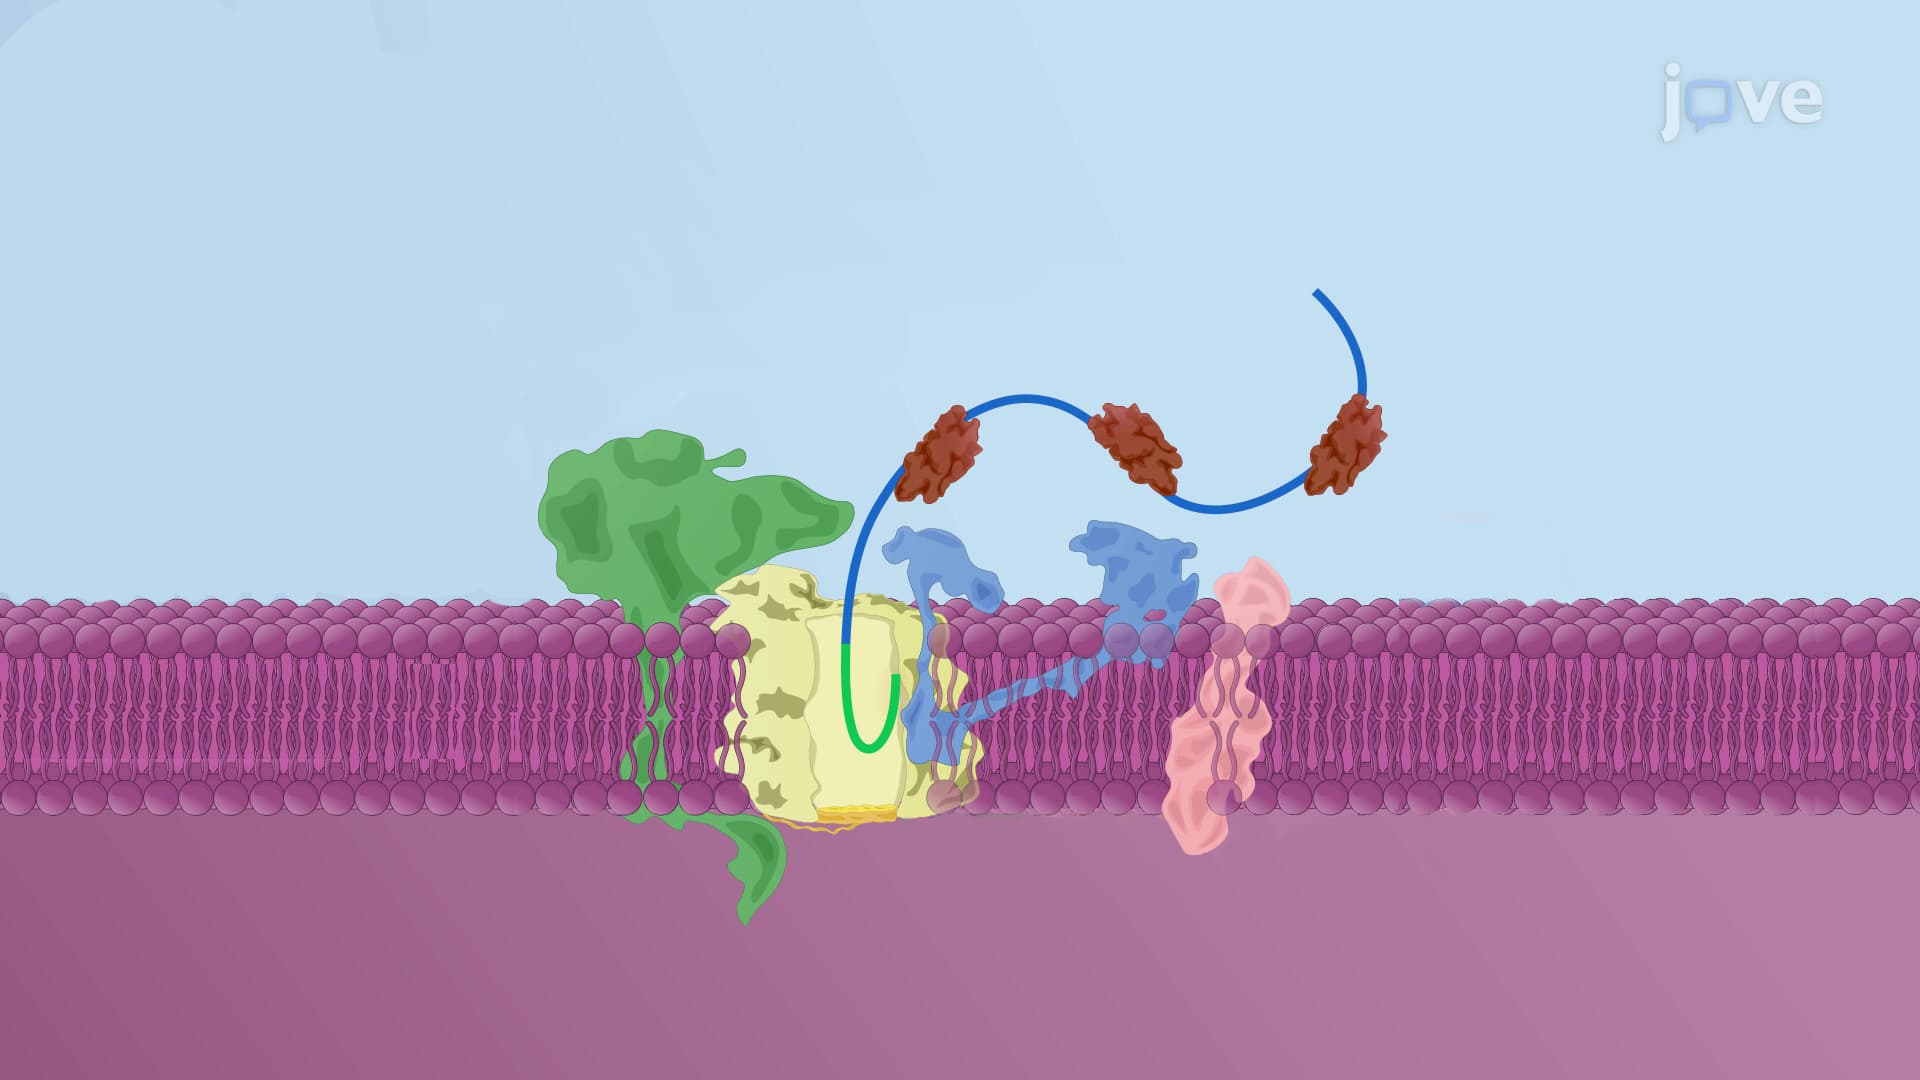
Post-translational Translocation of Proteins to the RER
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
 01:21
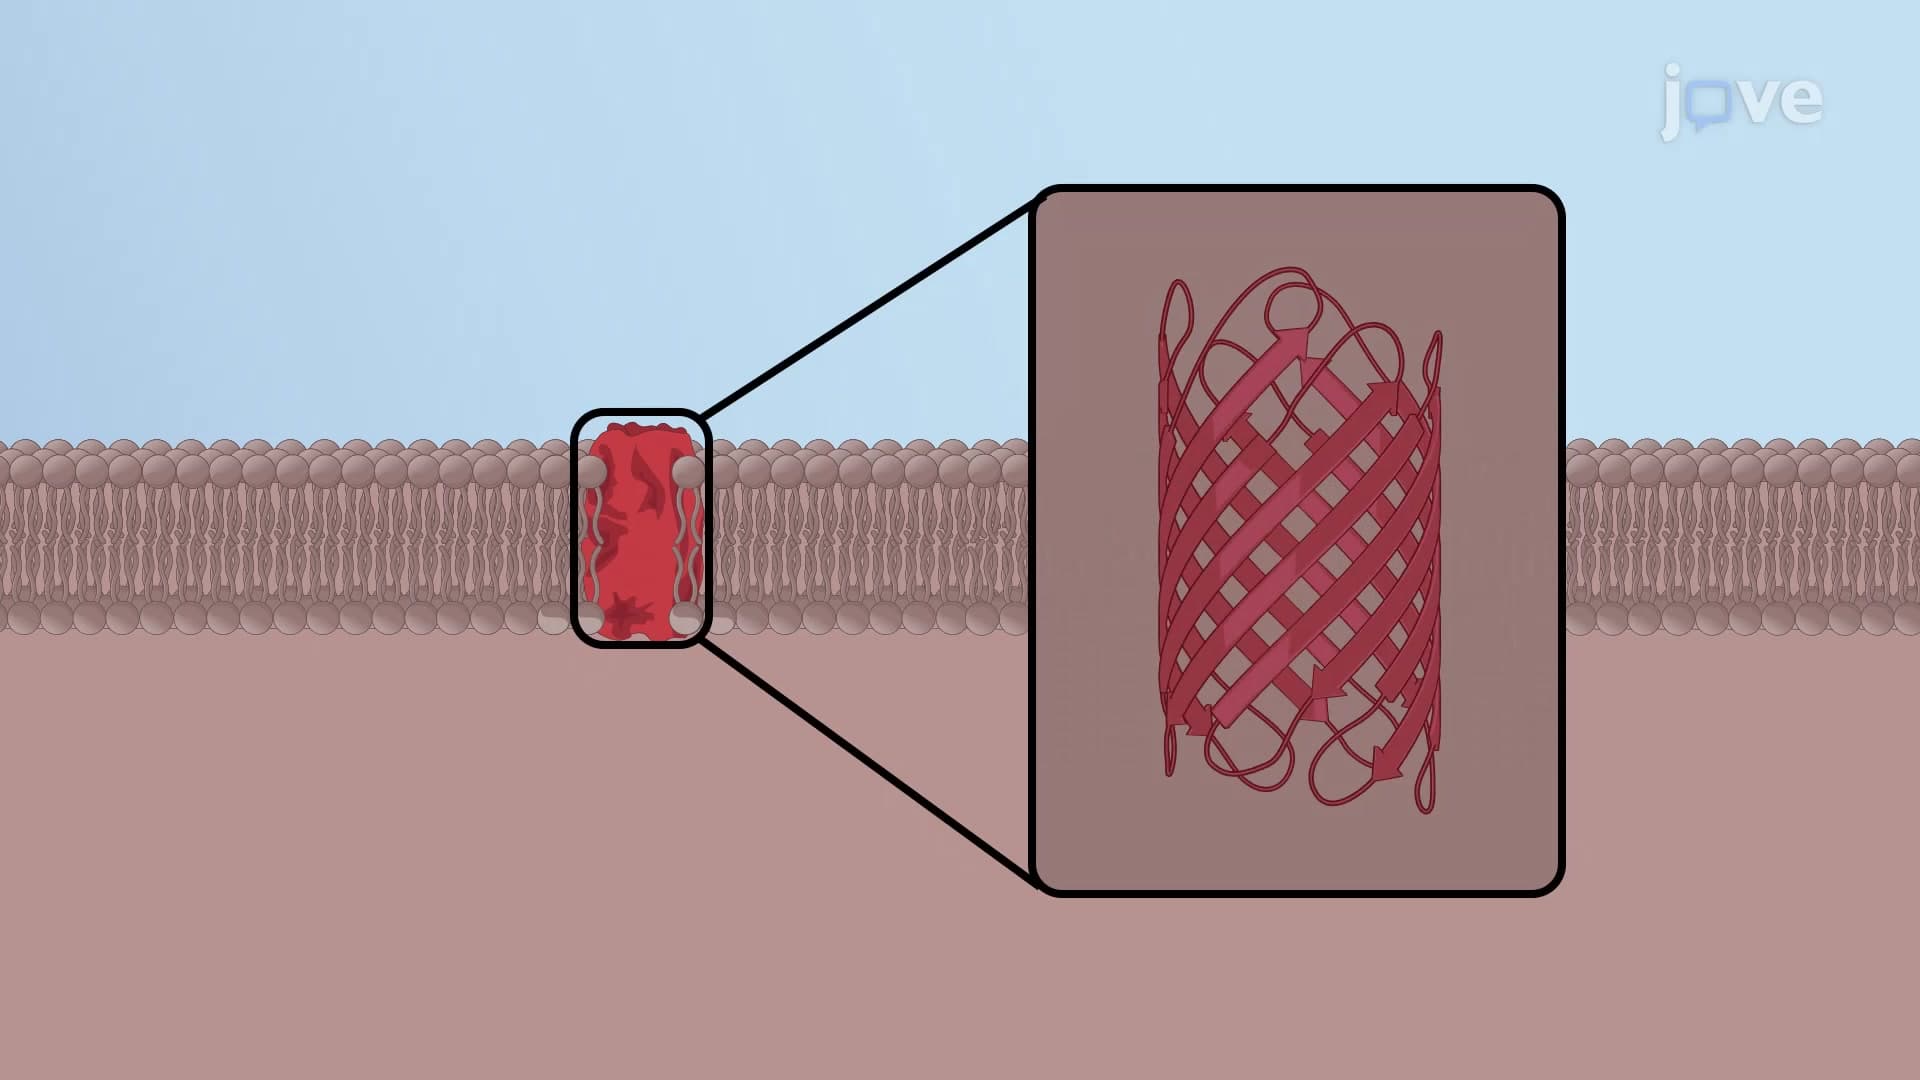
Structure of Porins
 01:45
Regulation of Nuclear Protein Sorting
 01:29
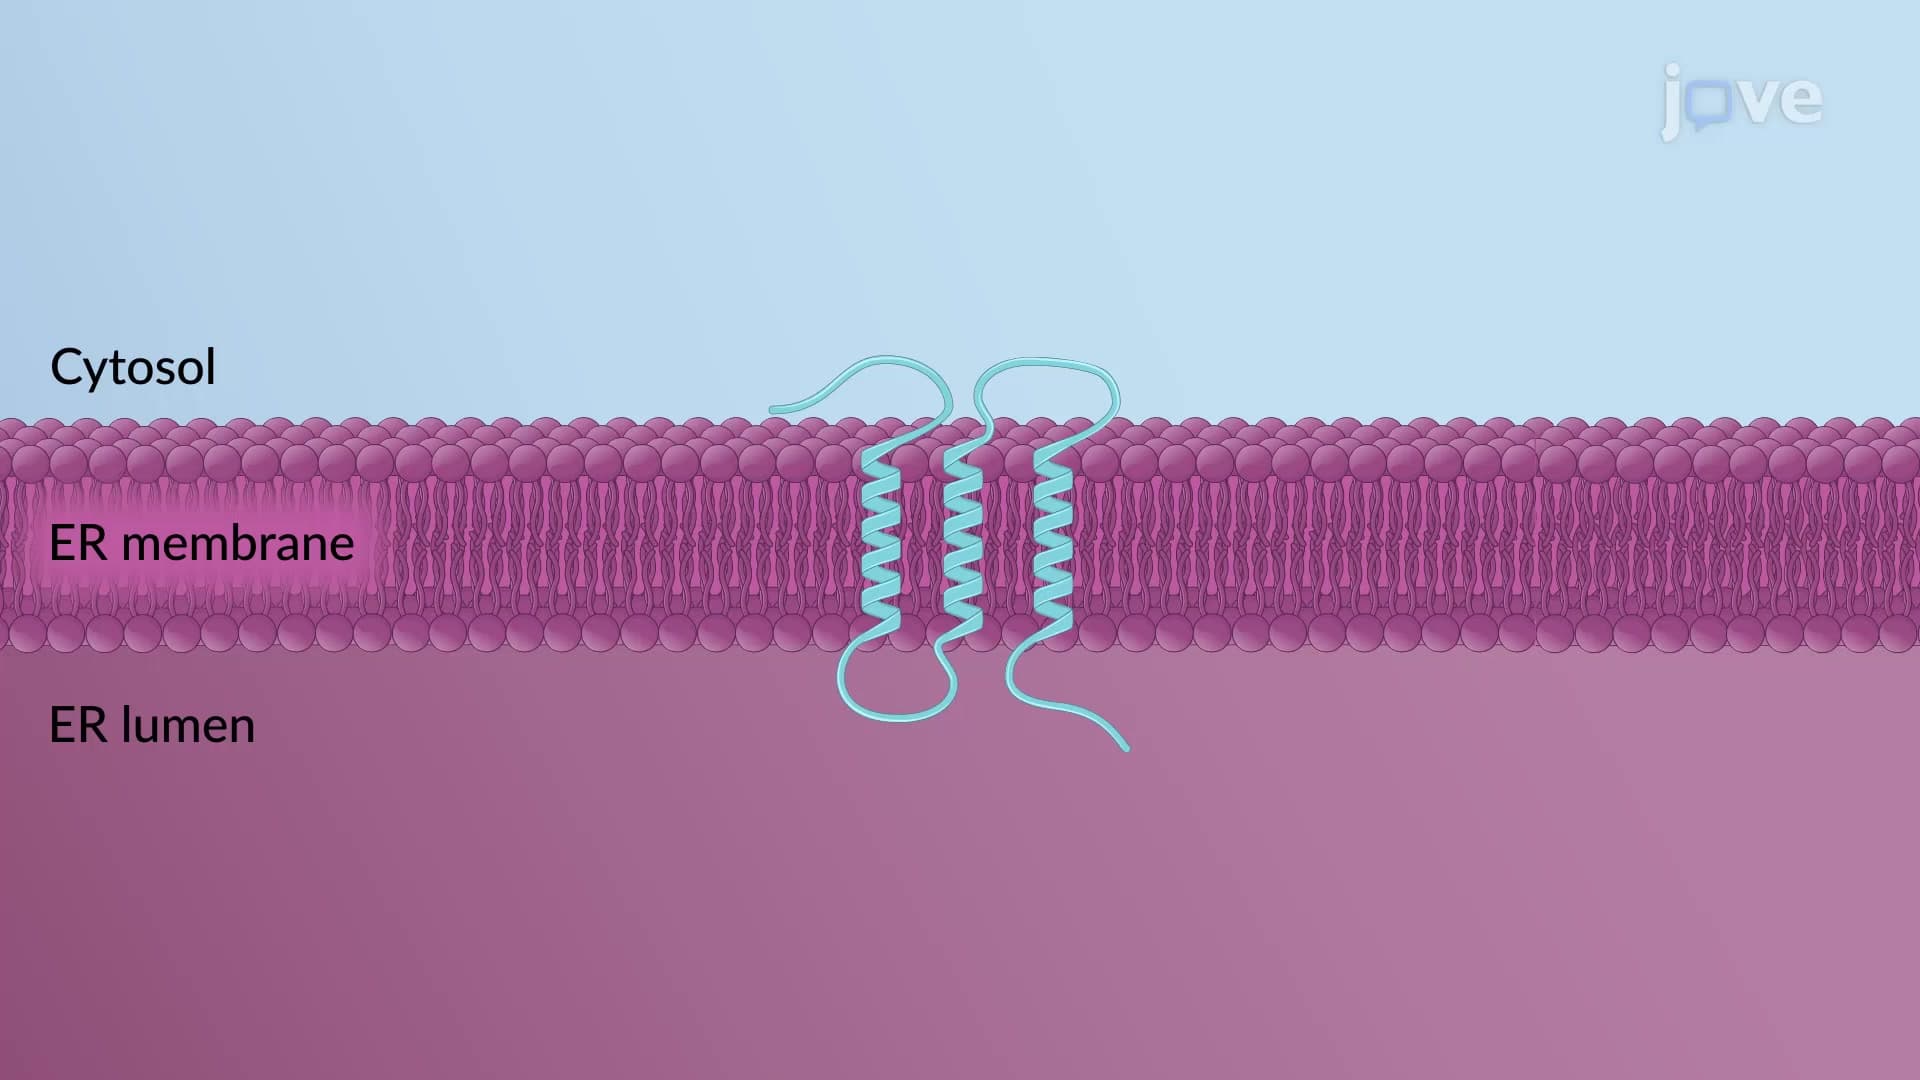
Insertion of Multi-pass Transmembrane Proteins in the RER
The multipass transmembrane proteins are the type IV integral membrane proteins with multiple topogenic sequences determining their spatial arrangement in the ER membrane. Nearly all multipass proteins lack a cleavable signal sequence and use...