Related Experiment Video
Updated: Mar 27, 2026

Flow Cytometric Analysis of Biomarkers for Detecting Human Sperm Functional Defects
Published on: April 21, 2022
Heat exposure during susceptible windows of spermatogenesis and sperm epigenetic age
Carrie Nobles1, Timothy P Canty2, Pauline Mendola3
1Department of Environmental Health Sciences, School of Public Health and Health Sciences, University of Massachusetts Amherst, Amherst, MA, USA.

Study Question:
Does preconception exposure to outdoor heat stress during spermatogenesis alter sperm epigenetic age among men from an infertility treatment population?
Summary Answer:
Exposure to outdoor heat stress during the developmental stages of mitosis and meiosis during spermatogenesis was associated with accelerated sperm epigenetic age.
What Is Known Already:
Spermatogenesis is uniquely susceptible to redox stress. Age-related disruption of the blood-testes barrier is associated with changes in sperm DNA methylation linked to reduced fecundity and pregnancy complications. Preconception heat stress may cause similar disruptions in the sperm epigenome, providing a pathway through which high temperatures may impair men's reproductive health.
Study Design, Size, Duration:
We evaluated exposure to high ambient temperatures and sperm epigenetic age among 1,220 men residing along the Wasatch Front in Utah in an ancillary prospective cohort study set within the Folic Acid and Zinc Supplementation Trial (FAZST; 2013-2018).
Participants/Materials, Setting, Methods:
Sperm epigenetic age (SEA), the acceleration or deceleration of age-related changes in sperm DNA methylation, was calculated in semen samples collected 6 months after enrollment. Utilizing local hourly temperature data, average temperature and hours per day exceeding the 98th, 95th, 90th, and 75th percentile thresholds for dry bulb temperature (ambient air) and wet bulb temperature (relative temperature with 100% humidity) were calculated across spermatogenesis and susceptible windows of mitosis, meiosis I + II, spermiogenesis, and spermiation. Temperature was modeled using three approaches: (i) Generalized linear models (GLMs) for average temperature by warm vs. cold season, (ii) GLMs incorporating natural cubic splines for average temperature, and (iii) GLMs for temperature thresholds.
Main Results And The Role Of Chance:
Across spermatogenesis, each additional 10% increase in proportion of time exposed to wet bulb temperatures ≥90th (16.1°C), ≥95th (17.2°C), and ≥98th (17.8°C) percentiles was associated with 0.063 (95% CI -0.001, 0.128), 0.121 (95% CI 0.022, 0.220), and 0.173 (95% CI 0.030, 0.316) years accelerated sperm epigenetic age, respectively. For spermatogenic-specific developmental windows, associations were strongest during meiosis I + II (e.g. 0.146 [95% CI 0.028, 0.264] years for ≥98th percentile) and, in spline models, both warmer and colder wet bulb temperatures during meiosis I + II were associated with accelerated sperm epigenetic age (P = 0.028). Associations for dry bulb temperatures were similar, although less precise, and no clear associations were observed when modeling average temperature by season.
Limitations, Reasons For Caution:
Due to reliance on outdoor temperatures rather than personal exposure, misclassification of exposure to temperature is likely. Findings should be generalized with caution to groups with different levels of exposure to and susceptibility to outdoor heat. While we observed modest effect sizes up to 0.173 years for accelerated SEA per 10% increased time exposed to heat conditions, these changes at the population-level may be impactful for downstream impacts on fertility and pregnancy health, and future work replicating and extending findings is an important next step.
Wider Implications Of The Findings:
Associations between high wet bulb temperatures, which capture impaired efficiency of sweating for cooling body temperature, and accelerated epigenetic aging add evidence that heat-related disruption of sperm DNA methylation may adversely impact men's reproductive health.
Study Funding/Competing Interest(S):
This study was supported by K01ES034005 from the National Institute of Environmental Health Sciences. The parent trial was supported by funding from the Intramural Research Program of the Eunice Kennedy Shriver National Institute of Child Health and Human Development (HHSN275201200007C and HHSN275201300026I).The authors have no conflicts of interest to declare.
Trial Registration Number:
NCT01857310.
More Related Videos
 05:55
Stable Isotope In-Vivo Labeling for Mass-Spectrometry Identification of Paternal Metabolites Transferred from Sperm to Oocyte During Fertilization
Published on: June 17, 2025
 10:24
Evaluation of Intracellular Location of Reactive Oxygen Species in Solea Senegalensis Spermatozoa
Published on: March 11, 2018
Related Concept Videos
 01:41
Spermatogenesis
 01:22
Spermatogenesis
The process of spermatogenesis can be divided into mitosis, meiosis, and spermiogenesis. During mitosis, the spermatogonia or stem cells divide to produce two identical daughter cells, type A and B spermatogonia. Type-A...
 01:35
Mutations
Chromosomal Alterations Are Large-Scale Mutations
While point mutations are changes in a single nucleotide in...
 01:39
Mutations
 03:09
Meiosis I
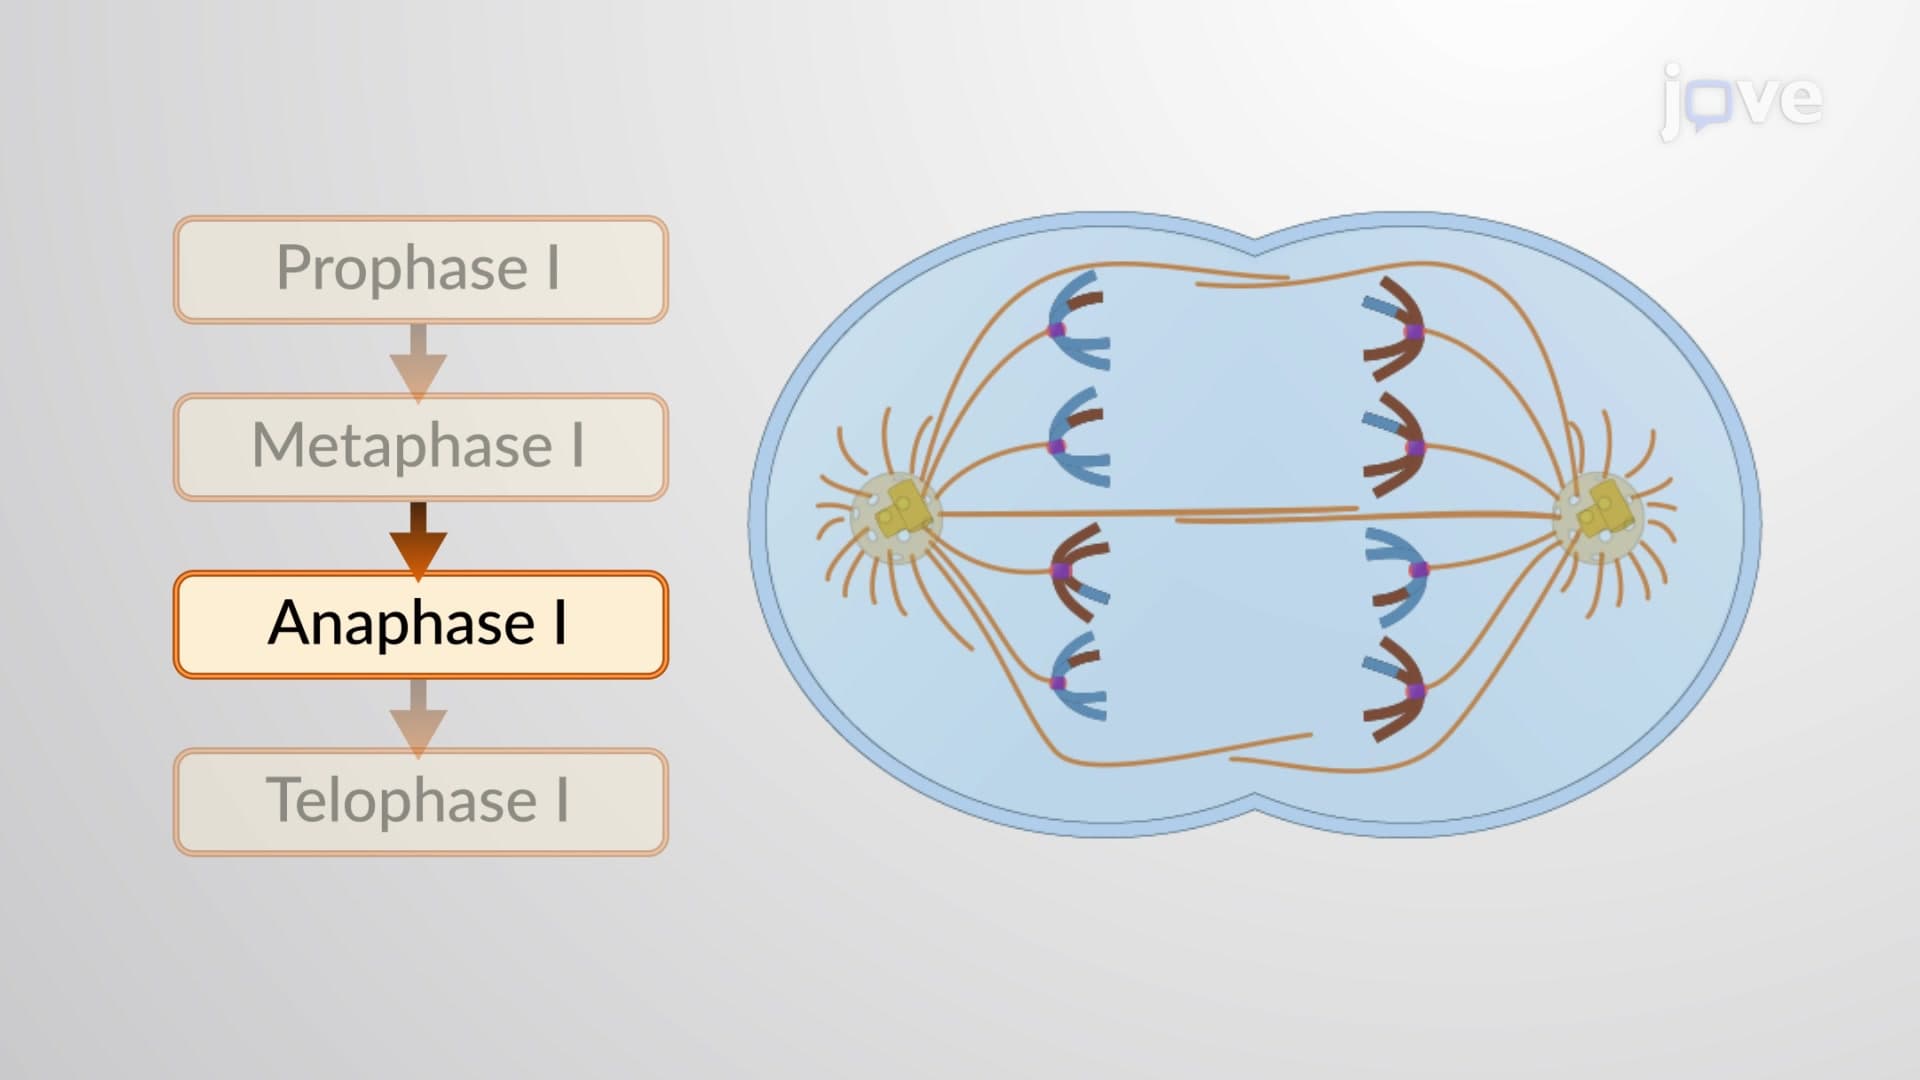
Prophase I is the most extended and complex step of meiosis I characterized by synapsis, chromosome pairing, and recombination of the homologous chromosomes. This process is facilitated by a proteinaceous structure called the...
 02:27
Background and Environment Affect Phenotype
An example of how genetic background affects phenotype can be seen in horses. The Extension gene in horses is responsible for their coat color. A wild-type gene (EE) produces black pigment in the coat, while a mutant gene (ee) produces red pigment. A...