Related Experiment Video
Updated: Aug 13, 2026
X-Ray Crystallography to Study the Oligomeric State Transition of the Thermotoga maritima M42 Aminopeptidase TmPep1050
Published on: May 13, 2020
The zinc metalloprotease ZMPSTE24 binds a distinct topological isoform of the tail-anchored protein IFITM3
Eric D Spear1, Khurts Shilagardi1, Sonia Sarju1
1Department of Cell Biology, The Johns Hopkins School of Medicine, Baltimore, Maryland, USA.

Abstract:
The biogenesis of integral membrane proteins is complex, as revealed by an ever-growing number of cellular components dedicated to the insertion, folding, surveillance, rectification, or quality control of specific client membrane proteins. The zinc metalloprotease ZMPSTE24 and its yeast homolog Ste24 have well-established roles in the proteolytic maturation of the nuclear scaffold protein lamin A and yeast a-factor, respectively. Additionally, Ste24 has been implicated through yeast genetic screens in a variety of membrane processes, including ER-associated degradation, Sec61 translocon "unclogging," and potentially as a membrane protein topology determinant. Recently, an interaction was demonstrated between ZMPSTE24 and the antiviral interferon induced transmembrane protein IFITM3, although the functional significance of this interaction is poorly understood. IFITM3 is a tail-anchored protein with a cytoplasmic N-terminus, a single transmembrane span, and a lumenal/exocellular C-terminus. Here, we show that a catalytic-dead version of ZMPSTE24, ZMPSTE24E336A, exhibits enhanced binding to IFITM3, and this bound species of IFITM3 is hypo-palmitoylated. Using a split fluorescence topology reporter, we demonstrate that ZMPSTE24E336A "traps" and stabilizes a subpopulation of IFITM3 molecules with an atypical membrane topology, whose C-terminus is cytosolic instead of lumenal. Such inverted forms of IFITM3 are also detected in the presence of ER-associated degradation inhibitors or for a lysineless version of IFITM3. We hypothesize the ZMPSTE24E336A trap mutant reveals a normally transient isoform of IFITM3 whose transmembrane span is inverted and that ZMPSTE24 is involved in the quality control of IFITM3 topology, either inverting, correcting or assisting in removal of aberrant IFITM3 molecules.
Related Concept Videos
 01:45
Tail-anchoring of Proteins in the ER Membrane
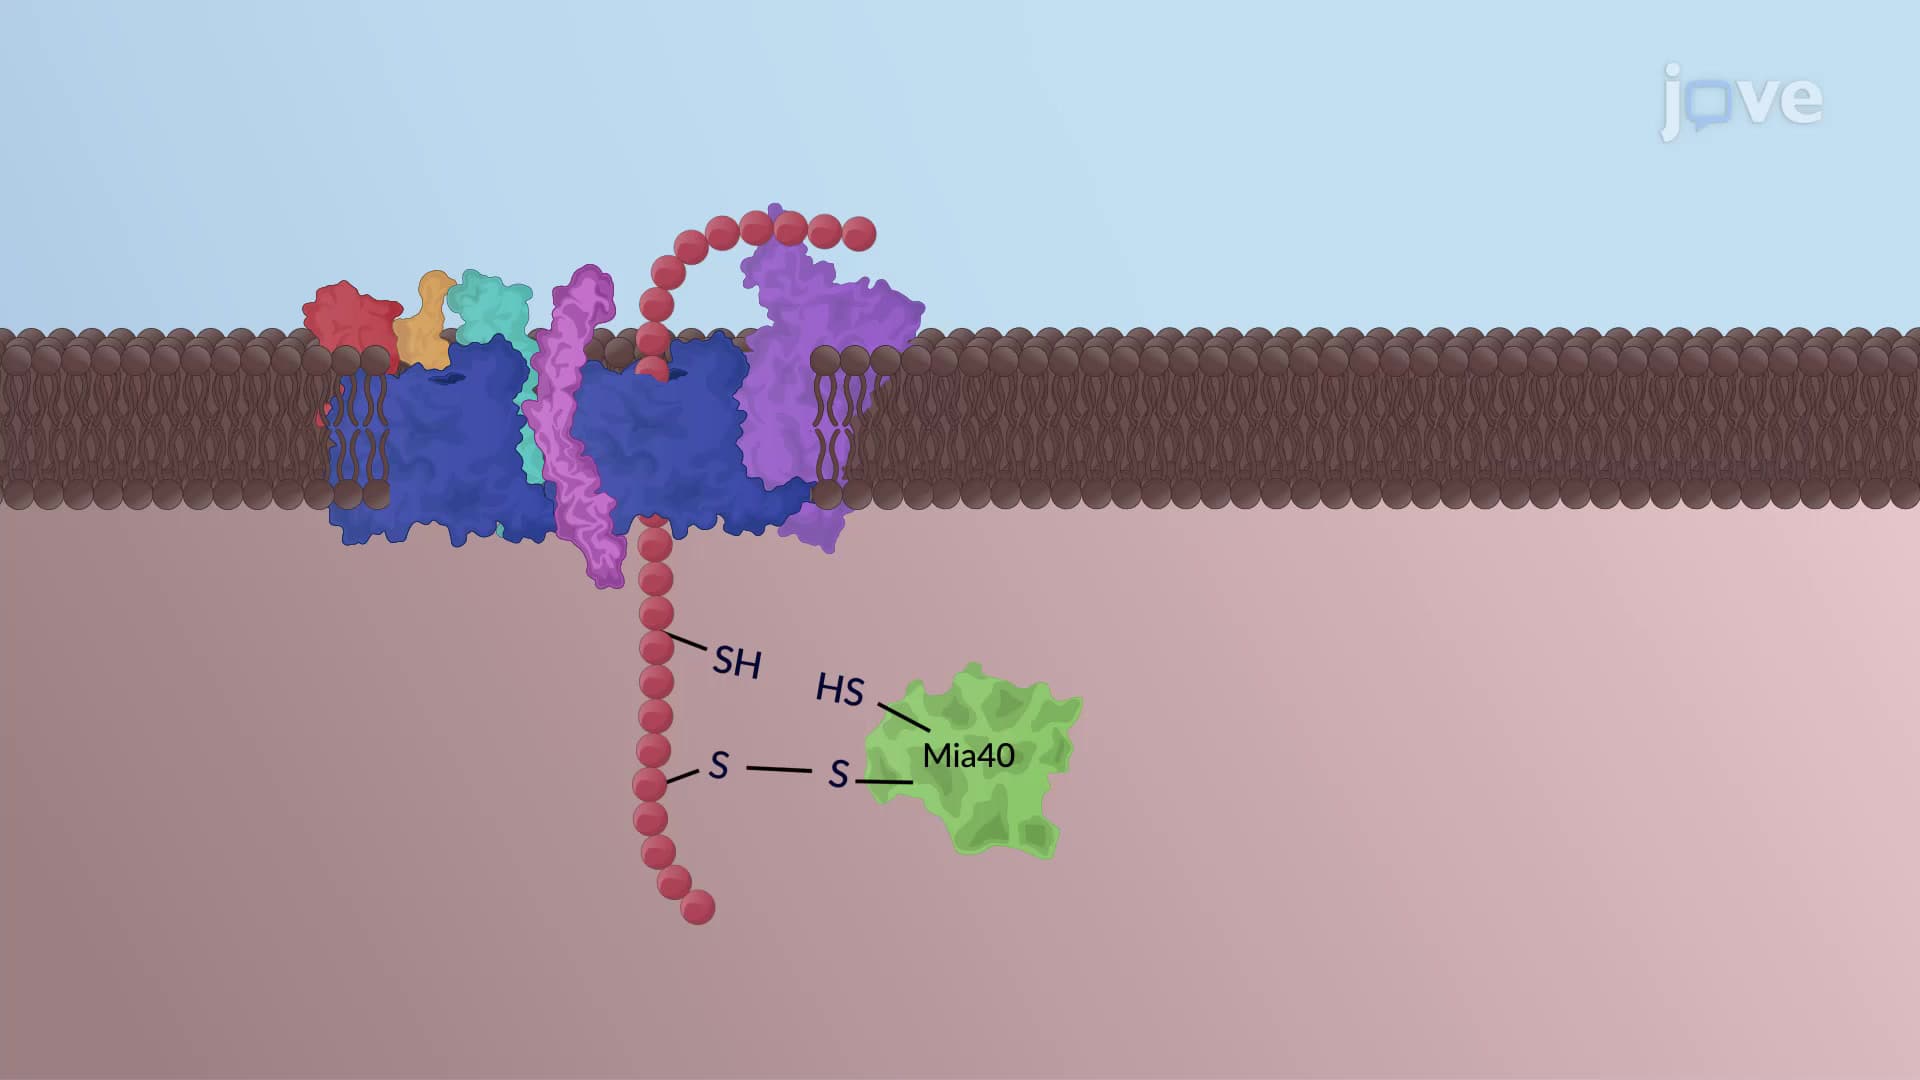 01:19
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:34
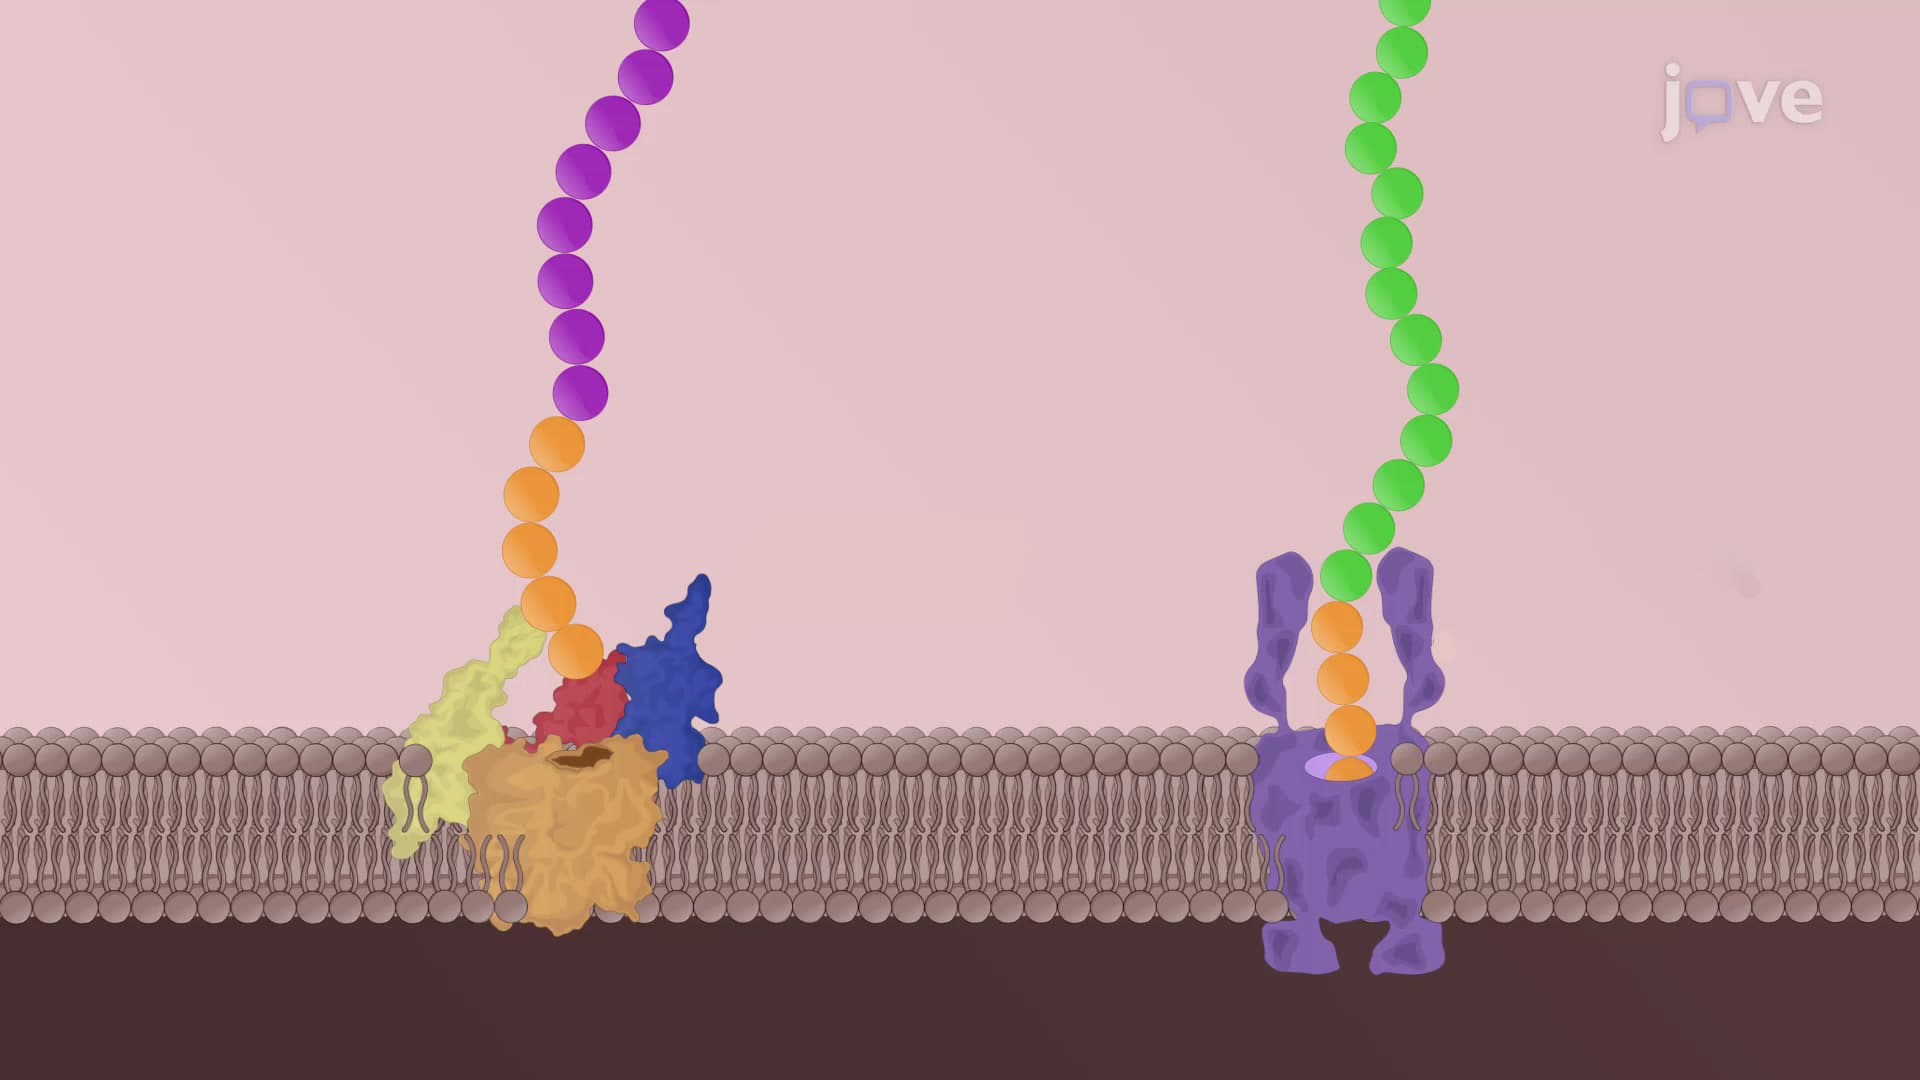
Protein Transport into the Inner Mitochondrial Membrane
Transport of mitochondrial precursors across the TIM23 channel is driven by...
 01:21
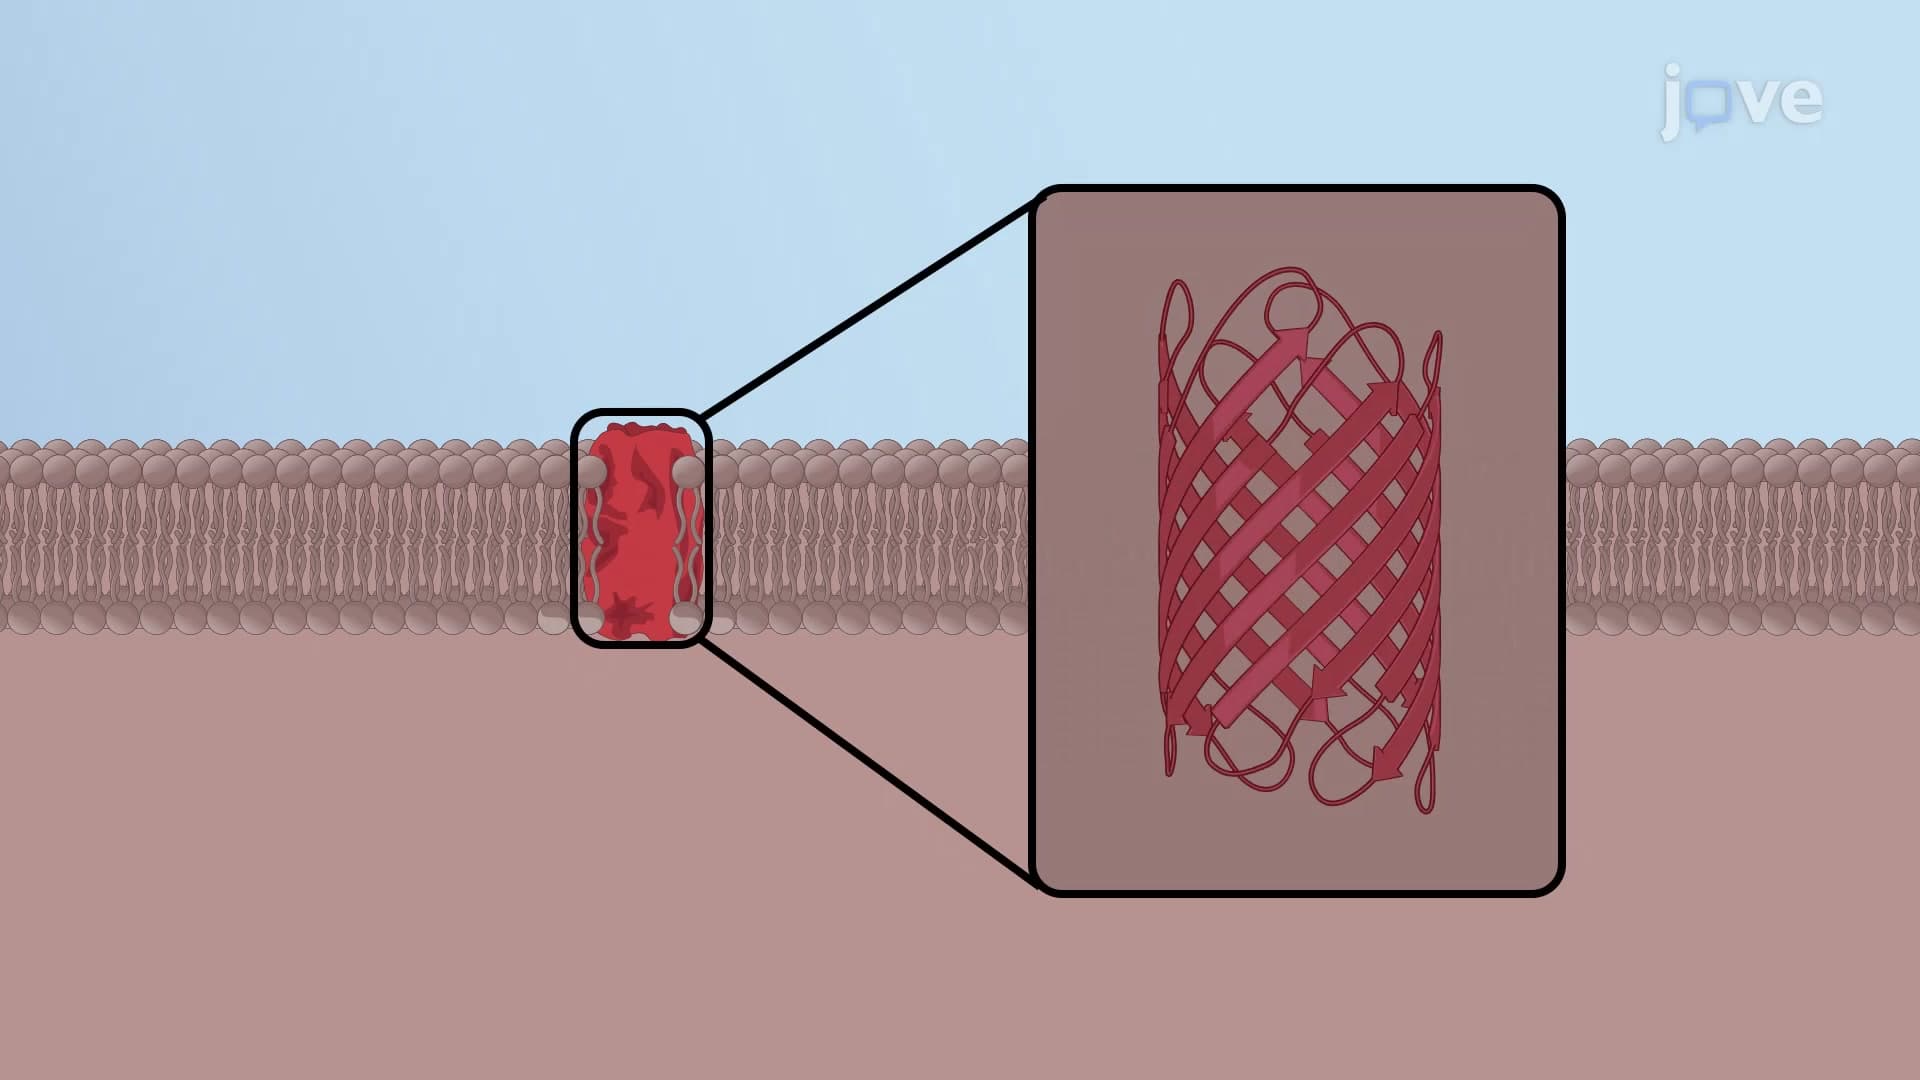
Structure of Porins
 01:15
Activation of Integrins
In "outside-in signaling," external factors in the extracellular space bind to exposed ligand binding sites on integrins. This causes the inactive protein to undergo a conformational change to become active. Integrins are often clustered on the cell membrane. Repetitive and regularly spaced ligand binding events provide an effective stimulus.
 01:17
Intracellular Signaling Affects Focal Adhesions
Some...