Related Experiment Video
Updated: Sep 19, 2026

Measuring Enzymatic Activity of Neurodevelopmental Disorder-Associated Deubiquitylating Enzymes via an In Vitro Ubiquitin Chain Cleavage Assay
Published on: September 27, 2024
Tied to Work: Topologically Knotted SPOUT Methyltransferases and UCH Deubiquitinases in Cellular Biochemistry
Shang-Te Danny Hsu1,2,3,4
1Institute of Biological Chemistry, Academia Sinica, Taipei, Taiwan.

Abstract:
Topologically knotted proteins are emerging as functional elements of the proteome rather than structural curiosities. Among the recurring protein knot types, the 31 trefoil, 52 Gordian and 71 septoil knots provide useful models for understanding how topology may reshape catalysis, substrate recognition, folding and mechanical behaviour. This review focuses on two systems in which these links can already be made with unusual clarity: the 31-knotted SPOUT methyltransferase superfamily and the 52-knotted ubiquitin C-terminal hydrolases (UCHs). In SPOUT methyltransferases, the knot defines a compact S-adenosyl-l-methionine (SAM)-binding pocket and enforces the bent cofactor geometry required for efficient methyl transfer. In UCH deubiquitinases, the 52 knot stabilises catalytic architecture, constrains the crossover loop that gates substrate access, and helps explain how mutations, regulatory elements and disease-linked perturbations alter function. Beyond catalysis, knotted topology may also modulate how some proteins respond to force, although the range of mechanostabilities across the knotted proteome is broad and many knotted proteins show moderate resistance to mechanical unfolding. Comparisons between 52-knotted UCH paralogs and the 71-knotted protein Q9PR55 raise the possibility that knot geometry contributes to resilience to withstand vectorial pulling, that is, mechanical unfolding, by a AAA+ protease, ClpXP, alongside local folding stability. In the context of folding mechanisms, knotted proteins are challenging systems in that many populate long-lived intermediates or misthreaded states along parallel or bifurcated folding pathways. Although populated intermediates and slow folding are also well documented in numerous unknotted systems, the question of how knotted topologies contribute to the formation of folding intermediates together with knotting/threading events adds to an extra layer of complexity to the analyses. Together, these examples support a broader view in which topology is not merely descriptive geometry, but a mechanistic variable that links structure, dynamics and biological function.
Related Concept Videos
 02:04
Covalently Linked Protein Regulators
These groups modify specific amino acids in a protein.
 02:58
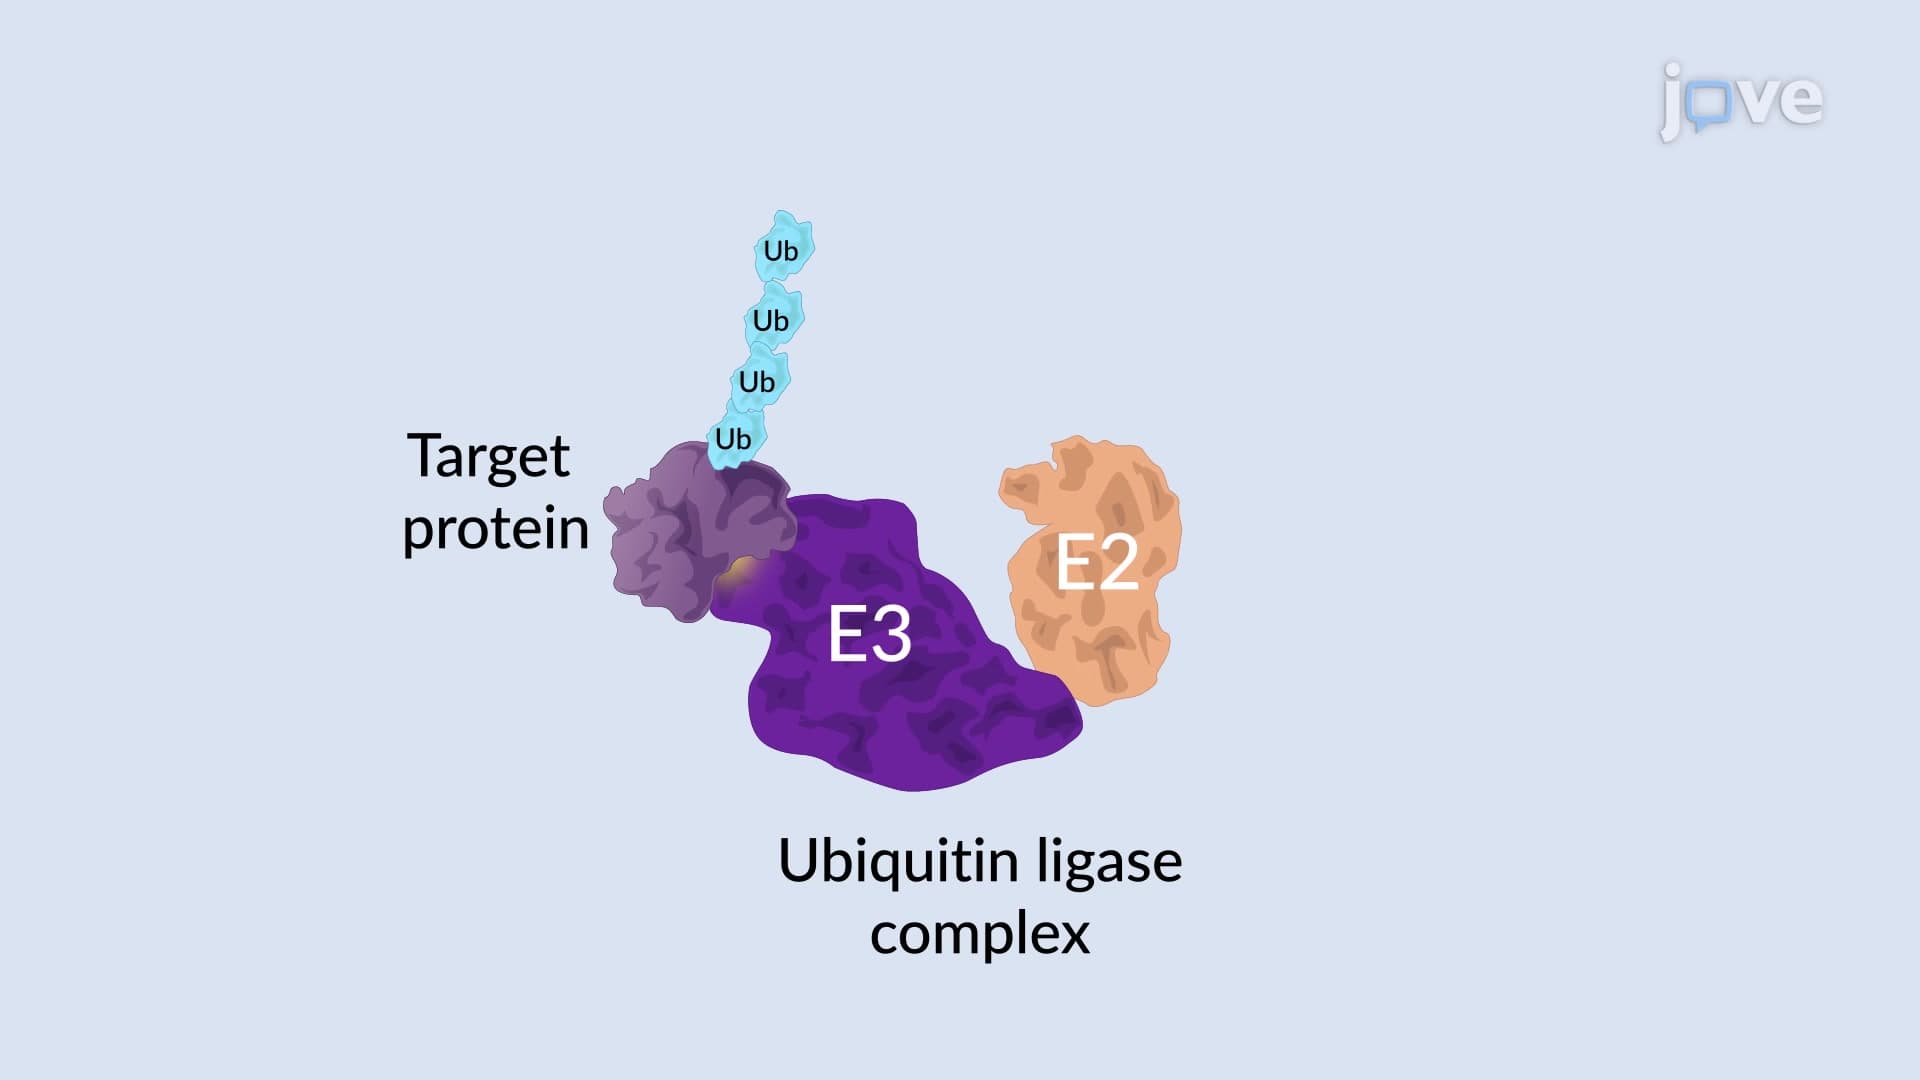
Regulated Protein Degradation
Protein degradation plays two important roles in the cells. It helps to protect cells from misfolded or damaged proteins before they lead to a...
 01:28
Biosynthesis of Nucleic Acids
 01:13
The Proteasome
In this pathway, the target proteins are first tagged with small proteins called ubiquitin. This involves participation of a series of enzymes including— E1 (ubiquitin-activating enzyme), E2 (ubiquitin-conjugating enzyme), and E3 (ubiquitin...
 02:18
The Proteasome
In this pathway, the target proteins are first tagged with small proteins called ubiquitin. A series of enzymes carry out the ubiquitination of the target proteins - E1 (ubiquitin-activating enzyme), E2 (ubiquitin-conjugating enzyme), and E3...
 01:26
Protein Modifications in the RER
Broadly, these modifications can be categorized into four main categories — glycosylation, formation of disulfide bonds, assembly of protein subunits, and specific proteolytic cleavages like removal of signal sequences.