Related Experiment Video
Updated: Sep 29, 2026

Functional Complementation Analysis (FCA): A Laboratory Exercise Designed and Implemented to Supplement the Teaching of Biochemical Pathways
Published on: June 24, 2016
Bifunctional architecture enables substrate catalysis and channeling in Paracoccus TMAO demethylase
Trung Thach1, KanagaVijayan Dhanabalan1, Shiwangi Maurya2
1Department of Biological Sciences, Purdue University, West Lafayette, United States.

Abstract:
Substrate channeling enhances efficiency and prevents toxicity by directing unstable intermediates between active sites. Trimethylamine N-oxide demethylase (TDM) degrades trimethylamine N-oxide (TMAO) to dimethylamine and formaldehyde (HCHO), but the fate of HCHO has remained unclear. We report cryo-EM structures of TDM in apo, substrate-, and product-bound states that reveal a previously unknown channeling pathway. Combined structural, biochemical, and target molecular dynamics analyses show that HCHO is generated in a catalytic core and guided through a tunnel to a remote tetrahydrofolate (THF)-binding site, where it forms methylene-THF. Thus, TDM emerges as a bifunctional enzyme that unites TMAO demethylation with one-carbon transfer, providing a mechanistic explanation for its role in metabolic efficiency and detoxification.
More Related Videos
 10:21
Expression, Purification, Crystallization, and Enzyme Assays of Fumarylacetoacetate Hydrolase Domain-Containing Proteins
Published on: June 20, 2019
 11:27
X-Ray Crystallography to Study the Oligomeric State Transition of the Thermotoga maritima M42 Aminopeptidase TmPep1050
Published on: May 13, 2020
Related Concept Videos
 01:19
Allosteric Proteins-ATCase
Aspartate transcarbamoylase (ATCase) is a cytosolic enzyme that catalyzes the condensation of L-aspartate and carbamoyl phosphate to N-carbamoyl-L-aspartate. This reaction is the first step in pyrimidine biosynthesis. UTP and CTP, the end products of the pyrimidine synthesis pathway,...
 01:07
Catalytically Perfect Enzymes
 01:18
Amino Acid Catabolism
 02:26
tRNA Activation
 01:21
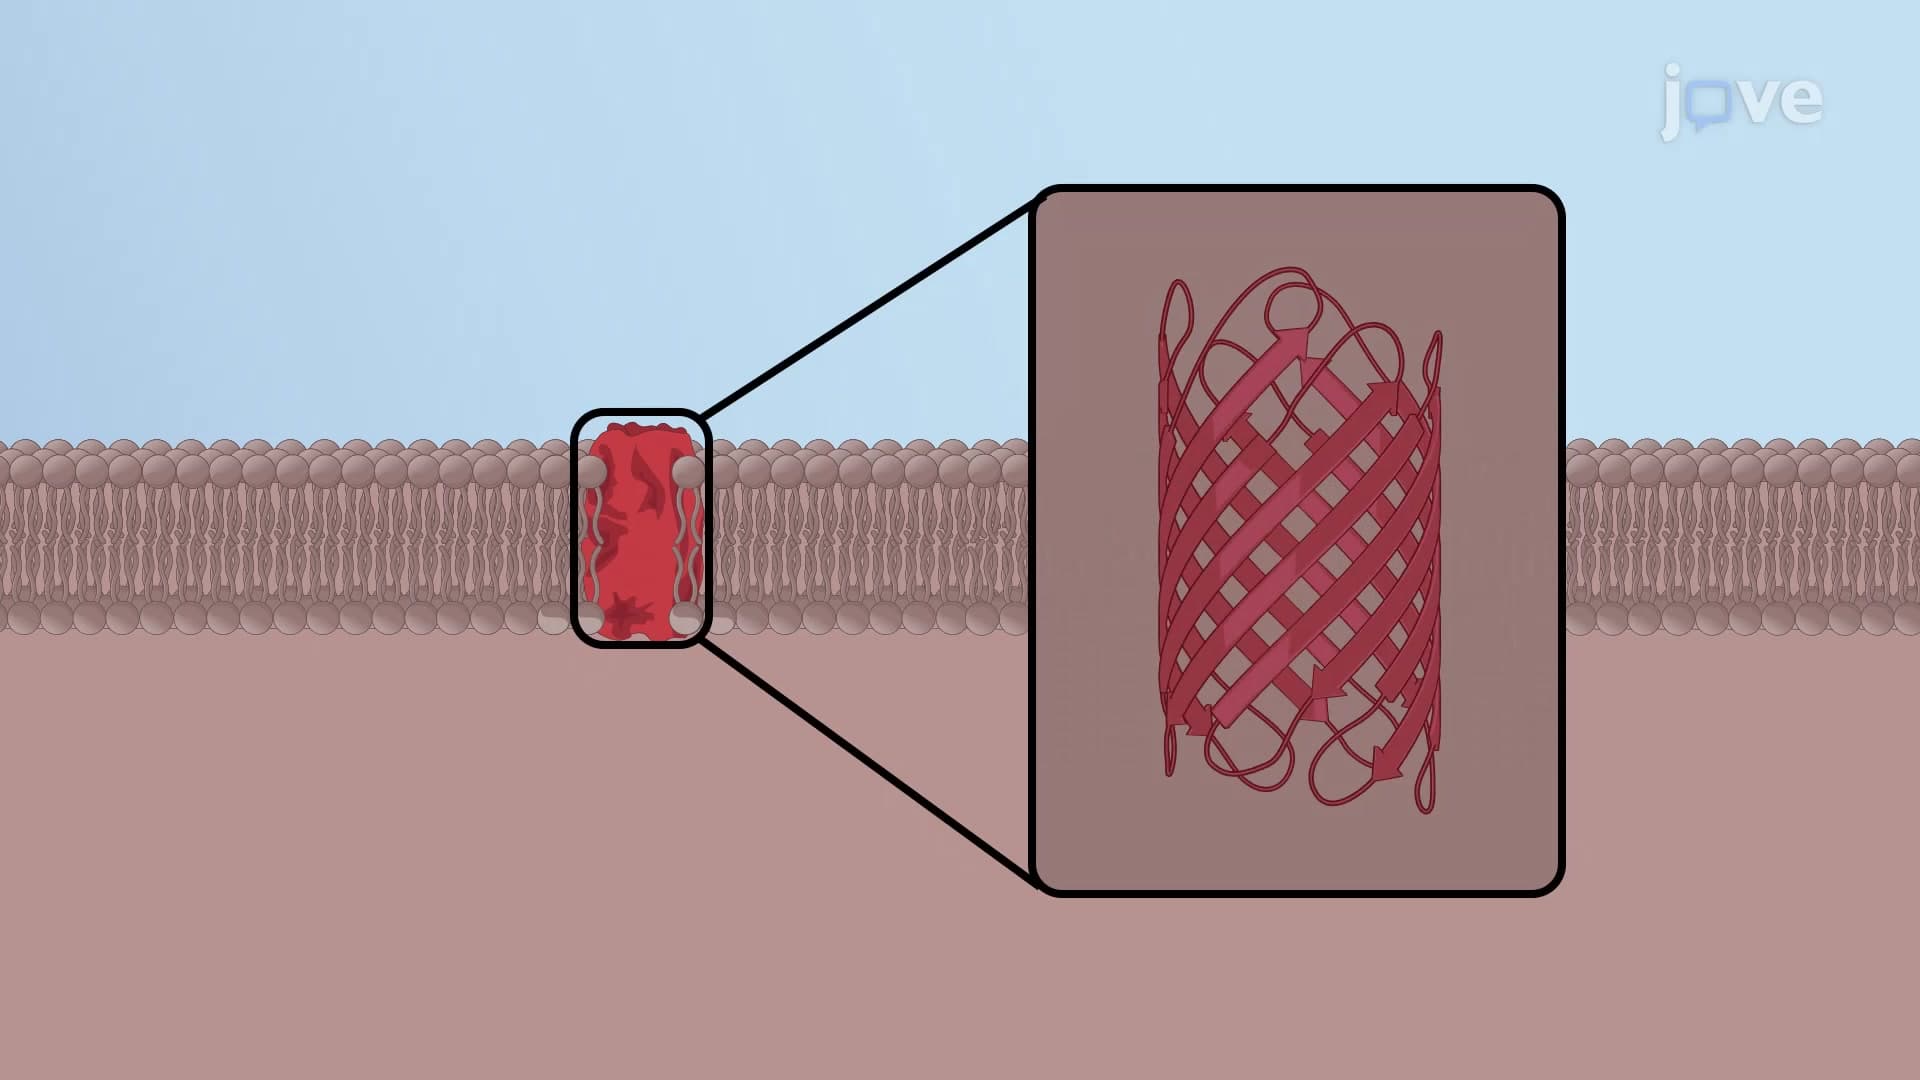
Structure of Porins
 01:45
Tail-anchoring of Proteins in the ER Membrane